


Abstract
Severe acute respiratory syndrome coronavirus 2 (SARS-CoV-2), a novel human coronavirus, which has triggered a global pandemic of the coronavirus infectious disease 2019 (COVID-19). Outbreaks of emerging infectious diseases continue to challenge human health worldwide. The virus conquers human cells through the angiotensin-converting enzyme 2 receptor-driven pathway by mostly targeting the human respiratory tract. Quercetin is a natural flavonoid widely represented in the plant kingdom. Cumulative evidence has demonstrated that quercetin and its derivatives have various pharmacological properties including anti-cancer, anti-hypertension, anti-hyperlipidemia, anti-hyperglycemia, anti-microbial, antiviral, neuroprotective, and cardio-protective effects, because it is a potential treatment for severe inflammation and acute respiratory distress syndrome. Furthermore, it is the main life-threatening condition in patients with COVID-19. This article provides a comprehensive review of the primary literature on the predictable effectiveness of quercetin and its derivatives docked to multi-target of SARS-CoV-2 and host cells via in silico and some of validation through in vitro, in vivo, and clinically to fight SARS-CoV-2 infections, contribute to the reduction of inflammation, which suggests the preventive and therapeutic latency of quercetin and its derived-products against COVID-19 pandemic, multisystem inflammatory syndromes (MIS), and long-COVID.
Keywords: Quercetin, COVID-19, In silico, Long-COVID, MIS
Graphical abstract
Therapeutic Implications of Quercetin and its Derived-products in COVID-19 Protection and Prophylactic.
1. Introduction
The first case of severe acute respiratory syndrome coronavirus 2 (SARS-CoV-2) was reported clinically and identified in Wuhan City, China, in December 2019. This was followed by a rapidly growing outbreak and transmission worldwide, which caused the most serious epidemic in human history (https://covid19.who.int/). At the end of 2019, the disease associated with SARS-CoV-2 was officially named coronavirus disease 2019 (COVID-19) by the World Health Organization (WHO) [1]. Based on data recorded by the WHO regarding the COVID-19 pandemic that has spread to all countries and regions, over 774 million people were infected and more than 7.03 million deaths occurred before Feb 2024 (https://covid19.who.int/), with both large between- and within-country variations in COVID-19 death rates. Infections result in a broad spectrum of clinical disease severity, which has led to devastating health crises worldwide [2]. First, SARS-CoV2 binds to a serine protease, which acts as a receptor for the ectoenzyme angiotensin-converting enzyme 2 (ACE2), whereas another transmembrane serine protease 2 (TMPRSS2) is necessary for priming the viral spike protein required to enter the cell, leading to COVID-19 [3,4]. This severity originates from the immune response of the host, particularly the release of inflammatory cytokines. Some of the consequences of severe inflammation and cytokine storms include acute lung injury, acute respiratory distress syndrome (ARDS), and multiple organ dysfunction syndromes.
Currently, no treatment exists to counter this highly contagious disease with high viral variants; some vaccines (AstraZeneca AZ, BioNTech BNT, Moderna) and antiviral agents (Remdesivir, Paxlovid (Pfizer), or Molnupiravir (Merck)) have been used for emergency authorization use (EAU), as stipulated by the WHO or Food and Drug Administration (FDA). At present, the WHO and all countries have announced the end of the emergency phase of the COVID-19 pandemic for more than one year, but the new mutant variants of SARS-CoV-2 continue to spread and cause reinfections in several million people [5], and the overall reinfection rate in Asian populations is more than 9.5 % per year [6]. Thus, there is an urgent need to find a cure for the disease, and global efforts have been directed toward developing SARS-CoV-2-specific antivirals and immunomodulators. Notably, potential and effective phytochemicals (phytoconstituents, phytomolecules, and phytocompounds), which act as phytomedicines, have been investigated to meet global demands [7]. In this review, we focus on recent investigations of the interactions of quercetin (or quercetin derivatives) with hosts or viral targets that interfere with the viral infective cycle of SARS-CoV-2. We collate and organize the most published results of the effects quercetin and quercetin derivatives on SARS-CoV-2 based on in-silico simulations, in-vitro and in-vivo tests, and clinical trials to reveal the therapeutic value of these molecules. Such promising studies may stimulate the use of quercetin, quercetin derivatives, and other phytocompounds in preventive/cotherapeutic strategies to combat the COVID-19 pandemic.
2. The viral structures and proteins of SARS-Co-2
SARS-CoV-2 is a single positive-stranded ribonucleic acid (RNA) virus, whose mutation rate is higher than that of DNA viruses [8]. To date, recorded variants of SARS-CoV-2 are over 1000, including the major epidemic variants, Beta, Delta, and Omicron [9] (https://www.who.int/activities/tracking-SARS-CoV-2-variants/tracking-SARS-CoV-2-variants). The diameter of SARS-CoV-2 viral particles is approximately 100 nm, and SARS-CoV-2 is enclosed by a phospholipid bilayer envelope with three integral membrane proteins: spike (S), envelope (E), and membrane (M) proteins [10] (Fig. 1). Within the envelope of the SARS-CoV-2 viral particles, there are single positive-stranded viral RNA genomes with a length of approximately 30 kb; these genomes bind to nucleocapsid (N) proteins to form tight spiral-folding structures, such as helical ribonucleoproteins (RNPs) [1,11]. Stable interactions between RNPs and M-proteins are involved in strengthening the coronavirus assemblage and may protect the virus against environmental and physical challenges [11,12]. E-proteins are the smallest virion structural proteins, and the five E-proteins form a pentamer transmembrane ion channel, also known as an E channel [13,14]. The S-protein comprises three S1–S2 heterodimers. The receptor binding domain (RBD) located on the head of S1 can bind to the host cellular receptor ACE2 to trigger viral infections, followed by fusion of the membrane between the viral envelope and host cell [3,4,15].
Fig. 1.

The graphic portrays the genome of SARS-CoV-2.
The genome of SARS-CoV-2 comprises several open reading frames (ORFs) separated by transcriptional regulatory sequences (TRSs) (Fig. 1). The 5′ two-thirds of the SARS-CoV-2 genome is ORF1. Genomic ORF1 comprises ORF1a and ORF1b. ORF1 can be translated into three polyproteins (PPs): PP1a, PP1b, and PP1ab. The PPs translated from ORF1 are further subjected to post-translational cleavage by two viral proteases into 16 non-structural proteins (nsp1–nsp16). These two viral proteases are papain-like proteinase (PLpro) and 3-chymotrypsin-like protease (3CLpro), also known as the main proteases (Mpro). The first three cleavage sites of PP1a or PP1ab are cleaved by PLpro to produce nsp1–nsp3, and the other post-translational cleavage of PP is achieved by 3CLpro to produce nsp4–nsp16 [8,16]. nsp1 binds with type-I interferon (IFN) to affect and inhibit virus-induced IFN-β production, wherein the host immune response is inhibited to erect the viral infected cell [17]. nsp2 participates in the viral genomic replication and transcription of SARS-CoV-2 and interacts with nsp7 and nsp8 to form a replication-transcription complex (RTC). nsp3 is the largest non-structural protein (nsp) of SARS-CoV-2 with PLpro activity, and is a virus-encoded protease that acts on the post-translational cleavage to produce nsp1, nsp2, and nsp3 of SARS-CoV-2 [8,18]. nsp4 is a transmembrane scaffold protein that interacts with nsp3 and nsp6 to promote the formation of double-membrane vesicles (DMVs) during viral replication [19]. nsp5 is 3CLpro (or Mpro), and serves as a post-translational cleavage site for the production of most SARS-CoV-2 nsps [20]. nsp7 and nsp8 comprise the accessory cofactors of the RNA-dependent RNA polymerase (RdRp), and nsp9 serves as a single-stranded RNA-binding protein that plays a role in viral genome reproduction [[21], [22], [23]]. nsp10 is a zinc finger protein that binds to non-specific RNA to serve as a cofactor for nsp14 and nsp16 [24,25]. nsp11 is an accessory remnant polypeptide of PP1 formed by the post-translational cleavage of only 13 amino acid residues [26]. nsp12 is an RdRp, namely, the core protein that binds to its essential cofactors nsp7 and nsp8 to form the RTC [27]. nsp13 catalyzes the unwinding of duplex oligonucleotides into single strands in a nucleotide-binding pocket (NTP)-dependent manner [28]. nsp14 is a bifunctional enzyme of SARS-CoV-2 with two active domains: the N-terminal exonuclease (ExoN) and C-terminal guanine-N7 methyltransferase (N7-MTase) domains. The ExoN of nsp14 is important for proofreading, elongating RNA, and excising mismatched bases during viral replication and transcription, and nsp10 serves as a cofactor to stimulate ExoN activity [29]. N7-MTase of nsp14 is an S-adenosylmethionine-dependent methyltransferase that catalyzes genomic RNA cap synthesis [30,31]. The C-terminal domain of nsp15 acts as a nidoviral RNA uridylate-specific endoribonuclease (NendoU) that cuts single-stranded RNA to evade viral detection by the host's defense system [22,32,33]. nsp16 of SARS-CoV-2 is a S-adenosyl-l-methionine (SAM)-dependent MTase that methylates the RNA cap at ribose 2′-O positions (2′-O-MTase). nsp16 binds with its cofactor nsp10 modify the 5′-end of viral RNAs to simulate the host mRNA structure, which is imperative for viral genomic replication and expression, and aids in the viral immune evasion of coronavirus [34,35]. All the viral functional proteins of SARS-CoV-2 may serve as antiviral therapeutic targets for the development of new pharmaceuticals.
3. The significance of quercetin against COVID-19
Quercetin (3,30,40,5,7-pentahydroxy-2-phenylchromen-4-one) is a major component of the flavonoid subclass. In particular, it is found in many common fruits and vegetables. Among vegetables, high levels of quercetin have been found in red leaf lettuce (Lactuca sativa L.; 10.3–30.6 mg/100 g), asparagus (Asparagus officinalis L.; 23.6 mg/100 g), Romaine lettuce (Lactuca sativa L.; 12 mg/100 g), and onions (Allium cepa L.; 11–41.9 mg/100 g); among fruits, apples (2.3 mg/100 g), cherries (1.2 mg/100 g), and blueberries (3.58 mg/100 g) have high contents of quercetin [36,37]. Quercetin has been found to possess multiple biological activities, including anti-allergic, anti-inflammatory, anti-oxidative, and anti-aging properties [38,39]. Notably, the potential pharmacological properties of quercetin are as follows: antiallergic, anti-diabetic, anticancer, promotion of anti-oxidant activities [[40], [41], [42]], anti-inflammatory, antimicrobial, immunoprotective effects [43], neuroprotective properties, prevention of chronic diseases [44], anti-obesity, antineoplastic, inhibition of lipid peroxidation, platelet aggregation, capillary permeability, and stimulation of mitochondrial biogenesis [[45], [46], [47]]. Similar to most other polyphenols, quercetin has a low rate of oral absorption, and its clinical use is considered to be of modest utility. Based on the low bioavailability of quercetin, innovative drug delivery strategies, such as quercetin polymeric micelles, quercetin nanoparticles, glucan-quercetin conjugates, and quercetin-loaded muco-adhesive nanoemulsions, have been suggested to increase the bioavailability of quercetin and facilitate novel therapeutic approaches [2,48]. Quercetin may be more applicable in new preparations for human healthcare after improvements in its solubility and bioavailability [49,50].
Quercetin is a nuclear factor erythroid-derived 2-like 2 (Nrf2)-interacting nutrient that reduces insulin resistance, endothelial damage, lung injury, and cytokine storms. Quercetin and some quercetin derivatives also play a role in certain mechanisms, such as the mammalian target of rapamycin (mTOR), peroxisome proliferator-activated receptor γ (PPARγ), nuclear factor kappa B (NF-κB), extracellular signal-regulated kinases (ERK), and elongation initiation factor 2α (eIF2α). Some quercetin derivatives are important in mitigating the severity of COVID-19 by acting through endoplasmic reticulum stress or the ACE-Angiotensin–II–AT1 receptor axis (AT1R) pathway [51,52], which is an Nrf2-interacting nutrient that also interacts with TRPA1 and/or TRPV1 [53]. First, Nrf2 agonists abolish the replication of SARS-CoV-2 in lung cells, and quercetin is a potent Nrf2 agonist. Second, quercetin exhibits antiviral activity against several zoonotic coronaviruses, including SARS-CoV-2, by hindering the entry of virions into host cells. Third, inflammasomes are cytosolic multi-protein complexes that generate active forms of cytokines IL-1β and IL-18. Quercetin suppresses the activation or inhibition of the nod-like receptor (NLR) family pyrin domain-containing 3 (NLRP3) inflammasomes by affecting mediators, such as thioredoxin-interacting protein, sirtuin 1, and NRF2 [44]. Inflammatory pathways are activated by inflammasome, and NF-κB and interleukin-6 signals provoke the cytokine release syndrome, which promotes ARDS in COVID-19 patients, and Quercetin may inhibit these pro-inflammatory signals [54]. Fourth, patients with COVID-19 can develop thrombosis, and quercetin alleviates coagulation abnormalities by inhibiting plasma protein disulfide isomerase [55]. Quercetin and some quercetin derivatives have multi-target binding abilities with several viral proteins of SARS-CoV-2, which play an indispensable role in facilitating viral replication (Fig. 3). Quercetin and its derivatives target the aforementioned target proteins to block viral replication and transcription, which may be used alone or in combination with other treatments to enhance therapeutic efficacy [56].
Fig. 3.

Quercetin and its derivatives docked on various domain or segment proteins of SRAS-CoV-2. Red indicates the dominated compounds. The black T bar present suppressed compounds. (For interpretation of the references to colour in this figure legend, the reader is referred to the Web version of this article.)
Multiple variants of SARS-CoV-2 have been found, raising questions regarding the efficacy of different lines of treatment, such as vaccines and antiviral drugs. Notably, many small molecules extracted and isolated from plants are known for their antiviral effects [57,58], whereas no antiviral drugs from plants have been approved thus far. Evaluating the safety and effectiveness of herbal medicines is difficult because of their adverse effects and herb-drug interactions [59,60]. To explore appropriate prevention/treatment measures, antibacterial, antifungal, and antiviral properties were verified in mammalian HEK293T cells [61], indicating that quercetin and some quercetin derivatives with immunomodulatory activity play a pertinent role in reducing inflammation and thwarting serious chronic diseases. This analysis indicated that although positive data were obtained, they were still insufficient to recommend quercetin and quercetin derivatives as potential immunomodulatory agents against COVID-19. Additionally, an essential enzyme in the SARS-CoV-2 replication machinery, namely, RdRp, was targeted in a virtual screening assay using a set of 1664 FDA-approved drugs, including botanical and synthetic derivatives. Notably, a set of 22 drugs with high docking scores may be candidates as inhibitors of RdRp of SARS-CoV-2 [62]. Among these candidates, quercetin and several phytocompounds have been approved by the FDA for use as anti-oxidants, cell-protective agents, general tonics, immune stimulants, and other miscellaneous systemic or topical applications.
The epidemiological burden of COVID-19 is a healthcare challenge worldwide as it tested the limits of medical capacity and preventive strategies and methods. Based on the identification of relevant key structure-activity relationships (SARs), analogs of quercetin and its derivatives have superior anti-inflammatory, anti-oxidative, and antiviral effects compared with the original molecules. These approaches highlight the mechanisms that govern their anti-inflammatory, anti-oxidant, and antiviral activities [63]. One strategy could be to enhance the antiviral immune response through a nutritious diet, including quercetin and quercetin derivatives isolated from natural extracts, to minimize the risk of infection (Fig. 2). Through a critical analysis of the literature, quercetin and its derivatives were found to act concurrently on inflammation and viral and oxidative stress, which may alleviate life-threatening diseases. Considering the increasing threat of COVID-19, the therapeutic efficacy of existing antiviral molecules in edible fruits should be evaluated; their potential anti-oxidant, anti-inflammatory, and immunomodulatory effects could help determine prophylactic and adjuvant therapies [64].
Fig. 2.

The illustration depicts the structure of quercetin and its derivatives. All share the same core structure.
In this review, we collected literature and subsequently analyzed and discussed the current state of knowledge regarding the antiviral properties of quercetin and its derivatives, wherein the underlying mechanisms of action were focused on major human viruses belonging to the family Coronaviridae. We collected literature from various data sources, such as Google Scholar, Medline, Scopus, and PubMed. The purposes of molecular docking, in-silico, and virtual screening (simulation) were separated into several aspects: the option of target (multi-target), compounds (multi-ligand), and signal transduction (multi-pathways) to show evidence of crosstalk and other relevant mechanisms (Fig. 3).
4. In silico investigations of quercetin and its derivatives on COVID-19
4.1. In silico of quercetin on targets of SARS-CoV-2
Molecular docking demonstrated multiple binding sites or different affinity scores for the same ligand/target protein and various programs were used or conditions set in many studies. However, the results from in silico studies provide predictive information on molecular interactions between ligands and target proteins along with the real effects still needed for further validation from in vitro, in vivo, and in clinical studies. There were more than 100 studies through Jan 2024 that had investigated the effects or medicinal potential of quercetin and its derivatives on COVID-19 pandemic based on molecular docking results. Notwithstanding, the docking evidence showed quercetin interact with different viral proteins of SARS-CoV-2, which affects viral infections and replication. It also acts on several host-based proteins as early as possible to attenuate infections and symptoms for COVID-19.
The genomic expressions of ORF-1 in SARS-CoV-2 are translated into polyproteins and the cleavage into several functional proteins (non-structural proteins, nsp1-nsp16) by two major viral proteinases, 3CLpro and PLpro (2), and in fact 3CLpro of SARS-CoV-2 is also called Mpro. The application of multi-target approach is employed for the termination of the viral life cycle. To explore the bioactive compounds in honey, the results presented quercetin as acting and forming hydrogen bonds with Tyr54, Leu141, Ser144, His163, and Gln189 residues for active binding sites in Mpro [65]. For screening bioactive compounds from Ayurvedic medicinal plants, this study conformed quercetin to form a hydrogen bond within the active site of Mpro [56]. A molecular docking study on the bioactive constituents from Cressa cretica revealed quercetin forms hydrogen bonds within the binding sites of Mpro at Thr24, Thr26, Asn28, His41, Asn119, Asn142, and Gln189 residues [66]. Another study showed the quercetin can form hydrogen bond interactions with the activation site and dimerization site of Mpro at Glu288, Asp289, and glu290 residues, as well as form a π-Alkyl interaction with regulatory site at Leu286 [67]. The results demonstrated that quercetin interacts with Mpro [[68], [69], [70], [71]], major predicted binding sites at three amino acid residues Asp48, Met49, and Asp187 of Mpro [69]. The in silico predicted study revealed quercetin binds with Mpro at Tyr237, Asn238, Gly275, Met276, and Gly278 residues [72]. For example, (quercetin/Mpro) interactions at amino acid residues at Asn142, Gly143, Ser144, Leu141, Cys145, His41. and Thr26 [73]. In another study, the substrate binding pocket of Mpro binds by rutin, quercetin, and kaempferol at the catalytic residues of His41 and Cys145 with high affinity (10−5-10−6 M) [74]. The results from the above studies showed that even with similar docking scores or binding energy, but the interacting residues for quercetin on Mpro only few matched from various experiments. Additionally, A molecular docking studies on the investigation of inhibitor for SARS-CoV-2 showed that quercetin also can form five hydrogen bond interactions with PLpro at AspP77, Arg83, Thr75, and Asn157 amino acid residues [75]. Such massively divergent results further indicated that for in silico outcomes, in particular, for Mpro were significantly affected by target protein model choice, molecular docking program used, operational and conditional setting, bias or training of researchers, and all in silico results need further validation from either direct evidence from a binding assay or indirect approach by in vitro or in vivo studies for further confirmation. These will be discussed in another section of this paper.
Another study illustrated that quercetin interacts with RBD of S-protein and also forms hydrogen bonds with the s2 domain of S-protein at Ala1056, Pro1075, Gly1059, His1058, Ser730, Met731, Lys733, and Leu861 residues [76]. Quercetin is a major bioactive component for several Ayurveda natural products, molecular docking results showed quercetin acts on S-protein by forming hydrogen bonds with Gln314, Ser316, Asn317, Asn764, Arg765, and Thr768 residues with a binding affinity of −14.48 kcal/mol [77]. Quercetin forms three conventional hydrogen bonds with amino acid residues at Gly496, Asn501, and Tyr505 in S-protein (PDB: 6LZG) of SARS-CoV-2, the pi-pi interaction at Tyr453, and pi donor hydrogen bond at Arg403. In addition, quercetin generates van der Waals interactions with Gln506, Phe497, Tyr495, Gln493, Lys417, Glu406, and Leu155 [67].
Nsp13 is a functional helicase of SARS-CoV-2 that provides the 5′-triphosphatase and RNA helicase activities [78]. In silico simulations show quercetin simultaneously docks with two major functional pockets of SARS-CoV-2 nsp13: the NTP and 5′-RNA-binding sites, which interrupts the viral RNA unwinding and ATPase activity; and the in vitro enzymatic activity test confirmed the potential of quercetin as candidate as for a powerful inhibitor of nsp13 [79]. SARS-CoV-2 nsp15, an endoribonuclease, is a crucial viral protein for the mechanistic action of viral infection, replication, and transcription; and it constrains production of the host, IFN-β [80]. The results presented show that quercetin forms several hydrogen bonds with nsp15 at four amino acid residues Lys290, His235, His250, and Glu340 [73].
In silico evidence showed that quercetin had a high binding affinity with nsp16 by forming hydrogen bonds or π-anion interactions with four amino acid residues at Asp130, Gly73, Leu100, and Asp99 [81]. In general, intracellular RNA will be degraded by RNase of eukaryotic cells for SARS-CoV-2 survival, while the modification of cap methylation at the 5′end of SARS-CoV-2 RNA genome plays a vital role in its prevention as it is degraded by the host intracellular protection mechanisms. The methylation on the 5′-cap of SARS-CoV-2 RNA genome assumes key roles on the viral replication and immune evasion, which is catalyzed by nsp14 (guanine-N7 methyltransferase) and nsp16 (2′-O-ribose methyltransferase) [30]. The RNA 5′ end cap modification of SARS-CoV-2 were carried by the nsp10/nsp16 RNA cap 2′-O-Methyltransferase [25]. Additionally, quercetin acts as the anti-cap methyltransferase inhibitor on the enzymatic active site of nsp16 at Tyr47, Gly71, Asp114, Phe149, and Asp130 residues via molecular docking [82] (Table 1).
Table 1.
Quercetin and its derivatives docking with targets of host and SARS-CoV-2.
| Ligand | Host/virus | Target | PDB ID | binding site | Reference |
|---|---|---|---|---|---|
| Quercetin | Host | ACE2 | 1R42 | Lys745, Tyr613, His493, Asp609 | [165] |
| Tyr385, Phe390, Arg393, Asp350 | [77] | ||||
| 1R4L | Arg273, Phe274, His345, Pro346, Thr347, Ala348, Thr371, His374, Glu375, His378, Glu406, Phe504, His505, Tyr515, Arg518 | [97] | |||
| STAT1 | 2KA6 | Met28, Asn93 | [166] | ||
| TNF | 5M2J | Phe144, Leu142, Ala22, Gly24 | |||
| GRP78 | 5E84 | Glu427, Gly430, Thr458, Lys460 | [167] | ||
| IL-6 | 1ALU | Arg30, Arg 179, Leu33, Leu178, Arg182 | [126] | ||
| n.a. | Glu127, Gln130, Glu137, Arg141 | [106] | |||
| IL-1α | n.a. | Asn92, Glu149, Lys150, Tyr153, Tyr175 | |||
| TNF-α | n.a. | Leu113, Gln201 | |||
| TMPRSS2 | UniProt O15393 | Gly383, Gly385, Asn433, Asp435, Asn398, Gly259, Ala400 | [99] | ||
| TMPRSS2 | 7MEQ | Lys390, Gln438, Ser436, Cys465, Trp461 Cys437, Gly464, Cys465 | [100] | ||
| FOS | 1FOS | Ser154, Arg155, Ser278, Arg279, Asn156 | [107] | ||
| p38/MAPK | 5XYY | Lys53, Thr106, His107, Met109, Asp112, Asp168 | [104] | ||
| JNK2 | 3E7O | Glu109, Met111, Gln117 | |||
| SARS-CoV-2 | Mpro (nsp5) | 3IWM | Tyr237, Asn238, Gly275, Met276, Gly278 | [72] | |
| 6LU7 | Leu141, Gly143, Ser144, Cys145, His163, Met165, Arg188 |
[88] | |||
| 2A5I | Tyr54, Glu55, Asp187 | [168] | |||
| 4XFQ | Ala26, Cys144, Ile140, Asn141, His162 | [169] | |||
| 5R84 | Arg298 | [68] | |||
| 5RFS | Thr190, His41, Met49, His164, Met165, Glu166, Pro168, Gln192 | [170] | |||
| 6LU7 | His164, His41, Cys44, Met49, Tyr54, Cys85, Cys145, Met165, Gly174, Thr175, Phe181, Phe185, Val186, Asp187, Arg188, Gln189, Gln192 | [56] | |||
| Thr24, Thr26, Asn28, His41, Asn119, Asn142, Gln189 | [66] | ||||
| Glu166, Gln189, Gln192 | [132] | ||||
| Arg131, Lys137, Thr199, Tyr239, Leu286, Asp289 | [120] | ||||
| Leu141, Gly143, Ser144, Glu166 | [167] | ||||
| Thr26, His41, Asn142, Leu141, Gly143, Ser144, Cys145 | [73] | ||||
| Tyr54, Leu141, Ser144, His163, Gln189 | [65] | ||||
| Tyr54, Glu166, Gln192, Thr190, Asp187, His41, Met165, Leu167, Arg188, Gln189, Pro168 | [171] | ||||
| Thr26 | [113] | ||||
| Gly143, Glu166, Arg188, Glu189 | [172] | ||||
| 6YB7 | Thr199, Glu288, Glu290, A sp289, Leu286 | [67] | |||
| 6Y2E, 6Y2F | Glu166, Leu141, His41, Cys145 | [118] | |||
| 6Y84 | Gln127, Cys128, Lys137, Asp289, Glu290 | [145] | |||
| 6W9C | Asp157 | [173] | |||
| Gln30 | [168] | ||||
| 2GTB | Thr111, Asp153 | ||||
| 6LU7, 5C3N | Leu50, Gln189 | [91] | |||
| S-protein | 6LZG | Arg454, Arg457, Lys458, Asp467, Ser469, Glu471 | [88] | ||
| 6LZG | Gly496, Asn501, Tyr505, Tyr453, Arg403, Gln506, Phe497, Tyr495, Gln493, Lys417, Glu406, Leu155 | [67] | |||
| 6M17 | Ser349, Leu441, Asp442, Asn448, Asn450, Arg509 | [167] | |||
| 6VXX | Gln314, Ser316, Thr768, Asn317, Asn764, Arg765 | [77] | |||
| Asp88, Asp198, Ile233, Ile235 | [168] | ||||
| 6VW1 | Thr445, Ile446 | [113] | |||
| 6VYB | Ser730, Met731, Lys733, Leu861, Ala1056, Pro1057, His1058, Gly1059, Val860, Pro863, Asp867, Met730, Ile870, | [76] | |||
| 6VSB | Thr549, Asp745, Asn978, Arg1000 | [75] | |||
| S-protein (Closed) | 6VXX | Tyr741 | |||
| S-protein (Open) | 6YVB | Tr549, Asn978, Gly744, Arg1000, Thr573, Met740, Tyr741 | |||
| nsp16 | 6YZ1 | Gly73, Leu100, Asp130, Glu71, Ala72, Ser74, Asp75, Ser98, Asp99, Leu100, Asp114, Cys115, Met131, Tyr132, Asp133, Phe149 | [81] | ||
| 6WJT, 6WKQ | Tyr47, Gly71, Asp114, Phe149, Asp130 | [82] | |||
| RdRp (nsp12) | 6M71 | Glu350, Asn628, Val315, Arg349, Pro461, Pro677 | [120] | ||
| 6NUS | Glu350, Pro323, Asn628, Val675 | [75] | |||
| 7BTF, 6M71, 6NUR | Tyr619, Cys622, Asp623, Asp761, Ser841 | [168] | |||
| 6W9Q | Leu45, Thr109 | ||||
| nsp9 | 6W4B | Pro58, Thr68 | |||
| nsp15 | 6VWW | Lys290, His235, His250, Glu340 | [73] | ||
| 6W01 | Leu347, Lys346, Asn279, Cys292 | [174] | |||
| PLpro (nsp3) | 3E9S | Lys158, Asp165, Thr169 | [168] | ||
| S-protein/ACE2 | 6M0J | Ala348, Gly352, Asp382, Phe390, Arg393, Asn394, His401 | [120] | ||
| Rutin | Host | ACE2 | 1R4L | Asn149, Met270, His345, Lys363, Thr445, Tyr127, Leu144, Glu145, Glu150, Met152, Ala153, Asp269, Trp271, Phe274, Thr276, Cys344, Pro346, Met360, Cys361, Asp367, Asp368, Thr371, Leu503, Phe504 | [97] |
| IRF3 | 1QWT | Leu196, Gly199, Glu201, Pro223, Glu224, Arg276, Gly278 | [102] | ||
| SARS-CoV-2 | Mpro (nsp5) | 5RFS | Thr25, Thr24, Gly143, His164, Asn142, Thr26, Cys145, Arg188, Met165, Asp187, Met49, Gln189, Glu166 | [170] | |
| 6LU7 | Asn142, Thr190, His41, Met49, Glu166, Asp187, Arg188, Gln189 | [70] | |||
| His164, Gln192, Asp187, Glu166, Leu141, Pro168, Ala191, Cys44, Pro168 | [175] | ||||
| 6Y2E, 6Y2F | His41, Cys145, Glu166, Leu141 | [118] | |||
| quercetin-3-O-glucoside | SARS-CoV-2 | PLpro (nsp3) | 4OVZ | His74, Arg83, Tyr155, Asn157, His176 | [75] |
| Mpro (nsp5) | 6LU7 | Leu141, His163, Met 165 | |||
| RdRp (nsp12) | 6NUS | Ala125, His133 | |||
| S-protein | 6VSB | Phe970, Arg995, Thr998 | |||
| S-protein (Closed) | 6VXX | Glu988 | |||
| S-protein (Open) | 6YVB | Thr998, Arg995, Asp994 | |||
| Quercetin 3-O-(6″-galloyl)-β-d-galactopyranoside | Host | IRF3 | 1QWT | Glu201, Thr219, Ile220, Ser221, Glu293, Ile395, Asp392, Ser398 | [102] |
| Quercetin-3-O-galactosyl-rhamnosyl-glucoside | SARS-CoV-2 | RBD of S-protein | 6M0J | Glu406, Gln493, Gly496, Gln498, Gly502, Tyr505 | [110] |
| Nsp15 | 6W01 | Gln245, Val339, Glu340, Trp333, Met219, Ala232, Gly230, Gly247, Gly248 | |||
| Quercetin-3-rutinoside-7-glucoside | SARS-CoV-2 | Mpro (nsp5) | 5RFS | Thr24, Thr25, Thr26, Ser46, Asn142, His164, Glu166, Gly143, Leu27, Thr45, Met165, His41, Met49, Arg188, Leu167, Pro168 | [106] |
| Bioquercetin (Quercetin 3-O-robinobioside) | SARS-CoV-2 | Mpro (nsp5) | 6LU7, 5C3N | Pro168, Gln189 | [91] |
| Quercetin-3-D-xyloside | SARS-CoV-2 | Mpro (nsp5) | 6LU7 | His41, Leu141, Asn142, Ser144, His163, Glu166, Thr190, Met165, Pro168, Asp187, Arg188, Gln189 | [70] |
| Quercetin 3-O-α-l-arabinopyranoside | SARS-CoV-2 | Tyr53, His163, Glu166, Asp187, His41, Met49, Phe140, Leu141, Arg188, Gln189 | |||
| Quercetin 3-O-(6″-O-malonyl)-β-D-glucoside | SARS-CoV-2 | Leu141, Ser144, Glu166, His41, Met49, Asn142, Cys145, Met165, Asp187, Arg188, Gln189 | |||
| Quercetin 3-β-D-glucoside | SARS-CoV-2 | Met49, Pro52, Asn142, Glu166, Leu167, Thr169, Gln189, Met49, Pro52 | [111] | ||
| 8-(ptolylselenyl)-quercetin | SARS-CoV-2 | Mpro (nsp5) | 6Y2E, 6Y2F | Gln189, His41, Cys145, | [117] |
| quercetin-3-rhamnoside | SARS-CoV-2 | Mpro (nsp5) | 6Y2E | Lys5, Ala7, Gln127, Lys137, Glu290 | [151] |
| Isoquercetin | SARS-CoV-2 | Mpro (nsp5) | 5RFS | Glu166, Asn146, His41, Gly143, Leu27, Thr25, Cys44, Val42, Met49, Cys145, Met165, Arg188, Gln189, Thr190, Pro168, Leu167, Leu141, Ser144, His163, Phe140 | [106] |
| S-protein | 6VSB | Phe347, Val350, Asp442, Phe497, Arg509, Arg346, Ala348, Val401, Ser349, Gln493, Tyr495, Tyr351, Ser494, Gln498, Pro499, Ser443 |
|||
| RdRp (nsp12) | 6M71 | Trp617, Asp618, Tyr619, Asp760, Lys798, Pro620, Lys621, Cys622, Cys799, Trp800, Gly616, Ala762, Asp761, Glu811, Ser814, Ser759 |
|||
| Quercetin 3-O-Neohesperidoside | SARS-CoV-2 | Mpro (nsp5) | 6LU7 | His41, Gly143, Cys145, Gln189, Thr190 | [85] |
| quercetin 3-O-arabinoside 7-O-rhamnoside | SARS-CoV-2 | PLpro (nsp3) | 4M0W | Lys27, Gln41, Arg42, Arg72, Arg74, Asn157, Lys158, Glu162, His176 | [87] |
| quercetin-3-neohesperidoside-7-rhamnoside | SARS-CoV-2 | Mpro (nsp5) | 6LU7 | Asn133, Thr169, Ala194, Asp197, Thr199, Asn238, Leu287 | |
| quercetin 3-[rhamnosyl-(1- > 2)-alpha-l-arabinopyranoside] | SARS-CoV-2 | S-protein | 6LZG | Ala348, Tyr385, Asn394, Glu398, Arg514 | |
| Quercetin-3-O-sophoroside | SARS-CoV-2 | Mpro (nsp5) | 6LU7 | Asn119, Asn142, Gly143, Cys145, His164, Met165, Glu166, Asp187, Gln189, | [144] |
| RdRp with RNA | 7BV2 | Asp452, Arg555, Thr556, Lys621, Cys622, Asp623, Ser682, | |||
| RdRp without RNA | 7BV2 | Tyr619, Asp760, Ser759, Arg553, Arg555, Thr556, Val557, Ser682, Ser681, Thr680, Arg624, Thr687, Cys622, Lys621, Asp623 | |||
| Nsp14 ExoN | 5C8S | Asp90, Val91, Glu92, Asn104, Pro141, Gln145, Ala178, Phe190, Glu191, Leu235, Asn252, His268, Asp273, | |||
| Nsp14 N7-MTase |
5C8S | Cys309, Arg310, Gln313, Gly333, Asn334, Pro335, Lys336, Ile338, Lys339, Trp385, Cys387, Phe401 | |||
| Nsp15 | 6WLC | His234, Gly246, Gly247, His249, Ser293, Trp332, Glu339, Thr340, Tyr342, Pro343, Lys344 | |||
| Nsp16 (2′-O-MTase) | 6WVN | Asn29, Tyr30, Lys46, Gly71, Ala72, Gly73, Ser74, Asp75, Asp99, Leu100, Asp130, Met131, Tyr132, Pro134, Lys170, Glu203 | |||
| PLpro (nsp3) | 6WUU | Lys157, Gly160, Glu161, Leu162, Leu199, Met206, Tyr207, Met208, Gly209, Gln221, Ile222, Tyr268, Gln269 | |||
| E protein | Epro.pdb | Phe23, Phe26, Leu27, Leu28, Val29, Thr30, Leu31, Ala32, Thr35, Cys43, Ile46, Val47, Leu51 | |||
| Nsp13 ADP site | 6JYT | Glu261, Gly285, Thr286, Gly287, Ser289, His290, Lys320, Lys322, Tyr324, Thr440, Arg442 | |||
| Nsp13 NCB site | 6JYT | Glu143, Arg178, Asn179, Val181, Thr228, His230, Cys309, Ser310, His311, Arg339, Asn361, Pro408, Arg409, Thr410, | |||
| N protein NCB site | 6YI3 | Arg41, Pro42, Leu45, Asn48, Thr49, Ala50, Ser51, Ala90, Thr91, Tyr109, Pro117, Pro151, | |||
| Luteolin | Host | IL-6 | 1ALU | Ser176, Arg182, Leu178, Arg179 | [126] |
| STAT1 | 2KA6 | Asp24 | [102] | ||
| IL-2 | 5LQB | Lys52, Thr57 | |||
| TNF | 5M2J | Asp45 | |||
| Kaempferol | Host | NF-κB | 1IKN | Gly31, Alh192, Asp185 | [102] |
| IκB-α | 1NFI | Gln212, Gly206, Arg245 | |||
| IL-6 | 1ALU | Arg179, Arg182, Leu178, Arg30 | [126] | ||
| SARS-CoV-2 | Mpro | 6LU7 | Try54, Glu166, Met165, Met49, Cys145, His41 |
*n.a as none available in cited References.
*Epro.pdb provided by COVID-19 Docking Server (https://ncov.schanglab.org.cn/).
*Protein amino acid residues interact by hydrogen bonds with ligands labeled in blue based on the indications of cited References.
4.2. In silico of quercetin derivatives on targets of SARS-CoV-2
A molecular docking study on the interaction with the active site of Mpro to screen anti-COVID-19 potential of the phytocompounds from the Acacia pennata had results that showed several flavonoids with a quercetin-similar chemical backbone as C6–C3–C6 structure act on the active site of Mpro [83]. Based on evidence from in silico simulations, many natural putative derivatives of quercetin and kaempferol both act on RdRp and Mpro, promising rutinoside flavonoids affecting SARS-CoV-2 replication [84]. The interaction between Quercetin 3-O-neohesperidoside and Mpro binding pockets is from the forming hydrogen bonds at Gly143, Cys145, Gln189, Thr190, and His41; and forming π-π interaction at His41 residues. The interaction between Quercetin 3-Rhamnoside and Mpro by forming hydrogen bonds at same amino acid residues as Quercetin 3-O-neohesperidoside [85]. The molecular docking simulation showed quercetin and its derivatives interacts with SARS-CoV-2 Mpro active sites but binds on the regulatory site, dimerization site, or other positions to indicate quercetin and its derivatives may inhibit or affect Mpro activity as the competitive or non-competitive inhibitor [67,86], but this needs additional experiments to verify it.
The results provide a high binding affinity between S-protein/quercetin 3-(rhamnosyl-(1 → 2)-α-l-arabinopyranoside], PLpro/Quercetin 3-O-arabinoside 7-O-rhamnoside, and 3CLpro/Quercetin-3-neohesperidoside-7-rhamnoside [87]. Quercetin 3-O-arabinoside 7-O-rhamnoside forms 9 hydrogen bonds with PLpro via 9 amino acid residues at Lys27, Gln41, Arg42, Arg72, Arg74, Asn157, Lys158, Glu162, and His176. Quercetin-3-neohesperidoside-7-rhamnoside forms 10 hydrogen bonds with 3CLpro via 7 amino acid residues Asn133, Thr169, Ala194, Asp197, Thr199, Asn238. and Leu287. Quercetin 3-[rhamnosyl-(1 → 2)-α-l-arabinopyranoside] forms 7 hydrogen bonds with S-protein via 5 amino acid residues Ala348, Tyr385, Asn394, Glu398, and Arg514 [87]. Quercetin-3-Orutinoside and quercetin-7-O-glucoside-3-O-rutinoside are metabolic products of quercetin glycoside that have the highest binding affinity with the Mpro of SARS-CoV-2 [84]. The chemical structure of myricetin has one more hydroxy group than quercetin that forms the interaction with Mpro at same amino acid resides at Leu141, Gly143, Ser144, Cys145, His163, and Met165 as quercetin [88]. Quercetin-3-glucoside is a monoglycosylated quercetin derivative with higher water solubility than quercetin, also called isoquercetin [89]. Isoquercerin forms double hydrogen bonds with two amino acid residues at Csy145 and Asn142 in the active site of Mpro to provide strong inhibition [90]. Another in silico study showed isoquercetin interacts with multiple viral proteins of SARS-CoV-2 to form hydrogen bonds with Mpro at Glu166, Asn146, and His41 residues, forms hydrogen bonds with S-protein at Phe347, Val350, Asp442, and Phe497 residues, and forms hydrogen bonds with RdRp at Trp617, Asp618, Tyr619, Asp760, and Lys798 residues [86]. Quercetin 3-O-robinobioside kaempferol, and quercetin are phytochemicals that could be isolated from Boerhavia diffusa with similar quercetin chemical backbones that may show the inhibiting effect on the Mpro by molecular docking simulation [91].
Quercetin acts on viral proteins to affect COVID-19 infection and in silico results have revealed that several quercetin derivatives act on the viral proteins of SARS-CoV-2 [92]. Quercetin can biosynthesis from kaempferol or de-glycosylation from rutin which has the same chemical backbone structure with only one different R-group (Fig. 2). The natural polyphenols luteolin and myricetin have a similar chemical backbone to quercetin, in silico docking simulation showed that the two compounds similarly interacted with S-protein RBD of SARS-CoV-2 at the amino acid residues Arg454, Arg457, Lys458, Asp467, and Glu471 [88] (Table 1).
Recently, the Omicron variant of SARS-CoV-2 quickly worldwide, molecular docking calculation showed quercetin 3-O-β-d-glucuronopyranoside and quercetin-3-O-glucuronide 6″-O-methyl ester may have a strong inhibition on the RBD of Omicron variant [93]. Moreover, the binding affinity of quercetin and its metabolic derivatives toward furin enzymes or S-protein of SARS-CoV-2 may be affected by the micro-environmental pH value. Increasing the pH value may cause deprotonation on quercetin to decrease the number of hydrogen bond formations and increase the length of hydrogen bounds to drop its inhibitory activity on viral proteins [94].
4.3. In silico of quercetin and its derivatives on targets of host cells
Quercetin forms binding interaction with viral non-structural proteins of SARS-CoV-2 as well as has a high binding affinity with COVID-19 reacted proteins of host, such as ACE2, ABL1, and TMPRSS2 [92,95]. ACE2 and NRP1 as the host viral receptors for the S-protein of SARS-CoV-2 binding triggers the viral infection and enter host cells, so one promising strategy to prevent SARS-CoV-2 infection is interrupted or blocked the interaction between S-protein and ACE2/NRP1 [92]. The first molecular docking study about quercetin acting on ACE2 and S-protein of SARS-CoV-2 was reported [96] and it provided evidence for quercetin having a high binding affinity with both targets: host ACE2 and viral S-protein by forming hydrogen bonds with ACE2 at Arg273, Asp269, Asn149, and Tyr127 residues. Further that quercetin forms hydrogen bonds within the binding pocket of RBD of S-protein at Lys462, Glu465, Arg466, Asp146, and Ile123 residues [96]. In silico evidences that quercetin affords a high binding affinity with S-protein by forming hydrogen bonds or π-π interactions with four amino acid residues Asn501, Tyr505, Gly496, and Tyr453 within the ACE2 binding packet of RBD [67], and several quercetin derivatives can simultaneously act on all three proteins of ACE2, NRP1, and S-protein to prevent protein-protein interactions between S-protein and ACE2/NRP1 receptors [92]. Interestingly, MLN-4760 is an ACE2 inhibitor that acts on the extracellular metallopeptidase domain of ACE2, the molecular docking results showed (rutin and quercetin) interacted with amino acid residues of ACE2 are similar to MLN-4760 (the natural inhibitor of ACE2) while have a higher binding affinity than MLN-4760 [97]. Quercetin acts on ACE2 by forming hydrogen bond interactions at Asp350, Tyr385, Phe390, and Arg393 residues with the binding affinity as −7.86 kcal/mol [77]. In addition to ACE2, the host TMPRSS2 also served an important function on the initial stage of SARS-Co-V-2 infection [3]. The coronavirus infects by first binding to ACE2 (a serine protease acting as the receptor), while another serine protease is necessary for priming the viral S-protein required for entering the cells. The TMPRSS2 of human cells play a significant role in proteolytic cleavage of SARS-Cov-2 S-protein and subsequent priming to the receptor ACE2. The catalytic domain with serine protease function is located at C-terminus of TMPRSS2, and it cleaves viral S-protein to facilitate the membrane fusion between SARS-CoV-2 and the host cells [98]. Based on the results of molecular docking calculation, the first report showed the inhibiting effect of quercetin on the TMPRSS2 because quercetin forms strong hydrogen bonds with TMPRSS2 at Gly383, Gly385, Asn398, Asn433, and Asp435 residues; weak carbon-hydrogens interaction at Gly259 and Asn398 residues; and π-alkyl bond at Ala400 [99]. Another molecular docking study indicated quercetin forms strong hydrogen bond interactions with the core functional amino acid residues of TMPRSS2 at Lys390, Gln438, Ser436, and Cys465 residues, and forms the π-π interactions at Cys437 and Trp461 that near the catalytic site of TMPRSS2 [100].
4.4. In silico of quercetin and its derivatives on inflammation and its targets of host cells
Host cells infected by SARS-CoV-2 may cause oxidative stresses, cell injury, cytokine storm, serious inflammations, and organ functional damages are the major etiological factors of COVID-19 pathogenesis. Quercetin forms interactions with different viral proteins of SARS-CoV-2 to affect the virus replication and acts on several host-based proteins to attenuate infected symptoms of COVID-19 pandemic. SARS-CoV-2 infection caused the activation of NF-κB signaling pathway, which leads to upregulating several inflammatory factors synthesis and release [101]. ORF8 of SARS-CoV-2 is a viral protein with 121 amino acids that forms the ORF8 dimer or interact with the host protein IRF3 or MHC-I to form ORF8-IRF3 protein complex or ORF8-MHC-1 complex [102,103]. The ORF8 dimer, ORF8-IRF3 complex and ORF8-MHC-1 complex may hijack the induction of host immune system, ORF8-IRF3 complex may inhibit NF-κB signal pathway to decrease IFN production and attenuate the downstream immune response [102]. Rutin and Quercetin 3-O-(6′-galloyl)-β-d-galactopyranoside can dock on the interface residues between OFR8 and IRF3 to disturb the formation of ORF8-IRF3 complex, and that may help virus scavenging by host immune responses [102]. It postulates that the promotion of host immunity against viral invasions.
Quercetin, kaempferol, and luteolin are the major bioactive components identified from Yindan Jiedu granules (YDJDG), which have an inhibiting effect on NF-κB signaling pathway [75]. The results found quercetin binds with NF-κB by hydrogen bonds at four residues: Gly31, Arg33, Thr191, and Ala192; and with IκB-α by hydrogen bonds at Lys177, Arg245, and Asp208 residues. The luteolin binds with NF-κB by hydrogen bonds at Gly31, Asp185, and Lys218 residues, and with IκB-α hydrogen bond at Gln 212 residues. The kaempferol binds with NF-κB by hydrogen bonds at three residues: Gly31, Alh192, and Asp185; and with IκB-α by hydrogen bonds at Gln212, Gly206, and Arg245 residues [75].
Quercetin inhibits the protein expressions of NLRP3 inflammasome pathway to decrease pro-inflammatory cytokine expressions as curcumin does [78], and the docking results confirmed quercetin forms hydrogen bonds within the ATP binding sites of p38/MAPK at Lys53, Thr106, His107, Met109, Asp112, and Asp168 residues; and binding with the ATP binding pocket of JNK2 at Glu109, Met111. and Gln117 residues [104]. The activation and expression of intracellular STAT3, PI3K, and MAPK are key targets for anti-inflammation. Molecular docking showed quercetin and luteolin interacts with STAT3, PIK3R1, and MAPK1 [105].
4.5. Immune response of quercetin and its derivatives on targets of host cells via in silico
The hyper-activation of the immune system causes an acute severe systemic inflammatory response called cytokine release syndrome (CRS). No effective prophylactic or post-exposure treatments are available, although some anti-inflammatory compounds are currently in clinical trials. The cytokine storm is one of the main causes of mortality by severe SARS-CoV-2 infection. The increase expressions of IL-1β, IL-6 and TNF-α levels were found in the pro-inflammatory status of SARS-CoV-2 infection, and quercetin interacts with those three pro-inflammatory cytokines to attenuate the downstream inflammatory pathways. The molecular docking calculation showed the strong interaction between quercetin and IL-1β by formed 6 hydrogen bonds with 5 amino acid residues at Asn92, Glu149, Lys150, Tyr153, and Tyr175. The quercetin interacts with TNF-α by two hydrogen bonds at Leu113 and Gln201. Quercetin forms a stable interaction with IL-6 by hydrogen bonds at the amino acid residues Glu127, Gln130, Glu137, and Arg141 [106].
One study reported that patients infected by SARS-CoV-2 may increase CCL2, CXCL8, FOS, IFN-β, IL-1A, IL-1B, and SERPINE1 gene expressions, suggesting that it participates in cytokines, inflammation, and oxidative stress pathways. Molecular docking results shows that quercetin acts on the proteins CCL2, CXCL8, FOS, IL-1α, IL-1β, and SERPINE1; rutin acts on CXCL8 and IL-1β; apigenin acts on FOS and SERPINE1; and baicalein acts on FOS [107]. Quercetin acts on the anti-inflammatory heme oxygenase-1 (HO-1) pathway to inhibit the expressions of TNF-α, IL-1β, IL-6, and NO production in the serum to attenuate inflammation induced by infection [108,109]. In the HO-1 pathway, quercetin did not affect the expression of kelch-like ECH-associated protein-1(Keap1), but in silico result showed quercetin binds on the Nrf2 binding site of Keap1 and leads to the expressions of downstream anti-oxidative genes [110]. Additionally, several quercetin and its derivatives (quercetin, kaempferol, luteolin, myricetin, and apigenin) were isolated from Platycladus orientalis form hydrogen bonds within the active site of xanthine oxidase to inhibit the enzyme activity and reactive oxygen species (ROS) production [111]. A total of 214 active ingredients and 339 target genes of Shufeng Jiedu capsules (SFJDC) were collected. Of note (quercetin, kaempferol, luteolin) and 10 hub target genes (TP53, AKT1, ANXA1, CTNNB1, NCOA1, EGFR, PRKCA, NCOA2, RELA, and FOS) were identified based on network analysis. The hub target genes are mostly augmented in pathways including MAPK signaling pathway, PI3K-Akt signaling pathway, and cAMP signaling pathway, which could be the underlying pharmacological mechanisms of SFJDC for treating COVID-19. Moreover, the key compounds had a high binding activity with three typical target proteins including ACE2, 2OFZ, and 1SSK [112].
4.6. In vitro and In vivo validation
To verify the results of in silico simulation, some of the studies performed further in vitro and in vivo tests. The cytotoxicity of quercetin on Vero E6 cells with 50 % cytotoxicity concentration (CC50) value as 301.5 μM. The anti-COVID-19 activity with 50 % inhibitory concentration (IC50) value as 18.2 μM. The selectivity indexes (SI CC50/IC50) of quercetin are about 17 and it had multiple molecular docking interactions with several SARS-CoV-2 viral proteins that indicate quercetin as a potential pharmaceutical candidate for SARS-CoV-2 treatment [113]. The SARS-CoV-2 infection was initiated by the viral S-protein binding with host membrane ACE2 receptor, ligands bind on the ACE2 may affect or interrupt the COVID-19 virus infection. The in vitro studies that were performed by surface plasmon resonance (SPR) technology showed the equilibrium dissociation constant (Kd) of quercetin binding with ACE2 is 5.92 μM with the IC50 of quercetin on recombinant human ACE2 was 4.48 μM [114], and several quercetin related glycosides also possessed the potential to be inhibitors of ACE2 [115]. The nsp13 of SARS-CoV-2 is a helicase for viral replication, quercetin and several flavonoids had a high binding affinity at the 5’ RNA binding site, the inhibiting effect of 30 μM quercetin completes blocking of the ATPase activity of nsp13. Quercetin, myricetin, and kaempferol inhibited SARS-CoV-2 nps13 through an unwinding activity at nanomolar concentrations but rare effects on viral replication [79].
The genomic expressions of ORF-1 in SARS-CoV-2 are translated into polyproteins and cleaved into functional proteins (non-structural proteins, nsp1-nsp16) by two major viral proteinases, Mpro and PLpro [116]. The inhibitions on the Mpro activities may inhibit the viral replication and infection, and an in vitro result demonstrate quercetin acts on the 3CLpro as the inhibitor with IC50 value range from 6.79 to 23.4 μM in different reports, and EC50 is 4.88 μM [69,71]. In vitro cell culture results showed natural quercetin inhibited SARS-CoV-2 replication in Vero cells at a relatively high concentration with the IC50 as 192 μM, and the quercetin modified into seleno-quercetin derivative can significantly improve the inhibiting effect on SARS-CoV-2 replication, and the best IC50 is 8 μM [118]. This shows that using quercetin as the structural backbone to modify and develop new bioactive compounds may provide more powerful pharmaceutical candidates for anti-SARS-CoV-2 treatments. Quercetin, and kaempferol are the major flavonoids of Hippophae rhamnoides. The result of an SPR assay showed the binding affinity of quercetin to human ACE2 protein with 5.92 μM of Kd, and the binding affinity of isorhamnetin was higher than quercetin with 2.51 μM of Kd. By using the SARS-CoV-2 spike pseudotyped virus assay, treated with 50 μM isorhamnetin inhibits 47.7 % viral entrance but treated by the same dose of quercetin had no effect [114].
Rutin is the quercetin with disaccharide retinose, also called quercetin-3-O-rutinose. Rutin is more water soluble and has more bioavailability than quercetin, which forms the interactions with Mpro at similar binding residues. In vitro Mpro activity shows that form an inhibiting test that is estimated to show that IC50 of rutin at about 32 μM [118]; and mixed rutin with l-arginine improves with more water solubility and its inhibiting effect on Mpro to decrease the Ki and IC50 values [119]. Another in vitro study used HCoV-229E to simulate SARS-CoV-2, the results showed the inhibitory effects of quercetin, isoquercetin, and rutin on Mpro activity of SARS-CoV-2 with 6.79 μM, 4.03 μM and 0.125 μM of IC50, respectively. The substitute test from the evaluation of the inhibiting effect on HCoV-229E replication in Huh-7 cells conformed with the antiviral effects of quercetin, isoquercetin, and rutin [71]. Another in vitro study also validated the ligands-protein interactions of SARS-CoV-2 by using fluorescence quenching methods and showed that the IC50 of quercetin on RdRp, Mpro and S-protein about 82 nM, 62 nM and 52 nM, respectively, as well as catechin had similar anti-COVID-19 potential. Its inhibiting efficacy on RdRp, Mpro and S-protein with 71 nM, 93 nM and 65 nM of IC50, respectively [120]. The nsp15 is uridylate specific endoribonuclease of SARS-CoV-2 that cleaved the viral own negative-sense RNA to evade the innate immune response [121]. In vitro results showed epigallocatechin gallate (EGCG) and baicalin inhibits nsp15 with 1.67 μM and 3.56 μM of IC50, respectively [122]. Further, another in vitro study tested the anti-COVID-19 effects of different combinations that mixed quercetin with different natural compounds to indicate the combination by resveratrol, broccoli extract, curcumin, quercetin, naringenin, baicalin, theaflavin, vitamin C, and N-acetylcysteine had the highest anti-SARS-CoV-2 potential. In vitro treatments with this combination (10 μg/mL) inhibited 90 % S-protein binding to ACE2, and 53 % RdRp activity to inhibit SARS-CoV-2 infection and replication [123]. Another in vitro study showed the inhibitory effect (IC50) of quercetin about 23.8 μM on Mpro and 8.7 μM on PLpro of SARS-CoV-2, respectively [124]. Additionally, the in vitro validation showed quercetin had a dose-dependent inhibiting effect on Mpro, used the non-linear regression to establish inhibition constant (Ki app) of quercetin on Mpro catalytic activity is 21 μM, and intrinsic inhibition constant (Ki) is 9.6 μM [125]. Direct binding evidence by an SPR assay showed that the equilibrium dissociation constants (Kd) value of quercetin on ACE2 was 0.67 mM; quercetin forms hydrogen bonds within the binding pocket of RBD of S-protein at Lys462, Glu465, Arg466, Asn146, and Ile123 residues with 2.21 μM of Kd [96] (Table 2).
Table 2.
The anti-SARS-CoV-2 targets and effects of Quercetin and its derivatives.
| Target | Quercetin/Quercetin derivatives | IC50 (μM) | CC50 (μM) | Method | Reference | |
|---|---|---|---|---|---|---|
| SARS-CoV-2 | Mpro | Quercetin | 6.79 | Measured by SARS-CoV-2 Assay Kit (BPS bioscience) | [71] | |
| Kaempferol | 6.83 | |||||
| Isoquercitrin | 4.03 | |||||
| Rutin | 0.125 | |||||
| Mpro | Quercetin | 23.4 | Measured by FRET | [69] | ||
| Mpro | Quercetin | 21 | Measured by FRET | [117] | ||
| Mpro | Rutin | 32 | Measured by FRET | [118] | ||
| Mpro | Quercetin | 62 nM | Measured by spectrofluorimetric assay | [120] | ||
| RdRp | Quercetin | 82 nM | ||||
| nsp13 | Quercetin | 10.2 | >100 | Measured by nsp13 unwinding associated activity | [79] | |
| nsp15 | Quercetin | 13.79 | Measured endoribonuclease activity by carboxyfluorescein fluorophore | [122] | ||
| S-protein | Quercetin | 52 nM | Measured by spectrofluorimetric assay | [120] | ||
| HOST | rh-ACE2 | Quercetin (2.5 min) | 4.48 | Measured rhACE2 activity by fluorogenic substrate Mca-APK(Dnp) | [115] | |
| Quercetin (10.5 min) | 29.5 | |||||
| ACE2 | Quercetin (KD) | 5.92 | Measured by SPR assay | [114] | ||
| Vero E6 cells | SARS-CoV-2 replication | Quercetin | 18.2 | 301 | Measured by MTT assay | [113] |
FRET: fluorescence resonance energy transfer; SPR: surface plasmon resonance; MTT: 3-[4,5-dimethylthiazol-2-yl]-2,5 diphenyl tetrazolium bromide.
There are several marketed herbal products developed in China or other countries that claimed antiviral activities with some suggested as having potential against COVID-19, but only few have been validated. In vitro results showed that when pretreated with herbal extracts of Jingyin granules (HEJG) there was an inhibiting effect on different drug-metabolizing enzymes (such as cytochrome P450 enzymes-CYPs) with the dose-dependent manners to affect pharmacokinetics of clinical medicines, which further indicated that cotreatment with HEJG and anti-viral drugs may increase the effective dose and prolong effective time for clinical drugs (such as lopinavir). Within HEJG, kaempferol and quercetin are major bioactive constituents of HEJG with inhibiting effects on the CYP3A [126]. Lopinavir is a general clinical medicine used for COVID-19 treatment. Rats pretreated with HEJG (3 g/kg) showed an inhibition of the activities of CPYs to influence the pharmacokinetic parameters of lopinavir to increase the maximum concentration in serum, prolong the half-life of antiviral drugs about 1.91 times, and extend the retention time [127]. Isoquercetin has higher water soluble, and the pharmacokinetic results showed oral administration with isoquercetin had over a 4-fold bioavailability when compared with quercetin in vivo [89]. Taken a deep insight into looking above sections of findings from in silico, preclinical tests and clinical trial, quercetin and its derivatives docked with various domain or segment proteins of SRAS-CoV-2 exert the suppression of inflammation and cytokine storm by coronavirus infected to combat COVID pandemic (Fig. 3).
5. Pharmaceutical potentials of quercetin and its derivatives in clinical trial of COVID-19 pandemic
Based on the ClinicalTrials. gov website (https://clinicaltrials.gov/), in 15 clinical trial enrollments, quercetin supplementation was used as a COVID-19 treatment. We also found other reports of six studies in PubMed (https://pubmed.ncbi.nlm.nih.gov/). In all clinical trials, quercetin was used as a supplement combined with standard care (SC) for symptomatic and antiviral treatment of COVID-19 patients (Table 3, Table 4). Outpatients with mild SARS-CoV-2 infections were treated with quercetin for two weeks (600 and 400 mg/daily of quercetin in the first and second weeks, respectively) in combination with SC, which significantly shortened the period of viral clearance, alleviated symptom occurrence, and attenuated the levels of lactate dehydrogenase (LDH) and ferritin in serum [128]. In the early stages of COVID-19, quercetin supplementation resulted in marked improvements in the ratio of hospitalized patients, decreased the oxygen needs of patients, and shortened the days of hospitalization [129]. Patients with severe SARS-CoV-2 infection were treated with 1000 mg/day of quercetin in combination with clinical antiviral drugs (such as remdesivir and favipiravir), which significantly decreased the levels of q-C-reactive protein (q-CRP), LDH, and alkaline phosphatase (ALP) in the serum and reduced the period of hospitalization [130].
Table 3.
Clinical trial of quercetin on COVID-19 treatment from PubMed and ClinicalTrial.gov.
| Formulation/Design | Phase | Regimen (Oral) | Patients (n) | Masking | Age (y) | Placebo (n) | Country | Authors or Institute | Serial number/(Other ID or DOI) |
|---|---|---|---|---|---|---|---|---|---|
| Quercetin Phytosome | 3 | 400 mg/daily | 152/200 | none | >18 | – | Pakistan | Ikram Din Ujjan | NCT04578158/(LUMHS/REC/894) |
| Quercetin Prophylaxis | – | 500 mg/daily | 447 | none | >18 | – | Turkey | Hasan Onal | NCT04377789/(KSSEAH--0058) |
| Quercetin Treatment | 1000 mg/daily | ||||||||
| Quercetin Phytosome | – | 600 mg/daily 1st week, 400 mg/daily 2ed week | 100/142 | none | >18 | – | Pakistan | King Edward Medical University | NCT04861298/(192/RC/KEMU) |
| Quercetin Treatment | 4 | 500 mg/daily | 60 | none | >18 | – | Saudi Arabia | Hiba Hamadelnil elsaeed | NCT04468139/(20–95 M) |
| Zinc Treatment | 50 mg/daily | ||||||||
| Bromelain Treatment | 500 mg/daily | ||||||||
| Vitamin C Treatment | 1000 mg/daily | ||||||||
| Quercetin/curcumin combination treatment | – | – | 50 | none | >18 | – | Pakistan | King Edward Medical University | NCT05130671/(785/RC/KEMU) |
| Quercetin Treatment | – | 500 mg, twice daily | 80 | double | >18 | 40 | Italy | Mariangela Rondanelli | NCT05037240/(1222/01022021) |
| Curcumin, Quercetin and Vitamin D3 combination treatment | – | curcumin168 mg, quercetin 260 mg, vitamin D3 360 IU | 50 | none | >18 | – | Pakistan | Liaquat University Hospital | NCT04603690/(LUMHS/REC/173) |
| Quercetix | 1 | one tablet twice daily (Acetyl-l-carnitine 500 mg, quercetin 200 mg, vitamin B 12 33 mg, Vitamin E 10 mg) | 80 | double | >18 | 40 | Tunisia | Hôpital Universitaire Sahloul | NCT04851821/(Quercetix) |
| Isoquercetin | 2 | 1000 mg/daily | 200 | triple | >18 | 100 | France | Pascal Chanez | NCT04622865/(AB20001)/(2020-001635-27) |
| Masitinib, | 3 mg/kg/day for 4 day, follow 4.5 mg/kg/day | ||||||||
| QUERCOV | 1 | one tablet twice daily | 200 | triple | 13–59 | 100 | Tunisia | Riadh Boukef | NCT04853199/(QUERCOV) |
| Extract Psidii guava | 3 | 2 Capsule Extract Psidii guava, three times daily | 90 | double | >18 | 45 | Indonesia | Fredia Heppy | NCT04810728/(PSIDII0520_COV19) |
| Isoquercetin | 2 | Isoquercetin 1000 mg on day 1, then 500 mg | 150 | single | >18 | 75 | USA | Institut de Recherches Cliniques de Montreal | NCT04536090/(IRCM-IQC-001) |
| NASAFYTOL | – | 1008 mg, 4 capsules twice a days | 51 | none | >18 | 25 | Belgium | Tilman S.A. | NCT04844658/(CHOPIN) |
| Quercetin | – | 1000 mg/daily | 60/72 | none | 32–79 | 30 | Iran | Shohan M | IRCT20200419047128N2 [130], |
| Yindan Jiedu granules | – | 12 or 24 g, 3 times daily | 262/270 | none | 18–86 | – | China | Fang Y | China, No. Z20200012000 |
| Quercetin Phytosome® (lecithin-based delivery form, quercetin 200 mg in 500 mg tablet) | – | 3 tablets/daily for 1st week, 2 tablets/daily for 2ed week | 42/50 | none | >18 | 21 | Pakistan | Di Pierro F | 192/RC/KEMU [128] |
| 3 | 2 tablets/daily | 152 | none | >18 | 76 | Pakistan | Di Pierro F | NCT04578158 [129] | |
| Shufeng Jiedu | – | 2.08 g, 3 times daily | 76 | none | >18 | 33 | China | Xia L | YJ-92 2020-S015–02 [132] |
| multi-component OTC | – | 25 mg zinc; 10 drops of Quina™; 400 mg quercetin; 1000 mg vitamin C; 1000 IU (25 mg) vitamin D3; 400 IU Vitamin E; and 500 mg l-lysine | 113 | none | 30–59 | 60 | USA | Margolin L | [133] |
“-“ as no mention.
Table 4.
Clinical trial results of quercetin on COVID-19 treatment from PubMed and ClinicalTrial.gov.
| Formulation (daily, Oral) | Patient (n) | Age (y) | Country | Authors | Results (intervened 7th day) | Serial number |
|---|---|---|---|---|---|---|
| Quercetin 200 mg/tab, 2 tab/daily | 152/200 | 18∼80 | Pakistan | Di Pierro et al. | Decrease hospitalization days, non-invasive oxygen therapy, ICU, and death | NCT04578158 [128] |
| Quercetin 200 mg/tab, 2 tab/daily | 100/108 | 47.6 ± 15.7 | Pakistan | Di Pierro et al. | Decrease RT-PCR viral positive; Speedy clinical recovery; Decrease LDH level |
192/RC/KEMU; NCT04861298 [136] |
| Quercetin 200 mg/tab, 3 tab/daily | 42 | 49.3 ± 16.5 | Pakistan | Di Pierro et al. | Decrease RT-PCR viral positive; Decrease LDH, Ferritin, CRP, and D-dimer levels |
192/RC/KEMU; NCT04861298 [129] |
| Quercetin 500 mg/tab, 2 tab/daily | 60 | 35∼75 | Iran | Shohan et al. | Decrease RT-PCR viral positive and post-intervention discharge; Decrease the symptoms of fever, weakness and lethargy; Decrease ALP, q-CRP, and LDH levels |
IRCT20200419047128N2 [130] |
| Curcumin (168 mg) Quercetin (260 mg) Vitamin D3 (9 μg) |
50 | 46–67 | Belgium | Gérain et al. | Decrease hospitalization, ICU, and COVID-19 WHO ordinal outcome score; Increase discharged participants |
B4062020000305 [137] |
| Curcumin (168 mg) Quercetin (260 mg), Vitamin D3 (9 μg) |
56/66 | 32∼52 | Pakistan | Khan et al. | Decrease RT-PCR viral positive, symptom of cough; Decrease CRP level |
785/RC/KEMU; NCT05130671 [138] |
| Curcumin (168 mg) Quercetin (260 mg) Vitamin D3 (9 μg) |
50/64 | 30∼50 | Pakistan | Ujjan et al. | Decrease RT-PCR viral positive, symptoms of myalgia, asthenia and dysgeusia; Decrease hs-CRP, D-dimer, LDH, Ferritin levels |
LUMHS/REC/137; NCT04603690 [139] |
The anti-COVID-19 efficacy of several traditional Chinese or herbal medicine patent prescriptions (TCMPPs or THMPPs) was determined within three years (2020–2022); however, they were applied or passed a clinical trial in only a few cases. Quercetin is the major bioactive component of TCMPPs and THMPPs. Yindan Jiedu granules (YDJDG) are TCMPPs originating from China, and clinical trials have shown that treatment with YDJGG (12 or 24 g, three times per day) suppressed the progression of COVID-19 based on the 1:1-ratio propensity score matching (PSM). Notably, quercetin is an effective component of YDJDG and modulates the NFκB pathway to attenuate inflammation [131]. Shufeng Jiedu capsules (SFJDC) are another type of THMPPs developed in China. In COVID-19 patients, antiviral therapy combined with SFJDC supplementation (2.08 g, three times daily) significantly alleviated coughing and fatigue symptoms, improved rehabilitation, and increased asymptomatic periods during the entire viral infection period compared with antiviral therapy alone [132].
In one clinical trial report, a multi-component over-the-counter (OTC) drug (comprising 10 drops of Quina™, 400 mg of quercetin, 25 mg of zinc, 1000 mg of vitamin C, 1000 IU (25 mg) of vitamin D3, 400 IU of vitamin E, and 500 mg of l-lysine) was used to treat early-stage COVID-19 patients. When supplied with OTC drugs, infected patients showed an asymptomatic status and a decreased ratio to become symptomatic [133]. Other studies on the effects and mechanisms of vitamin D3, quercetin, and estradiol on anti-inflammation, anti-oxidation, and antiviral infection indicated that their use in a tripartite combination is a potential mitigation agent of COVID-19 [134,135]. Quercetin possesses strong anti-inflammatory, anti-oxidant, immunomodulatory, and antiviral characteristics, which are considered to indicate a high safety profile, as determined by preclinical studies on animals and humans. Recently, quercetin was used as an adjuvant therapy in patients with COVID-19, and the results showed an improvement in clinical symptoms and a reduction in the length of hospitalization [128] (Di Pierro et al., 2021a). To date, only three different quercetin formulations have been investigated in clinical trials and published, with seven reports in PubMed, to evaluate the therapeutic and prophylactic potential of quercetin against SARS-CoV-2 infection (Table 4). Based on these reports, the administration of quercetin in SARS-CoV-2-infected patients can enhance recovery and decrease the acute and serious infective symptoms [[128], [129], [130],[136], [137], [138], [139]]. Most clinical reports have showed that in comparison with those in the control group, quercetin intervention could attenuate the levels of inflammatory biomarkers in patient serum on the 7th day after intervention [129,130,138,139].
6. To accelerate the prospective of in-silico findings
Currently, to rapidly track the urgent demand for treatments regardless of the COVID-19 pandemic or chronic diseases and syndromes, namely, diabetes, metabolic syndrome, and hypertension, a new bioinformatics approach has garnered research interest to determine the therapeutic effect in drug discovery and development, and the underlying mechanism of small molecules in signaling pathways. In several studies, network pharmacology was combined with molecular docking to investigate the potential compounds of traditional Chinese medicine (TCM) formulas for SARS-CoV-2 therapies. Many in-silico studies have shown that quercetin acts on the target proteins of SARS-CoV-2 and the concomitant pathway of COVID-19 pathogenesis [135,140,141]. Quercetin, luteolin, and kaempferol not only bind and inhibit Mpro, but can also dock on nine therapeutic targets, namely, IL-6, tumor necrosis factor (TNF), microtubule associated protein kinase 1 (MAPK1), CASP3, CXCL8, IL-10, IL-1β, MAPK8, and VEGFA [126]. Quercetin, luteolin, and kaempferol are the major bioactive flavonoids in Lianhuaqingwen capsule (LHQW-C), indicating that the above mixture is a TCM formula used for COVID-19 treatment. Kyoto encyclopedia of genes and genomes (KEGG) enrichment analysis indicated that the targets of LHQW-C highly enhanced several immune response-related and inflammation-related pathways, including the TNF signaling pathway, NF-κB signaling pathway, IL-17 signaling pathway, and Th17 cell differentiation. Moreover, kaempferol, quercetin, and luteolin showed high binding affinities for 3CLpro of SARS-CoV-2. One study revealed that some anti-inflammatory constituents of LHQW-C moderate the inflammatory response in severely ill patients with COVID-19 [126].
Additionally, an online COVID-19 docking server (http://ncov.schanglab.org.cn) was developed to apply small molecular ligands interacting with relative proteins of SARS-CoV-2 [142]. This docking server was used to screen the bioactive components from Mexican herbal medicines, and the simulation results showed that quercetin acts on several viral nsps and is one of the top three natural compounds with potential against SARS-CoV-2 [143]. Second, quercetin-3-O-sophoroside has a high binding affinity for several SARS-CoV-2 proteins, including E-protein, N-protein, nsp14, nsp15, nsp16, PLpro, Mpro, and RdRp [144].
Notably, numerous studies have investigated the docking of Mpro with quercetin, which has different amino acid residues at each binding site. Notably, SAR can be used to explain and identify potentially important residues. All the above studies showed that quercetin develops other interactions with Mpro in addition to the protease active sites, and may act as a mechanism of the allosteric inhibition of Mpro [145]. Certain amino acids in Mpro play a major role in binding, as determined by many studies, whereas other studies found that allosteric regulation is likely to exist. Additionally, the in-vitro validation assay was confirmed using amino acid mutations. Moreover, illustrating the direct binding or interaction of quercetin with target molecules requires further studies with target identification methods, such as surface plasmon resonance (SPR), isothermal titration calorimetry (ITC), microscale thermophoresis (MST), drug affinity responsive target stability (DARTS), stability of proteins from rates of oxidation (SPROX), and cellular thermal shift assay (CETSA), which are applicable to natural products, as well as indirect evidence through biological and pharmacological evaluations (in vitro and in vivo) [146]. Quercetin, rutin, and isoquercetin are the major bioactive natural compounds found in Toujie Quwen Granules, and have high binding scores for IL-6, ACE2, and S-protein. Further evidence based on SPR indicates that quercetin and isoquercetin bind to the RBD of the S-protein to interrupt the attachment and binding of the S-protein to the host ACE2, whereas rutin binds to ACE2 to decrease and dwindle the SARS-CoV-2 infection [147]. The S-protein of coronavirus activates the ERK-MAPK pathway to affect ACE2 expression, thereby increasing viral infection [148]. Once SARS-CoV-2 binds to ACE2, it causes viral replication, oxidative stress, and an immune response, which subsequently mediates the p38/MAPK signaling pathway and induces the upregulation of AP-1 through ERK-pJNK to overexpress ACE2 to increase the binding of coronavirus. Moreover, the production of reactive oxygen species (ROS), inflammation, and cytokine storms resulted in the activation of JAK/stat1, inflammatory cytokines (IL, IFN, and TNF), NF-κB, and NLRP3-translocated regulation of pro-inflammatory and IFN-stimulated genes.
7. The possible mechanisms of quercetin when targeting SARS-CoV-2 infection
Quercetin and its derivatives act on multiple pathways, including extracellular and cytoplasmic pathways, to abrogate SARS-CoV-2 infection (Fig. 4). Based on the above literature, the major anti-COVID-19 mechanisms of quercetin and its derivatives may involve three main routes for modulating and inhibiting SARS-CoV-2 infection. First, quercetin and its derivatives can interrupt the viral-host protein interaction by interrupting and preventing viral S-protein anchoring on the host ACE2/TMPRSS2, which may block membrane fusion between the virus and host cell and prevent viral entry into the host cell. Second, quercetin and its derivatives are predicted to have multiple binding characteristics to interact with several SARS-CoV-2 proteins, especially by binding to the active sides of viral proteins, which can inhibit viral replication and attenuate host intracellular oxidative stress by viral infection. Third, quercetin and its derivatives act on several host signaling pathways to attenuate oxidative stress, inhibit the synthesis of inflammatory cytokines, and activate autophagy. Quercetin and some of its derivatives can induce autophagy inducers [149,150]. Treatment with quercetin or its derivatives can activate the AMP-activated protein kinase (AMPK) pathway to promote autophagy in infected cells, which can help host cells remove viral proteins, harmful proteins, or impaired organelles. In other studies, autophagy was shown to act on the P38/MAPK pathway to downregulate the PI3K/AKT/mTOR and NLRP3 inflammasome pathways and decrease cytokine synthesis, which may attenuate the risk of developing a cytokine storm after SARS-CoV-2 infection.
Fig. 4.

The mediation of quercetin and its derivatives on (a) the inflammation and cytokine storm, (b). The expressions of inflammatory and interferon-stimulated genes and (c) the oxidative stress induced by SARS-CoV-2 infection.
8. Quercetin and its derivative as an adjuvant synergistic with other drugs for COVID-19 treatment
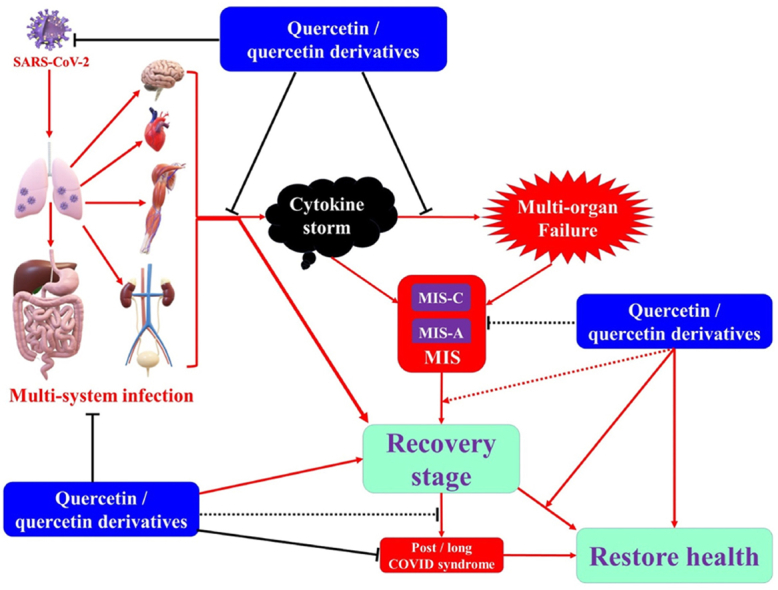
Additionally, there is a prospect for the development of formulations using different permutations and combinations of these phytomolecules to harness their synergistic potential. In another in-silico study, the anti-COVID-19 potential of several clinical anti-human immunodeficiency virus (HIV) drugs and phytoflavonoids was screened. The results showed that synergistic treatment with phyto-flavonoids and anti-HIV drugs could increase the docking score of anti-HIV drugs for SARS-CoV-2 Mpro. This study also indicated that synergistic treatment with quercetin-3-rhamnoside and darunavir had the highest docking score for SARS-CoV-2 Mpro, suggesting that this combination could be used as an effective approach against SARS-CoV-2 [151]. As expected, the high incidence of post-COVID-19 symptoms was ascribed to the long-term complications of COVID-19; this simultaneously provided a complex view that emphasized multidisciplinary care and the prophylactic and therapeutic potential of such treatments. The most advantageous flavonoid, quercetin, showed significant therapeutic and preventive effects for the mitigation and shortening of the period concomitant with post-COVID-19 syndrome [151,152]. Increasing evidence has revealed that many patients develop a chronic condition characterized by fatigue, neuropsychiatric symptoms, various neurological disorders, such as headache or myalgia, and more severe symptoms, such as stroke, psychosis (brain fog), and anosmia, termed long-COVID. There is an urgent need to identify possible interventions to mitigate the crossing of the blood-brain barrier (BBB) by the S-protein, which results in perivascular inflammation. Notably, the use of small natural molecules, especially luteolin and quercetin, to cross the BBB abrogates this detrimental effect [[153], [154], [155]].
Multisystem inflammatory syndrome (MIS) is a post-viral immunological or hyperinflammatory complication of SARS-CoV-2 infection in children (MIS-C) [156], adults (MIS-A) [157], or after vaccination (MIS-V). MIS-C is commonly observed in older children and is characterized by multi-organ dysfunction involving cardiac, renal, respiratory, hematologic, and acute gastrointestinal problems; neurological symptoms; rash or bilateral non-purulent conjunctivitis; hypotension; or shock. Its main manifestations include abdominal pain, diarrhea, fever, myocarditis, and coronary artery aneurysms [158]. The average age of children with MIS-C (56.8 % of male) was 9 years. Fever (100 %), gastrointestinal (GI) (82 %), and abdominal pain (68 %) were the decisive symptoms in the diagnosis of MIS-C. Shock and/or hypotension is common in patients with MIS-C. Cardiac symptoms (66 %) are dominant over respiratory (39 %) and neurological (28 %) symptoms [159]. However, pediatric COVID-19 is still a mild disease, affecting only 8 % of children. The pathogenesis of SARS-CoV-2 infection in children is comparable with that in adults, which indicates the impaired activation of IFN-α and IFN regulator 3 and decreased cell response, causing impaired viral defense; however, the clinical course is mild, and all children recover from the infection without major complications or sequelae. Furthermore, the clinical manifestations of MIS-C resemble certain pediatric rheumatologic diseases, such as Kawasaki disease (mucocutaneous lymph node syndrome), which distress the small-medium vessels [160]. Most patients with MIS-C have increased levels of at least four inflammatory markers (C-reactive protein, neutrophil count, ferritin, procalcitonin, fibrinogen, interleukin-6, and triglycerides) [161]. Critically, MIS-C, a hyper-inflammatory syndrome associated with SARS-CoV-2 infection, shares clinical features with toxic shock syndrome (TSS), which is triggered by bacterial superantigens (SAgs). Superantigen specificity for different Vβ chains results in Vβ skewing, wherein T cells with specific Vβ chains and varied antigen specificity are overrepresented in the T cell receptor (TCR) repertoire. Notably, in-silico modeling revealed that polyacidic residues in the Vβ chain encoded by TRBV11-2 (Vβ21.3) strongly interact with the SAg-like motif of the SARS-CoV-2 S-glycoprotein, suggesting that the unprocessed S-protein of SARS-CoV-2 may directly modulate TRBV11-2 expansion [162].
The pathology of COVID-19 is still characterized by a cytokine storm, such as an increased inflammatory response involving IL-6, TNF-α, and monocyte chemoattractant proteins that lead to endothelial inflammation, microvascular thrombosis, and multiple organ failure. An acute cytokine storm in severe COVID-19 results in multi-organ damage owing to vascular hyperpermeability, edema, and hypercoagulation. The consequences of SARS-CoV-2 infection include long-COVID (i.e., long-term) or post-COVID (i.e., short-term) syndromes and MIS-C [163,164]. In particular, COVID syndrome may be characterized by long-term tissue damage (e.g., lung, brain, and heart) and pathological inflammation (e.g., viral persistence, immune dysregulation, and autoimmunity) associated with increased levels of specific biomarkers (e.g., CRP, D-dimer, and lymphocyte count) [163]. Increasing evidence has indicated persistent and/or delayed complications from symptom onset in acute COVID-19. The pathophysiology and organ-specific sequelae of post-acute viral syndromes have been described in survivors of other infectious coronavirus epidemics [164]. The sequelae of coronavirus may be attributed to the manifestations of post viral syndrome, especially post- and long-COVID.
Based on the anti-inflammatory, immune-modulated, and cardiovascular protective effects of quercetin and its derivatives, the search of phytochemicals, namely, quercetin and its derivatives, that can bind to the S-protein of SARS-CoV-2 to block the interaction with TRBV11-2 (Vβ21.3) and reduce the symptoms or occurrence of MIS-C will be ongoing. Herbal compounds (mostly polyphenols and flavonoids, namely, luteolin) are known to possess a broad spectrum of pharmacological properties, such as anti-oxidant, anti-inflammatory, and antiviral activities, suggesting their role as a micronutrient in the prevention of the inflammatory cascade to alleviate manifestations of post-COVID, long-COVID, and MIS-C.
Unfortunately, according to the global statistics of population, the percentage of vaccination is over 63 % (1), whereas the low cumulative mortality is only approximately 1 %. Compared with the rapid decline of the SARS outbreak in the past decade, the declining tendency of COVID-19 pandemic is devastating, and COVID-19 may become infectious and flu-like in the future. In contrast, the high mutation rate of SARS-CoV-2 may give rise to new immune escape variants for vaccinated or infected people, which can increase the contagious risk. Notably, this multi-targeting potential of quercetin and its derivatives on several proteins of SARS-CoV-2 can potentially help combat COVID-19 and long-COVID.
9. Conclusion and future prospective
We provided a comprehensive review of the in-silico, in-vitro, in-vivo, and clinical literature examining the anti-SARS-CoV-2 effectiveness of quercetin and its derivatives. The evidence from in-silico simulations showed the potential multi-targeting effect of quercetin and its derivatives on several proteins of SARS-CoV-2 and host cells, some of which have been determined to combat COVID-19 through in-vitro, in-vivo, and clinical settings. From May 2023, the WHO and most countries announced the end of the emergency phase of the COVID-19 pandemic, and that most people have received several vaccinations; however, the variants of SARS-CoV-2 still spread worldwide and continue to infect several million people every year (https://covid19.who.int/). Considering the cost of global actions to fight the COVID-19 pandemic, the COVID-19 pandemic never ceased but became integrated into our everyday lives, thereby indicating the necessity and urgency of developing treatment strategies that are cheap and easy to obtain. Recent anti-SARS-CoV-2 studies have demonstrated the anti-inflammatory, anti-oxidative, neuroprotective, and cardiovascular protective effects of quercetin and its derivatives, suggesting their preventive and therapeutic potential against the ongoing COVID-19 pandemic and COVID-19-associated diseases and complications, such as post-COVID, long-COVID, and MIS-C.
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this review.
Ethics approval and consent to participate
Not applicable.
Human and animal rights
Not applicable.
Consent for publication
Not applicable.
Availability of data and materials
Not applicable.
Funding
The work was supported by Xiamen Medical College Research Grant (k2020-07; k2019-01; k2019-03) and Education and Scientific Research Project for Middle-aged and Young Teacher in Fujian Province, Department Education, Fujian (JAT200735 for Xiao-hui Zheng).
CRediT authorship contribution statement
Wan-Yi Ho: Formal analysis. Zi-han Shen: Validation, Supervision, Software, Resources, Project administration, Methodology. Yijing Chen: Visualization, Supervision, Formal analysis. Ting-Hsu Chen: Software, Resources, Project administration. XiaoLin Lu: Data curation. Yaw-Syan Fu: Writing – review & editing, Writing – original draft, Visualization, Data curation.
Declaration of competing interest
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
Footnotes
Supplementary data to this article can be found online at https://doi.org/10.1016/j.heliyon.2024.e30080.
Contributor Information
Wan-Yi Ho, Email: wayehe@kmu.edu.tw.
Zi-han Shen, Email: tzuhamsam@gmail.com.
Yijing Chen, Email: 202003420046@xmmc.edu.cn.
Ting-Hsu Chen, Email: 410613031@gms.ndhu.edu.tw.
XiaoLin Lu, Email: 328499601@qq.com.
Yaw-Syan Fu, Email: m805004@kmu.edu.tw.
Abbreviation
- SARS-CoV-2
Severe acute respiratory syndrome coronavirus 2
- COVID-19
coronavirus infectious disease 2019
- ACE2
angiotensin-converting enzyme 2
- TMPRSS2
transmembrane serine protease 2
- RBD
receptor binding domain
- ORFs
open reading frames
- TRSs
transcription regulatory sequences
- PPs
polyproteins
- PLpro
papain-like proteinase
- 3CLpro
3-chymotrypsin-like protease
- Mpro
main protease
- IFN
type-I interferon
- RTC
replication-transcription complex
- DMVs
double-membrane vesicles
- RTC
replication-transcription complex
- RdRp
RNA-dependent RNA polymerase
- ExoN
N-terminal exonuclease domain
- N7-Mtase
C-terminal guanine-N7 methyltransferase
- NendoU
nidoviral RNA uridylate-specific endoribonuclease
- SAM
S-adenosyl-l-methionine
- 2′-O-MTase
MTase to methylate the RNA cap at ribose 2′-O positions
- Nrf2
nuclear factors erythroid-derived 2-like
- mTOR
mammalian target of rapamycin
- PPARγ
peroxisome proliferator-activated receptor γ
- NF-κB
nuclear factor kappa B
- ERK
extracellular signal-regulated kinases
- eIF2α
elongation initiation factor 2α
- AT1R
ACE-Angiotensin–II–AT1 receptor
- SARs
relevant key structure activity relationships
- YDJDG
Yindan Jiedu granules
- CRS
cytokine release syndrome
- HO-1
heme oxygenase-1
- Keap1
kelch-like ECH-associated protein-1
- ROS
reactive oxygen species
- CC50
50 % cytotoxicity concentration
- IC50
50 % inhibitory concentration
- EGCG
epigallocatechin gallate
- HEJG
herbal extracts of Jingyin granules
- SC
standard care
- LDH
lactate dehydrogenase
- PSM
propensity score matching
- SFJDC
Shufeng Jiedu capsules
- OTC
over-the-counter
- LHQW-C
Lianhuaqingwen capsule
- nsps
non-structure proteins
- SAR
surface activity relationship
- ITC
isothermal titration calorimetry
- MST
microscale thermophoresis
- DARTS
drug affinity responsive target stability
- SPROX
stability of proteins from rates of oxidation
- CETSA
cellular thermal shift assay
- MIS
multisystem inflammatory syndrome
- GI
gastrointestinal
- TSS
toxic shock syndrome
- TCR
T cell receptor
Appendix A. Supplementary data
The following is the Supplementary data to this article:
figs1.

References
- 1.Ciotti M., Angeletti S., Minieri M., et al. COVID-19 outbreak: an overview. Chemotherapy. 2019;64(5–6):215–223. doi: 10.1159/000507423. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 2.Faiyazuddin M., Sophia A., Ashique S., et al. Virulence traits and novel drug delivery strategies for mucormycosis post-COVID-19: a comprehensive review. Front. Immunol. 2023;14 doi: 10.3389/fimmu.2023.1264502. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 3.Hoffmann M., Kleine-Weber H., Schroeder S., et al. SARS-CoV-2 cell entry depends on ACE2 and TMPRSS2 and is blocked by a clinically proven protease inhibitor. Cell. 2020;181(2):271–280. doi: 10.1016/j.cell.2020.02.052. e8. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 4.Kawasumi T., Takeno S., Ishino T., et al. Co-Expression and localization of angiotensin-converting enzyme-2 (ACE2) and the transmembrane serine protease 2 (TMPRSS2) in paranasal ciliated epithelium of patients with chronic Rhinosinusitis. Am. J. Rhinol. Allergy36. 2022;(3):313–322. doi: 10.1177/19458924211059639. [DOI] [PubMed] [Google Scholar]
- 5.Cai J., Zhang H., Zhu K., et al. Risk of reinfection and severity with the predominant BA.5 Omicron subvariant China, from December 2022 to January 2023. Emerg. Microbes. Infect. 2024;13(1) doi: 10.1080/22221751.2023.2292071. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 6.Tey S.F., Tsai Y.W., Wu J.Y., et al. Comparative outcomes of SARS-CoV-2 primary and reinfection in older adult patients. Front. Public Health. 2024;12 doi: 10.3389/fpubh.2024.1337646. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 7.Mohanto S., Faiyazuddin M., Dilip Gholap A., et al. Addressing the resurgence of global monkeypox (Mpox) through advanced drug delivery platforms. Travel Med. Infect. Dis. 2023;56 doi: 10.1016/j.tmaid.2023.102636. [DOI] [PubMed] [Google Scholar]
- 8.Rezaei N., Ashkevarian S., Fathi M.K., et al. Introduction on coronavirus disease (COVID-19) pandemic: the global challenge. Adv. Exp. Med. Biol. 2021;1318:1–22. doi: 10.1007/978-3-030-63761-3_1. [DOI] [PubMed] [Google Scholar]
- 9.Higdon M.M., Wahl B., Jones C.B., et al. A systematic review of coronavirus disease 2019 vaccine efficacy and effectiveness against severe acute respiratory syndrome coronavirus 2 infection and disease. Open Forum Infect. Dis. 2022;9(6):ofac138. doi: 10.1093/ofid/ofac138. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 10.Gorkhali R., Koirala P., Rijal S., et al. Structure and function of major SARS-CoV-2 and SARS-CoV proteins. Bioinform. Biol. Insights. 2021;15 doi: 10.1177/11779322211025876. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 11.Yao H., Song Y., Chen Y., et al. Molecular architecture of the SARS-CoV-2 virus. Cell. 2020;183(3):730–738.e13. doi: 10.1016/j.cell.2020.09.018. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 12.Fehr A.R., Perlman S. Coronaviruses: an overview of their replication and pathogenesis. Methods Mol. Biol. 2015;1282:1–23. doi: 10.1007/978-1-4939-2438-7_1. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 13.Saurabh K., Solovchuk M., Sheu T.W. A detailed study of ion transport through the SARS-CoV-2 E protein ion channel. Nanoscale. 2022;14(23):8291–8305. doi: 10.1039/d2nr01385a. [DOI] [PubMed] [Google Scholar]
- 14.Alam I., Kamau A.A., Kulmanov M., et al. Functional pangenome analysis shows key features of E protein are preserved in SARS and SARS-CoV-2. Front. Cell. Infect. Microbiol. 2020;10:405. doi: 10.3389/fcimb.2020.00405. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 15.Lan J., Ge J., Yu J., et al. Structure of the SARS-CoV-2 spike receptor-binding domain bound to the ACE2 receptor. Nature. 2020;581(7807):215–220. doi: 10.1038/s41586-020-2180-5. [DOI] [PubMed] [Google Scholar]
- 16.Rut W., Lv Z., Zmudzinski M., et al. Activity profiling and crystal structures of inhibitor-bound SARS-CoV-2 papain-like protease: a framework for anti-COVID-19 drug design. Sci. Adv. 2020;6(42) doi: 10.1126/sciadv.abd4596. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 17.Lei X., Dong X., Ma R., et al. Activation and evasion of type I interferon responses by SARS-CoV-2. Nat. Commun. 2020;11(1):3810. doi: 10.1038/s41467-020-17665-9. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 18.Calleja D.J., Lessene G., Komander D. Inhibitors of SARS-CoV-2 PLpro. Front. Chem. 2022;10 doi: 10.3389/fchem.2022.876212. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 19.Rohaim M.A., El Naggar R.F., Clayton E., et al. Structural and functional insights into non-structural proteins of coronaviruses. Microb. Pathog. 2021;150 doi: 10.1016/j.micpath.2020.104641. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 20.Yan F., Gao F. An overview of potential inhibitors targeting non-structural proteins 3 (PLpro and Mac1) and 5 (3CLpro/Mpro) of SARS-CoV-2. Comput. Struct. Biotechnol. J. 2021;19:4868–4883. doi: 10.1016/j.csbj.2021.08.036. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 21.Peng Q., Peng R., Yuan B., et al. Structural and biochemical characterization of the nsp12-nsp7-nsp8 core polymerase complex from SARS-CoV-2. Cell Rep. 2020;31(11) doi: 10.1016/j.celrep.2020.107774. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 22.Khan M.T., Irfan M., Ahsan H., et al. Structures of SARS-CoV-2 RNA-binding proteins and therapeutic targets. Intervirology. 2021;64(2):55–68. doi: 10.1159/000513686. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 23.Yan L., Ge J., Zheng L., et al. Cryo-EM structure of an extended SARS-CoV-2 replication and transcription complex reveals an intermediate state in Cap synthesis. Cell. 2021;184(1):184–193.e10. doi: 10.1016/j.cell.2020.11.016. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 24.Narayanan N., Nair D.T. Ritonavir may inhibit exoribonuclease activity of nsp14 from the SARS-CoV-2 virus and potentiate the activity of chain terminating drugs. Int. J. Biol. Macromol. 2021;168:272–278. doi: 10.1016/j.ijbiomac.2020.12.038. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 25.Viswanathan T., Arya S., Chan S.H., et al. Structural basis of RNA cap modification by SARS-CoV-2. Nat. Commun. 2020;11(1):3718. doi: 10.1038/s41467-020-17496-8. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 26.Yan S., Wu G. Potential 3-chymotrypsin-like cysteine protease cleavage sites in the coronavirus polyproteins pp1a and pp1ab and their possible relevance to COVID-19 vaccine and drug development. FASEB J. 2021;35(5) doi: 10.1096/fj.202100280RR. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 27.Yan L., Zhang Y., Ge J., et al. Architecture of a SARS-CoV-2 mini replication and transcription complex. Nat. Commun. 2020;11(1):5874. doi: 10.1038/s41467-020-19770-1. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 28.Jia Z., Yan L., Ren Z., et al. Delicate structural coordination of the severe acute respiratory syndrome coronavirus Nsp13 upon ATP hydrolysis. Nucleic Acids Res. 2019;47(12):6538–6550. doi: 10.1093/nar/gkz409. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 29.Ma Y., Wu L., Shaw N., et al. Structural basis and functional analysis of the SARS coronavirus nsp14-nsp10 complex. Proc. Natl. Acad. Sci. U.S.A. 2015;112(30):9436–9441. doi: 10.1073/pnas.1508686112. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 30.Romano M., Ruggiero A., Squeglia F., et al. A structural view of SARS-CoV-2 RNA replication machinery: RNA synthesis, proofreading and final capping. Cells. 2020;9(5):1267. doi: 10.3390/cells9051267. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 31.Yan L., Yang Y., Li M., et al. Coupling of N7-methyltransferase and 3'-5' exoribonuclease with SARS-CoV-2 polymerase reveals mechanisms for capping and proofreading. Cell. 2021;184(13):3474–3485.e11. doi: 10.1016/j.cell.2021.05.033. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 32.Hackbart M., Deng X., Baker S.C. Coronavirus endoribonuclease targets viral polyuridine sequences to evade activating host sensors. Proc. Natl. Acad. Sci. U.S.A. 2020;117(14):8094–8103. doi: 10.1073/pnas.1921485117. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 33.Pillon M.C., Frazier M.N., Dillard L.B., et al. Cryo-EM structures of the SARS-CoV-2 endoribonuclease Nsp15 reveal insight into nuclease specificity and dynamics. Nat. Commun. 2021;12(1):636. doi: 10.1038/s41467-020-20608-z. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 34.Chen Y., Su C., Ke M., et al. Biochemical and structural insights into the mechanisms of SARS coronavirus RNA ribose 2'-O-methylation by nsp16/nsp10 protein complex. PLoS Pathog. 2011;7(10) doi: 10.1371/journal.ppat.1002294. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 35.Rosas-Lemus M., Minasov G., Shuvalova L., et al. High-resolution structures of the SARS-CoV-2 2'-O-methyltransferase reveal strategies for structure-based inhibitor design. Sci. Signal. 2020;13(651) doi: 10.1126/scisignal.abe1202. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 36.Nishimuro H., Ohnishi H., Sato M., et al. Estimated daily intake and seasonal food sources of quercetin in Japan. Nutrients. 2015;7(4):2345–2358. doi: 10.3390/nu7042345. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 37.Bhagwat S., Haytowitz D.B. USDA database for the flavonoid content of selected foods, Release 3.3 (March 2018) 2022. [DOI]
- 38.Carrasco-Pozo C., Tan K.N., Reyes-Farias M., et al. The deleterious effect of cholesterol and protection by quercetin on mitochondrial bioenergetics of pancreatic β-cells, glycemic control and inflammation: In vitro and in vivo studies. Redox Biol. 2016;9:229–243. doi: 10.1016/j.redox.2016.08.007. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 39.Carullo G., Cappello A.R., Frattaruolo L., et al. Quercetin and derivatives: useful tools in inflammation and pain management. Future Med. Chem. 2017;9(1):79–93. doi: 10.4155/fmc-2016-0186. [DOI] [PubMed] [Google Scholar]
- 40.Aguirre L., Arias N., Macarulla M.T., et al. Beneficial effects of quercetin on obesity and diabetes. Open Nutraceuticals J. 2011;4:189–198. [Google Scholar]
- 41.Rauf A., Imran M., Khan I.A., et al. Anticancer potential of quercetin: a comprehensive review. Phytother Res. 2018;32(11):2109–2130. doi: 10.1002/ptr.6155. [DOI] [PubMed] [Google Scholar]
- 42.Xu D., Hu M.J., Wang Y.Q., et al. Antioxidant activities of quercetin and its complexes for medicinal application. Molecules24. 2019;(6):1123. doi: 10.3390/molecules24061123. Published 2019 Mar 21. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 43.Saeedi-Boroujeni A., Mahmoudian-Sani M.R. Anti-inflammatory potential of quercetin in COVID-19 treatment. J. Inflamm. 2021;18(1):3. doi: 10.1186/s12950-021-00268-6. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 44.Oboh G., Ademosun A.O., Ogunsuyi O.B. Quercetin and its role in chronic diseases. Adv. Exp. Med. Biol. 2016;929:377–387. doi: 10.1007/978-3-319-41342-6_17. [DOI] [PubMed] [Google Scholar]
- 45.Azuma M., Dat Le T., Yoshimoto Y., et al. RNA-seq analysis of diet-driven obesity and anti-obesity effects of quercetin glucoside or epigallocatechin gallate in Drosophila adults. Eur. Rev. Med. Pharmacol. Sci. 2019;23(2):857–876. doi: 10.26355/eurrev_201901_16901. [DOI] [PubMed] [Google Scholar]
- 46.Koshinaka K., Honda A., Masuda H., et al. Effect of quercetin treatment on mitochondrial biogenesis and exercise-induced AMP-activated protein kinase activation in rat skeletal muscle. Nutrients. 2020;12(3):729. doi: 10.3390/nu12030729. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 47.Zaragozá C., Monserrat J., Mantecón C., et al. Binding and antiplatelet activity of quercetin, rutin, diosmetin, and diosmin flavonoids. Biomed. Pharmacother. 2021;141 doi: 10.1016/j.biopha.2021.111867. [DOI] [PubMed] [Google Scholar]
- 48.Manzoor M.F., Hussain A., Sameen A., et al. Novel extraction, rapid assessment and bioavailability improvement of quercetin: a review, Ultrason. Sonochem. 2021;78 doi: 10.1016/j.ultsonch.2021.105686. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 49.Aytac Z., Kusku S.I., Durgun E., et al. Quercetin/β-cyclodextrin inclusion complex embedded nanofibres: slow release and high solubility. Food Chem. 2016;197(Pt A):864–871. doi: 10.1016/j.foodchem.2015.11.051. [DOI] [PubMed] [Google Scholar]
- 50.Di Petrillo A., Orrù G., Fais A., et al. Quercetin and its derivates as antiviral potentials: a comprehensive review. Phytother Res. 2022;36(1):266–278. doi: 10.1002/ptr.7309. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 51.Iddir M., Brito A., Dingeo G., et al. Strengthening the immune system and reducing inflammation and oxidative stress through diet and nutrition: considerations during the COVID-19 Crisis. Nutrients. 2020;12(6):1562. doi: 10.3390/nu12061562. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 52.Cuadrado A., Pajares M., Benito C., et al. Can activation of NRF2 be a strategy against COVID-19? Trends Pharmacol. Sci. 2020;41(9):598–610. doi: 10.1016/j.tips.2020.07.003. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 53.Bousquet J., Cristol J.P., Czarlewski W., et al. Nrf2-interacting nutrients and COVID-19: time for research to develop adaptation strategies. Clin. Transl. Allergy. 2020;10(1):58. doi: 10.1186/s13601-020-00362-7. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 54.Fu Y.S., Kang N., Yu Y., et al. Polyphenols, flavonoids and inflammasomes: the role of cigarette smoke in COPD. Eur. Respir. Rev. 2022;31(164) doi: 10.1183/16000617.0028-2022. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 55.Manjunath S.H., Thimmulappa R.K. Antiviral, immunomodulatory, and anticoagulant effects of quercetin and its derivatives: potential role in prevention and management of COVID-19. J. Pharm. Anal. 2022;12(1):29–34. doi: 10.1016/j.jpha.2021.09.009. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 56.Kumar Verma A., Kumar V., Singh S., et al. Repurposing potential of Ayurvedic medicinal plants derived active principles against SARS-CoV-2 associated target proteins revealed by molecular docking, molecular dynamics and MM-PBSA studies. Biomed. Pharmacother. 2021;137 doi: 10.1016/j.biopha.2021.111356. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 57.Di Petrillo A., Santos-Buelga C., Era B., et al. Sardinian honeys as sources of xanthine oxidase and tyrosinase inhibitors. Food Sci. Biotechnol. 2017;27(1):139–146. doi: 10.1007/s10068-017-0275-z. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 58.Singh S., Florez H. Coronavirus disease 2019 drug discovery through molecular docking. F1000Res. 2020;9:502. doi: 10.12688/f1000research.24218.1. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 59.Izzo A.A., Hoon-Kim S., Radhakrishnan R., et al. A critical approach to evaluating clinical efficacy, adverse events and drug interactions of herbal remedies. Phytother Res. 2016;30(5):691–700. doi: 10.1002/ptr.5591. [DOI] [PubMed] [Google Scholar]
- 60.Lin J.F., Fan L.L., Li B.W., et al. A study to evaluate herb-drug interaction underlying mechanisms: an investigation of ginsenosides attenuating the effect of warfarin on cardiovascular diseases. Eur. J. Pharm. Sci. 2020;142 doi: 10.1016/j.ejps.2019.105100. [DOI] [PubMed] [Google Scholar]
- 61.Sharad S., Kapur S. Indian herb-derived phytoconstituent-based antiviral, antimicrobial and antifungal formulation: an oral rinse candidate for oral hygiene and the potential prevention of COVID-19 outbreaks. Pathogens. 2021;10(9):1130. doi: 10.3390/pathogens10091130. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 62.Kandeel M., Kitade Y., Almubarak A. Repurposing FDA-approved phytomedicines, natural products, antivirals and cell protectives against SARS-CoV-2 (COVID-19) RNA-dependent RNA polymerase. PeerJ. 2020;8 doi: 10.7717/peerj.10480. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 63.Souid I., Korchef A., Souid S. In silico evaluation of Vitis amurensis Rupr. polyphenol compounds for their inhibition potency against CoVID-19 main enzymes Mpro and RdRp. Saudi. Pharm. J. 2022;30(5):570–584. doi: 10.1016/j.jsps.2022.02.014. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 64.Septembre-Malaterre A., Boumendjel A., Seteyen A.S., et al. Focus on the high therapeutic potentials of quercetin and its derivatives. Phytomed Plus. 2022;2(1) doi: 10.1016/j.phyplu.2022.100220. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 65.Shaldam M.A., Yahya G., Mohamed N.H., et al. In silico screening of potent bioactive compounds from honeybee products against COVID-19 target enzymes. Environ. Sci. Pollut. Res. Int. 2021;28(30):40507–40514. doi: 10.1007/s11356-021-14195-9. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 66.Shah S., Chaple D., Arora S., et al. Prospecting for Cressa cretica to treat COVID-19 via in silico molecular docking models of the SARS-CoV-2. J. Biomol. Struct. Dyn. 2022;40(12):5643–5652. doi: 10.1080/07391102.2021.1872419. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 67.Vijayakumar B.G., Ramesh D., Joji A., et al. In silico pharmacokinetic and molecular docking studies of natural flavonoids and synthetic indole chalcones against essential proteins of SARS-CoV-2. Eur. J. Pharmacol. 2020;886 doi: 10.1016/j.ejphar.2020.173448. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 68.Khan J., Sakib S.A., Mahmud S., et al. Identification of potential phytochemicals from Citrus Limon against main protease of SARS-CoV-2: molecular docking, molecular dynamic simulations and quantum computations. J. Biomol. Struct. Dyn. 2022;40(21):10741–10752. doi: 10.1080/07391102.2021.1947893. [DOI] [PubMed] [Google Scholar]
- 69.Bahun M., Jukić M., Oblak D., et al. Inhibition of the SARS-CoV-2 3CLpro main protease by plant polyphenols. Food Chem. 2022;373(Pt B) doi: 10.1016/j.foodchem.2021.131594. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 70.Majumder R., Mandal M. Screening of plant-based natural compounds as a potential COVID-19 main protease inhibitor: an in silico docking and molecular dynamics simulation approach. J. Biomol. Struct. Dyn. 2022;40(2):696–711. doi: 10.1080/07391102.2020.1817787. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 71.Zhu Y., Scholle F., Kisthardt S.C., et al. Flavonols and dihydroflavonols inhibit the main protease activity of SARS-CoV-2 and the replication of human coronavirus 229E. Virology. 2022;571:21–33. doi: 10.1016/j.virol.2022.04.005. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 72.Oso B.J., Olaoye I.F., Omeike S.O. Molecular docking and ADMET prediction of natural compounds towards SARS spike glycoprotein-human angiotensin-converting enzyme 2 and SARS-CoV-2 main protease. Arch. Razi. Inst. 2021;76(3):453–459. doi: 10.22092/ari.2020.351202.1517. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 73.Sharma A., Goyal S., Yadav A.K., et al. In-silico screening of plant-derived antivirals against main protease, 3CLpro and endoribonuclease, NSP15 proteins of SARS-CoV-2. J. Biomol. Struct. Dyn. 2022;40(1):86–100. doi: 10.1080/07391102.2020.1808077. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 74.Rehman M.T., Alajmi M.F., Hussain A. Natural compounds as inhibitors of SARS-CoV-2 main protease (3CLpro): a molecular docking and simulation approach to combat COVID-19. Curr Pharm Des. 2021;27(33):3577–3589. doi: 10.2174/1381612826999201116195851. [DOI] [PubMed] [Google Scholar]
- 75.Hiremath S., Kumar H.D.V., Nandan M., et al. In silico docking analysis revealed the potential of phytochemicals present in Phyllanthus amarus and Andrographis paniculata, used in Ayurveda medicine in inhibiting SARS-CoV-2. 3 Biotech. 2021;11(2):44. doi: 10.1007/s13205-020-02578-7. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 76.Pandey P., Rane J.S., Chatterjee A., et al. Targeting SARS-CoV-2 spike protein of COVID-19 with naturally occurring phytochemicals: an in silico study for drug development. J. Biomol. Struct. Dyn. 2021;39(16):6306–6316. doi: 10.1080/07391102.2020.1796811. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 77.Maurya V.K., Kumar S., Prasad A.K., et al. Structure-based drug designing for potential antiviral activity of selected natural products from Ayurveda against SARS-CoV-2 spike glycoprotein and its cellular receptor. Virusdisease. 2020;31(2):179–193. doi: 10.1007/s13337-020-00598-8. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 78.Fu Y.S., Ho W.Y., Kang N., et al. Pharmaceutical prospects of curcuminoids for the remedy of COVID-19: truth or myth. Front. Pharmacol. 2022;13 doi: 10.3389/fphar.2022.863082. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 79.Corona A., Wycisk K., Talarico C., et al. Natural compounds inhibit SARS-CoV-2 nsp13 unwinding and ATPase enzyme activities. ACS Pharmacol. Transl. Sci. 2022;5(4):226–239. doi: 10.1021/acsptsci.1c00253. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 80.Liu X., Fang P., Fang L., et al. Porcine deltacoronavirus nsp15 antagonizes interferon-β production independently of its endoribonuclease activity. Mol. Immunol. 2019;114:100–107. doi: 10.1016/j.molimm.2019.07.003. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 81.Saliu T.P., Umar H.I., Ogunsile O.J., et al. Molecular docking and pharmacokinetic studies of phytocompounds from Nigerian Medicinal Plants as promising inhibitory agents against SARS-CoV-2 methyltransferase (nsp16) J. Genet. Eng. Biotechnol. 2021;19(1):172. doi: 10.1186/s43141-021-00273-5. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 82.Omotuyi I.O., Nash O., Ajiboye B.O., et al. Aframomum melegueta secondary metabolites exhibit polypharmacology against SARS-CoV-2 drug targets: in vitro validation of furin inhibition. Phytother Res. 2021;35(2):908–919. doi: 10.1002/ptr.6843. [DOI] [PubMed] [Google Scholar]
- 83.Zothantluanga J.H., Gogoi N., Shakya A., et al. Computational guided identification of potential leads from Acacia pennata (L.) Willd. as inhibitors for cellular entry and viral replication of SARS-CoV-2. Futur. J. Pharm. Sci. 2021;7(1):201. doi: 10.1186/s43094-021-00348-7. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 84.da Silva F.M.A., da Silva K.P.A., de Oliveira L.P.M., et al. Flavonoid glycosides and their putative human metabolites as potential inhibitors of the SARS-CoV-2 main protease (Mpro) and RNA-dependent RNA polymerase (RdRp) Mem. Inst. Oswaldo Cruz. 2020;115 doi: 10.1590/0074-02760200207. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 85.Fadaka A.O., Sibuyi N.R.S., Martin D.R., et al. Development of effective therapeutic molecule from natural sources against coronavirus protease. Int. J. Mol. Sci. 2021;22(17):9431. doi: 10.3390/ijms22179431. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 86.Kushwaha P.P., Singh A.K., Bansal T., et al. Identification of natural inhibitors against SARS-CoV-2 drugable targets using molecular docking, molecular dynamics simulation, and MM-PBSA approach. Front. Cell. Infect. Microbiol. 2021;11 doi: 10.3389/fcimb.2021.730288. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 87.Bhattacharya K., Bordoloi R., Chanu N.R., et al. In silico discovery of 3 novel quercetin derivatives against papain-like protease, spike protein, and 3C-like protease of SARS-CoV-2. J. Genet. Eng. Biotechnol. 2022;20(1):43. doi: 10.1186/s43141-022-00314-7. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 88.Ferdous N., Reza M.N., Islam M.S., et al. Newly designed analogues from SARS-CoV inhibitors mimicking the druggable properties against SARS-CoV-2 and its novel variants. RSC Adv. 2021;11(50):31460–31476. doi: 10.1039/d1ra04107j. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 89.Mbikay M., Chrétien M. Isoquercetin as an anti-COVID-19 medication: a potential to realize. Front. Pharmacol. 2022;13 doi: 10.3389/fphar.2022.830205. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 90.Umar A.K. Flavonoid compounds of buah merah (Pandanus conoideus Lamk) as a potent SARS-CoV-2 main protease inhibitor: in silico approach. Futur. J. Pharm. Sci. 2021;7(1):158. doi: 10.1186/s43094-021-00309-0. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 91.Rutwick Surya U., Praveen N. A molecular docking study of SARS-CoV-2 main protease against phytochemicals of Boerhavia diffusa Linn. for novel COVID-19 drug discovery. Virusdisease. 2021;32(1):46–54. doi: 10.1007/s13337-021-00683-6. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 92.Şimşek Y., Baran S.S., Aslım B. In silico identification of SARS-CoV-2 cell entry inhibitors from selected natural antivirals. J. Mol. Graph. Model. 2021;109 doi: 10.1016/j.jmgm.2021.108038. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 93.Hassan H.A., Hassan A.R., Mohamed E.A.R., et al. Conducting the RBD of SARS-CoV-2 omicron variant with phytoconstituents from Euphorbia dendroides to repudiate the binding of spike glycoprotein using computational molecular search and simulation approach. Molecules. 2022;27(9):2929. doi: 10.3390/molecules27092929. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 94.Milanović Ž.B., Antonijević M.R., Amić A.D., et al. Inhibitory activity of quercetin, its metabolite, and standard antiviral drugs towards enzymes essential for SARS-CoV-2: the role of acid-base equilibria. RSC Adv. 2021;11(5):2838–2847. doi: 10.1039/d0ra09632f. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 95.Hossain R., Sarkar C., Hassan S.M.H., et al. In silico screening of natural products as potential inhibitors of SARS-CoV-2 using molecular docking simulation. Chin. J. Integr. Med. 2022;28(3):249–256. doi: 10.1007/s11655-021-3504-5. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 96.Pan B., Fang S., Zhang J., et al. Chinese herbal compounds against SARS-CoV-2: puerarin and quercetin impair the binding of viral S-protein to ACE2 receptor. Comput. Struct. Biotechnol. J. 2020;18:3518–3527. doi: 10.1016/j.csbj.2020.11.010. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 97.Guler H.I., Tatar G., Yildiz O., et al. Investigation of potential inhibitor properties of ethanolic propolis extracts against ACE-II receptors for COVID-19 treatment by molecular docking study. Arch. Microbiol. 2021;203(6):3557–3564. doi: 10.1007/s00203-021-02351-1. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 98.Singh R., Bhardwaj V., Das P., et al. Natural analogues inhibiting selective cyclin-dependent kinase protein isoforms: a computational perspective. J. Biomol. Struct. Dyn. 2020;38(17):5126–5135. doi: 10.1080/07391102.2019.1696709. [DOI] [PubMed] [Google Scholar]
- 99.Oyedara O.O., Agbedahunsi J.M., Adeyemi F.M., et al. Computational screening of phytochemicals from three medicinal plants as inhibitors of transmembrane protease serine 2 implicated in SARS-CoV-2 infection. Phytomed. Plus. 2021;1(4) doi: 10.1016/j.phyplu.2021.100135. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 100.Manjunathan R., Periyaswami V., Mitra K., et al. Molecular docking analysis reveals the functional inhibitory effect of genistein and quercetin on TMPRSS2: SARS-COV-2 cell entry facilitator spike protein. BMC Bioinf. 2022;23(1):180. doi: 10.1186/s12859-022-04724-9. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 101.Hasanvand A. COVID-19 and the role of cytokines in this disease. Inflammopharmacology. 2022;30(3):789–798. doi: 10.1007/s10787-022-00992-2. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 102.Albutti A. Rescuing the host immune system by targeting the immune evasion complex ORF8-IRF3 in SARS-CoV-2 infection with natural products using molecular modeling approaches. Int. J. Environ. Res. Public Health. 2021;19(1):112. doi: 10.3390/ijerph19010112. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 103.Chaudhari A.M., Singh I., Joshi M., et al. Defective ORF8 dimerization in SARS-CoV-2 delta variant leads to a better adaptive immune response due to abrogation of ORF8-MHC1 interaction. Mol. Divers. 2023;27(1):45–57. doi: 10.1007/s11030-022-10405-9. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 104.Chanjitwiriya K., Roytrakul S., Kunthalert D. Quercetin negatively regulates IL-1β production in Pseudomonas aeruginosa-infected human macrophages through the inhibition of MAPK/NLRP3 inflammasome pathways. PLoS One. 2020;15(8) doi: 10.1007/s11030-022-10405-9. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 105.Zhu J., Xue X., He Z., et al. Using network pharmacology and molecular docking to explore the underlying anti-inflammatory mechanism of Wuyao-Danshen to treat endometriosis. Ann. Transl. Med. 2022;10(4):198. doi: 10.21037/atm-22-419. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 106.Wang L., Wang Y., Yang W., et al. Network pharmacology and molecular docking analysis on mechanisms of Tibetan Hongjingtian (Rhodiola crenulata) in the treatment of COVID-19. J. Med. Microbiol. 2021;70(7) doi: 10.1099/jmm.0.001374. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 107.He D.D., Zhang X.K., Zhu X.Y., et al. Network pharmacology and RNA-sequencing reveal the molecular mechanism of Xuebijing injection on COVID-19-induced cardiac dysfunction. Comput. Biol. Med. 2021;131 doi: 10.1016/j.compbiomed.2021.104293. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 108.Wang L., Chen J., Wang B., et al. Protective effect of quercetin on lipopolysaccharide-induced acute lung injury in mice by inhibiting inflammatory cell influx. Exp. Biol. Med. (Maywood) 2014;239(12):1653–1662. doi: 10.1177/1535370214537743. [DOI] [PubMed] [Google Scholar]
- 109.Takashima K., Matsushima M., Hashimoto K., et al. Protective effects of intratracheally administered quercetin on lipopolysaccharide-induced acute lung injury. Respir. Res. 2014;15(1):150. doi: 10.1186/s12931-014-0150-x. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 110.Ji L.L., Sheng Y.C., Zheng Z.Y., et al. The involvement of p62-Keap1-Nrf2 antioxidative signaling pathway and JNK in the protection of natural flavonoid quercetin against hepatotoxicity. Free Radic. Biol. Med. 2015;85:12–23. doi: 10.1016/j.freeradbiomed.2015.03.035. [DOI] [PubMed] [Google Scholar]
- 111.Ren J., Liao L., Shang S., et al. Purification, characterization, and bioactivities of polyphenols from Platycladus orientalis (L.) Franco. J. Food Sci. 2019;84(3):667–677. doi: 10.1111/1750-3841.14483. [DOI] [PubMed] [Google Scholar]
- 112.Zhuang Z., Zhong X., Zhang H., et al. Exploring the potential mechanism of Shufeng Jiedu capsule for treating COVID-19 by comprehensive network pharmacological approaches and molecular docking validation. Comb. Chem. High Throughput Screen. 2021;24(9):1377–1394. doi: 10.2174/1386207323999201029122301. [DOI] [PubMed] [Google Scholar]
- 113.Kandeil A., Mostafa A., Kutkat O. Bioactive polyphenolic compounds showing strong antiviral activities against severe acute respiratory syndrome coronavirus 2. Pathogens. 2021;10(6):758. doi: 10.3390/pathogens10060758. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 114.Zhan Y., Ta W., Tang W., et al. Potential antiviral activity of isorhamnetin against SARS-CoV-2 spike pseudotyped virus in vitro. Drug Dev. Res. 2021;82(8):1124–1130. doi: 10.1002/ddr.21815. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 115.Liu X., Raghuvanshi R., Ceylan F.D., et al. Quercetin and its metabolites inhibit recombinant human angiotensin-converting enzyme 2 (ACE2) activity. J. Agric. Food Chem. 2020;68(47):13982–13989. doi: 10.1021/acs.jafc.0c05064. [DOI] [PubMed] [Google Scholar]
- 116.Amin S.A., Banerjee S., Ghosh K., et al. Protease targeted COVID-19 drug discovery and its challenges: insight into viral main protease (Mpro) and papain-like protease (PLpro) inhibitors. Bioorg. Med. Chem. 2021;29 doi: 10.1016/j.bmc.2020.115860. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 117.Mangiavacchi F., Botwina P., Menichetti E., et al. Seleno-functionalization of quercetin improves the non-covalent inhibition of Mpro and its antiviral activity in cells against SARS-CoV-2. Int. J. Mol. Sci. 2021;22(13):7048. doi: 10.3390/ijms22137048. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 118.Rizzuti B., Grande F., Conforti F., et al. Rutin is a low micromolar inhibitor of SARS-CoV-2 main protease 3CLpro: implications for drug design of quercetin analogs. Biomedicines. 2021;9(4):375. doi: 10.3390/biomedicines9040375. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 119.Sancineto L., Ostacolo C., Ortega-Alarcon D., et al. L-arginine improves solubility and anti SARS-CoV-2 Mpro activity of rutin but not the antiviral activity in cells. Molecules. 2021;26(19):6062. doi: 10.3390/molecules26196062. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 120.Sakshi C., Harikrishnan A., Jayaraman S., et al. Predictive medicinal metabolites from Momordica dioica against comorbidity related proteins of SARS-CoV-2 infections. J. Biomol. Struct. Dyn. 2022;40(11):5175–5188. doi: 10.1080/07391102.2020.1868340. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 121.Frazier M.N., Dillard L.B., Krahn J.M., et al. Characterization of SARS2 Nsp15 nuclease activity reveals it's mad about U. Nucleic Acids Res. 2021;49(17):10136–10149. doi: 10.1093/nar/gkab719. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 122.Hong S., Seo S.H., Woo S.J., et al. Epigallocatechin gallate inhibits the uridylate-specific endoribonuclease Nsp15 and efficiently neutralizes the SARS-CoV-2 strain. J. Agric. Food Chem. 2021;69(21):5948–5954. doi: 10.1021/acs.jafc.1c02050. [DOI] [PubMed] [Google Scholar]
- 123.Goc A., Niedzwiecki A., Ivanov V., et al. Inhibitory effects of specific combination of natural compounds against SARS-CoV-2 and its alpha, Beta, gamma, delta, kappa, and mu variants. Eur. J. Microbiol. Immunol. (Bp) 2022;11(4):87–94. doi: 10.1556/1886.2021.00022. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 124.Ryu Y.B., Jeong H.J., Kim J.H., et al. Biflavonoids from Torreya nucifera displaying SARS-CoV 3CLpro inhibition. Bioorg. Med. Chem. 2010;18(22):7940–7947. doi: 10.1016/j.bmc.2010.09.035. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 125.Abian O., Ortega-Alarcon D., Jimenez-Alesanco A. Structural stability of SARS-CoV-2 3CLpro and identification of quercetin as an inhibitor by experimental screening. Int. J. Biol. Macromol. 2020;164:1693–1703. doi: 10.1016/j.ijbiomac.2020.07.235. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 126.Zhang X., Gao R., Zhou Z., et al. A network pharmacology based approach for predicting active ingredients and potential mechanism of Lianhuaqingwen capsule in treating COVID-19. Int. J. Med. Sci. 2021;18(8):1866–1876. doi: 10.7150/ijms.53685. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 127.Zhang F., Liu W., Huang J., et al. Inhibition of drug-metabolizing enzymes by Jingyin granules: implications of herb-drug interactions in antiviral therapy. Acta Pharmacol. Sin. 2022;43(4):1072–1081. doi: 10.1038/s41401-021-00697-2. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 128.Di Pierro F., Derosa G., Maffioli P., et al. Possible therapeutic effects of adjuvant quercetin supplementation against early-stage COVID-19 infection: a prospective, randomized, controlled, and open-label study. Int. J. Gen. Med. 2021;14:2359–2366. doi: 10.2147/IJGM.S318720. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 129.Di Pierro F., Iqtadar S., Khan A., et al. Potential clinical benefits of quercetin in the early stage of COVID-19: results of a second, pilot, randomized, controlled and open-label clinical trial. Int. J. Gen. Med. 2021;14:2807–2816. doi: 10.2147/IJGM.S318949. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 130.Shohan M., Nashibi R., Mahmoudian-Sani M.R., et al. The therapeutic efficacy of quercetin in combination with antiviral drugs in hospitalized COVID-19 patients: a randomized controlled trial. Eur. J. Pharmacol. 2022;914 doi: 10.1016/j.ejphar.2021.174615. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 131.Feng Y., Zhu B., Liu Y., et al. Yindan Jiedu granules exhibit anti-inflammatory effect in patients with novel Coronavirus disease (COVID-19) by suppressing the NF-κB signaling pathway. Phytomedicine. 2022;95 doi: 10.1016/j.phymed.2021.153784. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 132.Xia L., Shi Y., Su J., et al. Shufeng Jiedu, a promising herbal therapy for moderate COVID-19: antiviral and anti-inflammatory properties, pathways of bioactive compounds, and a clinical real-world pragmatic study. Phytomedicine. 2021;85 doi: 10.1016/j.phymed.2020.153390. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 133.Margolin L., Luchins J., Margolin D., et al. 20-Week study of clinical outcomes of over-the-counter COVID-19 prophylaxis and treatment, J. Evid. Based Integr. Med. 2021;26 doi: 10.1177/2515690X211026193. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 134.Glinsky G.V. Tripartite combination of candidate pandemic mitigation agents:Vitamin D, quercetin, and estradiol manifest properties of medicinal agents for targeted mitigation of the COVID-19 pandemic defined by genomics-guided tracing of SARS-CoV-2 targets in human cells. Biomedicines. 2020;8(5):129. doi: 10.3390/biomedicines8050129. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 135.Chapman R.L., Andurkar S.V. A review of natural products, their effects on SARS-CoV-2 and their utility as lead compounds in the discovery of drugs for the treatment of COVID-19. Med. Chem. Res. 2022;31(1):40–51. doi: 10.1007/s00044-021-02826-2. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 136.Di Pierro F., Khan A., Iqtadar S., et al. Quercetin as a possible complementary agent for early-stage COVID-19: concluding results of a randomized clinical trial. Front. Pharmacol. 2023;13 doi: 10.3389/fphar.2022.1096853. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 137.Gérain J., Uebelhoer M., Costes B., et al. NASAFYTOL® supplementation in adults hospitalized with COVID-19 infection: results from an exploratory open-label randomized controlled trial. Front. Nutr. 2023;10 doi: 10.3389/fnut.2023.1137407. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 138.Khan A., Iqtadar S., Mumtaz S.U., et al. Oral co-supplementation of curcumin, quercetin, and vitamin D3 as an adjuvant therapy for mild to moderate symptoms of COVID-19-results from a pilot open-label, randomized controlled trial. Front. Pharmacol. 2022;13 doi: 10.3389/fphar.2022.898062. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 139.Ujjan I.D., Khan S., Nigar R., et al. The possible therapeutic role of curcumin and quercetin in the early-stage of COVID-19-Results from a pragmatic randomized clinical trial. Front. Nutr. 2023;9 doi: 10.3389/fnut.2022.1023997. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 140.Khazeei Tabari M.A., Iranpanah A., Bahramsoltani R., et al. Flavonoids as promising antiviral agents against SARS-CoV-2 infection: a mechanistic review. Molecules. 2021;26(13):3900. doi: 10.3390/molecules26133900. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 141.Ruan X., Du P., Zhao K., et al. Mechanism of Dayuanyin in the treatment of coronavirus disease 2019 based on network pharmacology and molecular docking. Chin. Med. 2020;15:62. doi: 10.1186/s13020-020-00346-6. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 142.Kong R., Yang G., Xue R., et al. COVID-19 docking server: a meta server for docking small molecules, peptides and antibodies against potential targets of COVID-19. Bioinformatics. 2020;36(20):5109–5111. doi: 10.1093/bioinformatics/btaa645. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 143.Rivero-Segura N.A., Gomez-Verjan J.C. In silico screening of natural products isolated from Mexican herbal medicines against COVID-19. Biomolecules. 2021;11(2):216. doi: 10.3390/biom11020216. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 144.Khan S., Hussain A., Vahdani Y., et al. Exploring the interaction of quercetin-3-O-sophoroside with SARS-CoV-2 main proteins by theoretical studies: a probable prelude to control some variants of coronavirus including Delta. Arab. J. Chem. 2021;14(10) doi: 10.1016/j.arabjc.2021.103353. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 145.Verma S., Pandey A.K. Factual insights of the allosteric inhibition mechanism of SARS-CoV-2 main protease by quercetin: an in silico analysis. 3 Biotech. 2021;11(2):67. doi: 10.1007/s13205-020-02630-6. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 146.Muroi M., Osada H. Proteomics-based target identification of natural products affecting cancer metabolism. J. Antibiot. (Tokyo) 2021;74(10):639–650. doi: 10.1038/s41429-021-00437-y. [DOI] [PubMed] [Google Scholar]
- 147.Ye M., Luo G., Ye D., et al. Network pharmacology, molecular docking integrated surface plasmon resonance technology reveals the mechanism of Toujie Quwen Granules against coronavirus disease 2019 pneumonia. Phytomedicine. 2019;85 doi: 10.1016/j.phymed.2020.153401. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 148.Chen I.Y., Chang S.C., Wu H.Y., et al. Upregulation of the chemokine (C-C motif) ligand 2 via a severe acute respiratory syndrome coronavirus spike-ACE2 signaling pathway. J. Virol. 2010;84(15):7703–7712. doi: 10.1128/JVI.02560-09. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 149.Bernini R., Velotti F. Natural polyphenols as immunomodulators to rescue immune response homeostasis: quercetin as a research model against severe COVID-19. Molecules. 2021;26(19):5803. doi: 10.3390/molecules26195803. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 150.Limanaqi F., Busceti C.L., Biagioni F., et al. Cell clearing systems as targets of polyphenols in viral infections: potential implications for COVID-19 pathogenesis. Antioxidants. 2020;9(11):1105. doi: 10.3390/antiox9111105. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 151.Swain S.S., Singh S.R., Sahoo A., et al. Anti-HIV-drug and phyto-flavonoid combination against SARS-CoV-2: a molecular docking-simulation base assessment. J. Biomol. Struct. Dyn. 2022;40(14):6463–6476. doi: 10.1080/07391102.2021.1885495. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 152.Bardelčíková A., Miroššay A., Šoltýs J., et al. Therapeutic and prophylactic effect of flavonoids in post-COVID-19 therapy. Phytother Res. 2022;36(5):2042–2060. doi: 10.1002/ptr.7436. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 153.Theoharides T.C., Cholevas C., Polyzoidis K., et al. Long-COVID syndrome-associated brain fog and chemofog: luteolin to the rescue. Biofactors. 2021;47(2):232–241. doi: 10.1002/biof.1726. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 154.Theoharides T.C., Lauritano D., Ronconi G., et al. Antibodies for COVID-19 - which, when and how long? J. Biol. Regul. Homeost. Agents. 2021;35(2):417–422. doi: 10.23812/Theo_edit. [DOI] [PubMed] [Google Scholar]
- 155.Theoharides T.C. Could SARS-CoV-2 spike protein be responsible for long-COVID syndrome? Mol. Neurobiol. 2022;59(3):1850–1861. doi: 10.1007/s12035-021-02696-0. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 156.Algarni A.S., Alamri N.M., Khayat N.Z., et al. Clinical practice guidelines in multisystem inflammatory syndrome (MIS-C) related to COVID-19: a critical review and recommendations. World J. Pediatr. 2022;18(2):83–90. doi: 10.1007/s12519-021-00499-w. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 157.Ish P., Kunal S., Sakthivel P. MIS-A after COVID-19: points to ponder. Indian J. Crit. Care Med. 2022;26(4):531. doi: 10.5005/jp-journals-10071-24180. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 158.Patel J.M. Multisystem inflammatory syndrome in children (MIS-C) Curr. Allergy Asthma Rep. 2022;22(5):53–60. doi: 10.1007/s11882-022-01031-4. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 159.Santos M.O., Gonçalves L.C., Silva P.A.N., et al. Multisystem inflammatory syndrome (MIS-C): a systematic review and meta-analysis of clinical characteristics, treatment, and outcomes. J. Pediatr. 2022;98(4):338–349. doi: 10.1016/j.jped.2021.08.006. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 160.Bukulmez H. Current understanding of multisystem inflammatory syndrome (MIS-C) following COVID-19 and its distinction from Kawasaki disease. Curr. Rheumatol. Rep. 2021;23(8):58. doi: 10.1007/s11926-021-01028-4. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 161.Giacalone M., Scheier E., Shavit I. Multisystem inflammatory syndrome in children (MIS-C): a mini-review. Int. J. Emerg. Med. 2021;14(1):50. doi: 10.1186/s12245-021-00373-6. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 162.Porritt R.A., Paschold L., Rivas M.N., et al. HLA class I-associated expansion of TRBV11-2 T cells in multisystem inflammatory syndrome in children. J. Clin. Invest. 2021;131(10) doi: 10.1172/JCI146614. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 163.Yong S.J. Long COVID or post-COVID-19 syndrome: putative pathophysiology, risk factors, and treatments. Infect. Dis. (Lond) 2021;53(10):737–754. doi: 10.1080/23744235.2021.1924397. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 164.Parums D.V. Editorial: multisystem inflammatory syndrome in adults (MIS-A) and the spectrum of COVID-19. Med. Sci. Monit. 2021;27 doi: 10.12659/MSM.935005. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 165.Tao Q., Du J., Li X., et al. Network pharmacology and molecular docking analysis on molecular targets and mechanisms of Huashi Baidu formula in the treatment of COVID-19. Drug Dev. Ind. Pharm. 2020;46(8):1345–1353. doi: 10.1080/03639045.2020.1788070. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 166.Xiong H., Dong Z., Lou G., et al. Analysis of the mechanism of Shufeng Jiedu capsule prevention and treatment for COVID-19 by network pharmacology tools. Eur. J. Integr. Med. 2020;40 doi: 10.1016/j.eujim.2020.101241. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 167.Arokiyaraj S., Stalin A., Kannan B.S., et al. Geranii Herba as a potential inhibitor of SARS-CoV-2 main 3CLpro, spike RBD, and regulation of unfolded protein response: an in silico approach. Antibiotics (Basel) 2020;9(12):863. doi: 10.3390/antibiotics9120863. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 168.Saakre M., Mathew D., Ravisankar V. Perspectives on plant flavonoid quercetin-based drugs for novel SARS-CoV-2, Beni. Suef. Univ. J. Basic. Appl. Sci. 2021;10(1):21. doi: 10.1186/s43088-021-00107-w. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 169.Li Z., CaoY H., Cheng, et al. Inhibition of porcine epidemic diarrhea virus replication and viral 3C-like protease by quercetin. Int. J. Mol. Sci. 2020;21(21):8095. doi: 10.3390/ijms21218095. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 170.Kushwaha P.P., Singh A.K., Prajapati K.S., et al. Phytochemicals present in Indian ginseng possess potential to inhibit SARS-CoV-2 virulence: a molecular docking and MD simulation study. Microb. Pathog. 2021;157 doi: 10.1016/j.micpath.2021.104954. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 171.Bhati S., Kaushik V., Singh J. Rational design of flavonoid based potential inhibitors targeting SARS-CoV 3CL protease for the treatment of COVID-19. J. Mol. Struct. 2021;1237 doi: 10.1016/j.molstruc.2021.130380. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 172.Alrasheid A.A., Babiker M.Y., Awad T.A. Evaluation of certain medicinal plants compounds as new potential inhibitors of novel corona virus (COVID-19) using molecular docking analysis. Silico. Pharmacol. 2021;9(1):10. doi: 10.1007/s40203-020-00073-8. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 173.Kandeel M., Abdelrahman A.H.M., Oh-Hashi K., et al. Repurposing of FDA-approved antivirals, antibiotics, anthelmintics, antioxidants, and cell protectives against SARS-CoV-2 papain-like protease. J. Biomol. Struct. Dyn. 2021;39(14):5129–5136. doi: 10.1080/07391102.2020.1784291. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 174.Chikhale R.V., Gurav S.S., Patil R.B., et al. SARS-CoV-2 host entry and replication inhibitors from Indian ginseng: an in-silico approach. J. Biomol. Struct. Dyn. 2021;39(12):4510–4521. doi: 10.1080/07391102.2020.1778539. [DOI] [PMC free article] [PubMed] [Google Scholar]
- 175.Tatar G., Salmanli M., Dogru Y., et al. Evaluation of the effects of chlorhexidine and several flavonoids as antiviral purposes on SARS-CoV-2 main protease: molecular docking, molecular dynamics simulation studies. J. Biomol. Struct. Dyn. 2022;40(17):7656–7665. doi: 10.1080/07391102.2021.1900919. [DOI] [PubMed] [Google Scholar]
Associated Data
This section collects any data citations, data availability statements, or supplementary materials included in this article.
Data Availability Statement
Not applicable.