



Abstract
The pan-eukaryotic protein kinase GCN2 (General Control Nonderepressible2) regulates the translation of mRNAs in response to external and metabolic conditions. Although GCN2 and its substrate, translation initiation factor 2 (eIF2) α, and several partner proteins are substantially conserved in plants, this kinase has assumed novel functions in plants, including in innate immunity and retrograde signaling between the chloroplast and cytosol. How exactly some of the biochemical paradigms of the GCN2 system have diverged in the green plant lineage is only partially resolved. Specifically, conflicting data underscore and cast doubt on whether GCN2 regulates amino acid biosynthesis; also whether phosphorylation of eIF2α can in fact repress global translation or activate mRNA specific translation via upstream open reading frames; and whether GCN2 is controlled in vivo by the level of uncharged tRNA. This review examines the status of research on the eIF2α kinase, GCN2, its function in the response to xenobiotics, pathogens, and abiotic stress conditions, and its rather tenuous role in the translational control of mRNAs.
Keywords: translation initiation, amino acids, tRNA, reactive oxygen, innate immunity, ribosome stalling
1. Introduction
The translation apparatus synthesizes every protein in every cell. Engaging mRNAs and tRNAs, amino acids, ribosomes, and numerous accessory translation factors, protein synthesis consumes a substantial portion of cellular energy and locks up rate-limiting nutrients, especially significant proportions of phosphate and nitrogen. A regulatory network referred to as ‘translational control’ ensures that the rate of protein synthesis is fine-tuned in global, i.e., transcriptome-wide, and mRNA-specific ways. Translational control of specific mRNAs helps to ensure that functionally related proteins are made at rates that optimize the efficiency of metabolic pathways and stoichiometry of protein complexes; excess capacity should be avoided. Beyond individual mRNAs, translation is repressed across the entire transcriptome under a variety of environmental conditions that challenge protein synthesis because of bottlenecks in energy charge (e.g., darkness and hypoxia) and protein folding (e.g., heat stress) [1, 2].
During translation initiation a cytosolic mRNA is joined by the small (40S) ribosomal subunit, which then scans along the 5’ untranslated ‘leader’ of the mRNA, recognizes the AUG start codon, and is joined by the large (60S) ribosomal subunit. The initiation phase is the key target of translational control, because it mainly determines the rate of synthesis for individual proteins over time scales of more than a few minutes, i.e., the ribosome transit time on an mRNA. At first approximation, regulating translation elongation or termination will not affect the rate with which an encoded protein is completed, except for a transient blip, unless elongation comes to a complete halt. Slowing elongation will however raise the density of ribosomes on the mRNA and thus increase the fraction of cellular ribosomes that are engaged in translation. Because the total number of ribosomes in the cell is finite, this may eventually push the translation apparatus to the point where the number of free ribosomes becomes rate limiting for initiation [3, 4].
Among the plethora of the eukaryotic translation initiation factors (eIFs), eIF2 occupies a key position. EIF2 is a trimeric GTPase that carries the initiator methionyl-tRNA to the 40S ribosome. Across fungi, plants, and animals, global protein synthesis is repressed by kinases that phosphorylate the α subunit of eIF2 under a variety of stress conditions on a highly conserved serine residue (Ser 51 in mammals and budding yeast, Ser 52 in fission yeast, Ser 56 in Arabidopsis) [5]. In yeast and animals, translational repression ensues because P-eIF2α inhibits the GDP-GTP exchange factor (GEF) for eIF2, a rate-limiting decameric protein complex called eIF2B [6–8]. In plants it is evident that conditions leading to P-eIF2α generally repress translation, but the biochemical significance of eIF2α phosphorylation, specifically whether P-eIF2α inhibits eIF2B, remains unresolved, as discussed below.
2. The GCN2 signaling system
2.1. The eIF2α kinase GCN2
Plants and budding yeast (Saccharomyces cerevisiae) possess only one kinase that phosphorylates eIF2α on the critical serine 56 residue, GCN2 (General Control Nonderepressible2), whereas fission yeast and animals have additional eIF2α kinases [5, 9, 10]. The universally conserved features of GCN2 are; (i) a central serine-threonine kinase domain; (ii) a carboxyl-terminal domain with similarity to histidyl-tRNA synthetase (HisRS-like); and (iii) an amino-terminal RWD domain that facilitates the interaction of GCN2 with a partner protein, GCN1 [11–13] in complex with GCN20 [14]. The potentially regulatory pseudokinase domain found in fungal and animal GCN2 [15, 16] is absent in plant GCN2 (Fig. 1A).
Figure 1.

(A) Domain architecture of GCN2. At, Arabidopsis thaliana; Sc, Saccharomyces cerevisiae; Hs, Homo sapiens; Dm, Drosophila melanogaster; Ce, Caenorhabditis elegans. Numbers denote amino acid positions. RWD, a domain common in Ring-finger and WD40-domain proteins and yeast DEAD (DEXD)-like helicases; interacts with GCN1. Linker (+/−), Region with mostly charged amino acids (Arg, Lys, Gln and Asp) found between the RWD and pseudokinase domain. Pseudokinase (ΨPK), a domain similar to the eIF2α kinase domain that lacks crucial residues for catalytic activity and may function as a regulatory domain. EIF2α kinase, catalyzes the phosphorylation of eIF2α; double asterisks (**) symbols denote two conserved threonine autophosphorylation sites within the activation sub-domain. HisRS, histidinyl-tRNA synthetase (HisRS)-like domain. CTD, carboxy-terminal domain, functions in dimerization and ribosome-binding and together with the HisRS-like domain, inhibits kinase activity in yeast [105]. The m2 motif (pink rectangle) within the HisRS domain is a conserved YR dipeptide motif required for tRNA binding [19]. Also shown (*) is the TOR kinase phosphorylation site at Serine (Ser) 577 in ScGCN2, which is not conserved in AtGCN2. The amino acid coordinates of the individual domains are assigned based on [15, 22, 72, 106, 107] and NCBI protein domain prediction. CTD for DmGCN2 and CeGCN2 is predicted based on the presence of amino acids at the C-terminal region corresponding to the ScGCN2. AtGCN2 does not have any amino acids beyond the HisRS domain. (B) Model for the activation of ScGCN2. In non-starved yeast cells, interactions between the CTD, HisRS and kinase domains of each monomer keep GCN2 in an enzymatically inactive antiparallel dimer. Consequently, eIF2 continues to support translation initiation by metabolizing GTP and supplying the initiator tRNAMet to the 40S ribosome. Upon amino acid starvation, uncharged tRNA accumulates, which is bound by the HisRS domain of GCN2, evoking a conformational change, thereby allowing the kinase domain to dimerize in the active back-to-back conformation. This structural rearrangement, in combination with the interactions of the RWD domain with GCN1/GCN20, allows the kinase domain to bind and phosphorylate eIF2α, resulting in suppression of translation initiation. Adapted and modified from [50,105]. One of the monomers of the GCN2 dimer is shown in transparent background for simplicity. PKN and PKc are the N- and C-terminal lobe of the kinase domain respectively.
2.2. General amino acid control by Gcn2 in yeast
In S. cerevisiae, deficit in a single amino acid triggers a general increase in all amino acid biosynthesis [17]. This response is known as the general amino acid control (GAAC), which is regulated in part by the cis-acting regulatory elements such as the 5’-TGACTC-3’ sequence found in the upstream regions of many genes under GAAC (e.g., His1, His3, His4) [18]. The other regulatory module of GAAC is composed of two general types of trans-acting genes, the general control derepressed (GCD) genes that function as negative regulators and general control nonderepressible (GCN) genes that are positive regulators of the GAAC. Thus, in a yeast gcn mutant, amino acid starvation does not induce the general amino acid biosynthesis, hence “nonderepressible”. Consequently, gcn mutants fail to grow in the presence of amino acid biosynthesis inhibitors.
The molecular events involving regulation of GAAC are tightly linked with the process of translation initiation and formation of P-eIF2α (Fig. 1B). In detail, the HisRS-like domain inhibits Gcn2’s kinase activity when amino acids are plentiful. Gcn2 becomes activated when a shortage of amino acids raises the levels of uncharged tRNA, which in turn binds to the aaRS domain and relieves its autoinhibitory function [19, 20]. This triggers autophosphorylation of the kinase on two critical threonine residues and activates the kinase to phosphorylate eIF2α [15, 16, 21–23]. Although the HisRS-like domain is most similar to the histidyl tRNA synthetase, it binds multiple uncharged tRNAs [19, 21, 24].
The phosphorylation of eIF2α represses translation because yeast P-eIF2α binds to and inhibits its guanine nucleotide exchange factor, eIF2B [8]. As more of eIF2B is inhibited, the rate at which eIF2’s spent GDP gets exchanged with fresh GTP declines resulting in less eIF2 available to deliver methionyl-tRNA to the 40S subunit. This causes a global decline in translation initiation. More mRNAs remain untranslated and fewer ribosomes are engaged on polysomes. However, a small subset of mRNAs become translated under conditions of amino acid starvation, when eIF2α is phosphorylated *reviewed in 25–26]. Specifically, the Gcn4 mRNA codes for a bZip transcription factor that activates the expression of amino acid biosynthesis genes [5, 26]. The inverse translational control of Gcn4 is achieved by virtue of two upstream open reading frames (uORFs), short coding sequences in the 5’ leader of the Gcn4 mRNA that form a ‘lure and trap’ system. The combined action of uORF #1 (the lure) and uORF #2 (the trap) under amino acid replete or starvation conditions represses or activates the translation of Gcn4 mRNA, respectively. In a gcn2 mutant background, the system assumes the amino acid replete state, eIF2α remains unphosphorylated, and therefore Gcn4 translation remains repressed. Thus, in a gcn2 mutant, the general amino acid control is “non-derepressible” (GCN). Similar sets of lure-and-trap uORFs mediate the translational induction of yeast Gcn4 and vertebrate ATF4, a bZip transcription factor driving a variety of stress responses [reviewed in 26, 27] (for details see Fig. 2).
Figure 2.
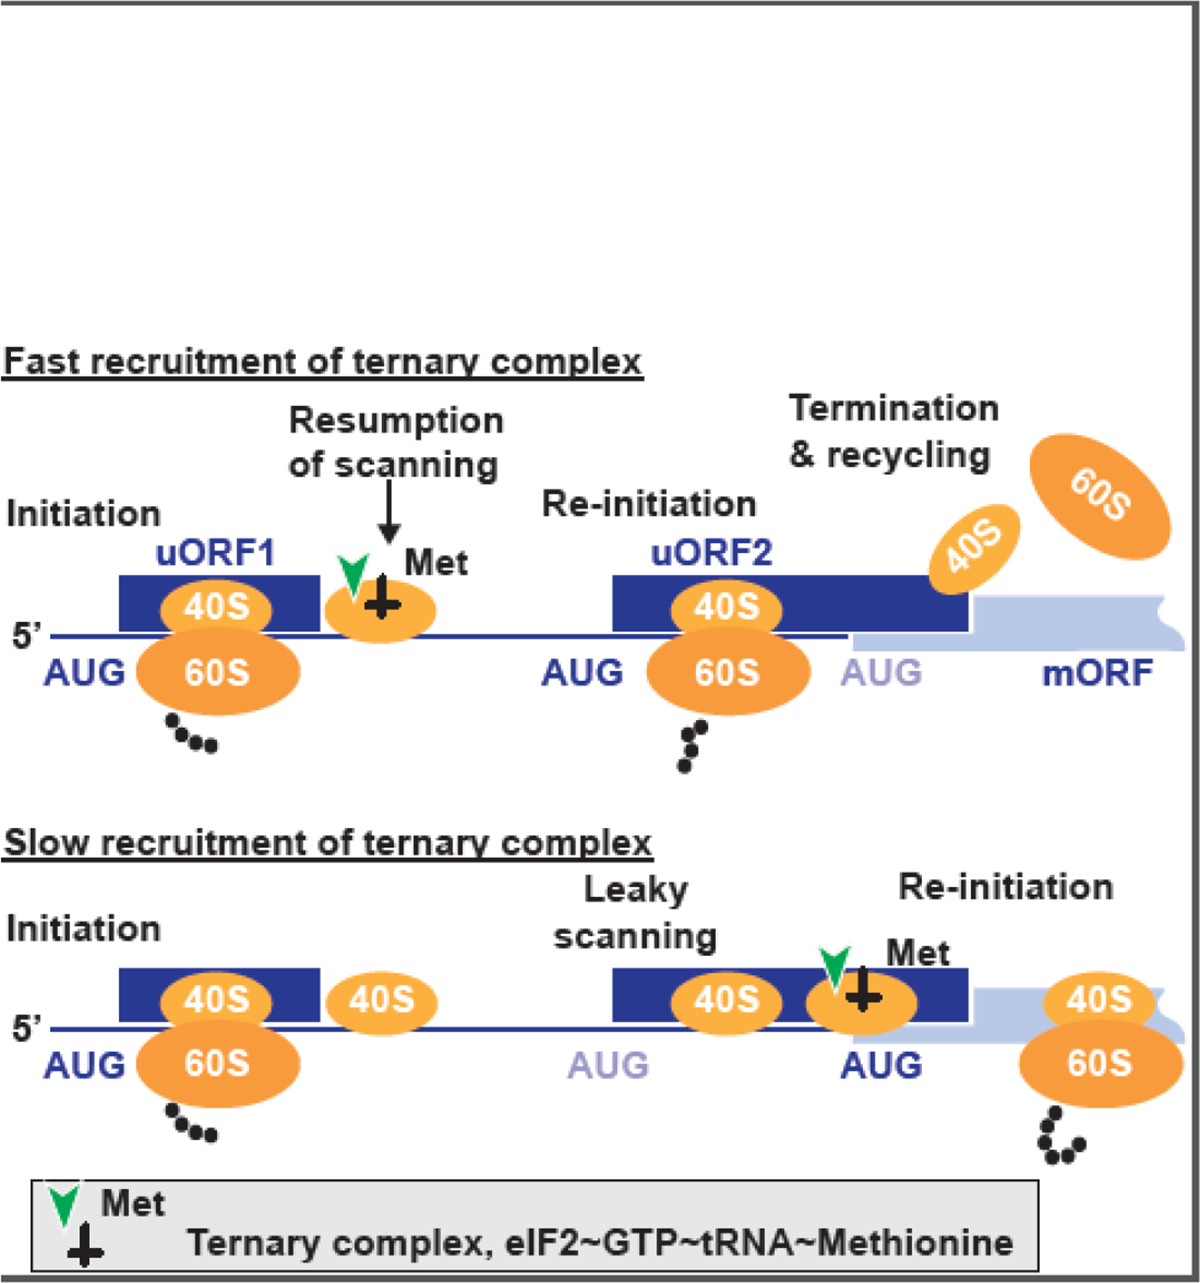
Translational regulation of the mammalian ATF4 mRNA by availability of active ternary complex (eIF2~GTP~Methionyl-tRNA). Under normal conditions, when active eIF2~GTP is plentiful, the ribosome that resumes scanning after having translated uORF1 (the ‘lure’), quickly acquires a fresh ternary complex, and therefore translates uORF2 (the ‘trap’). Because uORF2 overlaps the main ATF4 mORF, the ribosome bypasses that ATF4 AUG codon by leaky scanning and ATF4 is not translated. Under stress conditions, when ternary complex is in low abundance because of phosphorylation by eIF2 kinases, the ribosome that resumes scanning after uORF1 bypasses the uORF2 AUG before acquiring a fresh ternary complex. This allows the main ORF to be translated (after [26, 108]).
2.3. uORFs that sense the level of eIF2 have not been described in plants
In plants, there is yet no solid evidence for an mRNA with a lure-and-trap uORF system equivalent to GCN4 and ATF4. In Arabidopsis, the tendency for ribosomes to resume scanning after terminating on a uORF is generally deemed high and declines with the length of the uORF [28], and uORFs that overlap the mORF’s AUG definitely abrogate translation (e.g., [29]). Thus, the sequence determinants necessary for the lure-and-trap system can be built. However, there are no experimental data to demonstrate that the tendency for ribosomes to reinitiate can be titrated by the level of active eIF2α, or, more specifically, by the phosphorylation status of eIF2α. Some data show that the translation of the TBF1 transcription factor mRNA depends on GCN2 in Arabidopsis [30], but this observation has been disputed elsewhere [31]. Two bZip transcription factors, the maize regulator of seed storage protein expression Opaque-2 as well as Arabidopsis bZip11 have also been suggested as uORF-containing, translationally regulated mRNAs analogous to yeast Gcn4 and mammalian ATF4 [32]. However, it has not been shown that these or other uORF systems form a lure and trap system as for Gcn4 and ATF4. The yeast Gcn4 leader sequence and its uORFs do not seem to function in an equivalent manner in plants [29]. When Arabidopsis GCN2 was activated and eIF2α phosphorylated, a few mRNAs appeared insensitive or even translationally induced, but these mRNAs did not have a uORF arrangement resembling the ATF4 lure-and-trap system [33]. Thus, how Arabidopsis uses uORFs, P-eIF2α, and GCN2 to induce translation of specific mRNAs warrants further study.
3. GCN2 and the Integrated Stress Response
While budding yeast and plants have only a single eIF2α kinase (Gcn2), vertebrates and fission yeast possess up to three additional eIF2α kinases. PERK kinase is activated by misfolded proteins in the endoplasmic reticulum; heme regulated inhibitor (HRI) is activated by heme shortage, and protein kinase R (PKR) is activated by double-stranded RNA, together constituting the integrated stress response (ISR) (Fig. 3). In plant genomes no kinases equivalent to PERK, HRI and PKR have been discovered. In Arabidopsis a kinase activity with properties similar to PKR was characterized [34], but since no PKR-like sequence was found in the sequenced plant genomes, the origin of the PKR-like activity is unclear.
Figure 3.

GCN2 mediated translational repression is part of the integrated stress response in fungi, mammals and plants. MV, methyl viologen. For details see text.
In Arabidopsis as well as in yeast, the GCN2 kinase alone responds to multiple stress conditions, thus forming the basis for an integrated stress response. Notably, in every case tested, any phosphorylation of eIF2α that was observed was absent in null mutants of GCN2 kinase, supporting that GCN2 is the only eIF2α kinase in Arabidopsis. Given the very low or undetectable phosphorylation of eIF2α under control conditions, and given that the transcriptome of the gcn2 mutant is nearly identical to wild type [33], GCN2 kinase activity appears to be largely inactive in the absence of stress.
4. Conservation of structure and function of plant GCN2 with other eukaryotes
Many structural elements of the GCN2 signaling system and some of its functions are generally conserved between yeast, plants and other organisms. Plant GCN2 has a similar domain architecture as yeast GCN2, although the pseudokinase domain is not recognizable and the extreme carboxyl-terminal domain is absent (Fig. 1A) [13, 35, 36]. The kinase domain of tobacco GCN2 alone is active in phosphorylating eIF2α [37], and Arabidopsis GCN2 binds uncharged tRNA [38]. What has not been shown as yet is to what degree plant GCN2 is auto-inhibited by its HisRS-like domain and derepressed by tRNA. However, Arabidopsis GCN2 can functionally complement a yeast gcn2 mutation [13], including the translational control by amino acid starvation, suggesting functional conservation of the major regulatory principle. Moreover, wheat eIF2α can functionally complement a yeast eIF2α mutation including the translational induction of GCN4. This implies that plant eIF2α can trimerize with the yeast eIF2β and γ subunits, and the chimeric complex can dock on and block yeast’s eIF2B GEF activity [39].
However, several important elements of the yeast and mammalian GCN2 signaling paradigm have yet to be discovered in plants, leaving open the possibility that biochemical functions have diverged since the last common ancestor of plant and non-plant lineages. All five subunits of eIF2B are conserved in the Arabidopsis genome, and eIF2B exists as a protein complex [40]; however, neither the biochemical activity nor the genetic role of plant eIF2B are well understood. First, it is questionable whether plant eIF2 requires eIF2B as a GEF at all, because the affinity of plant eIF2 for GDP in vitro is only 10-fold higher than for GTP [41], which should allow for spontaneous GDP-GTP exchange [42–44], wheat eIF2 did not bind GDP as tightly as rabbit eIF2 did, and rabbit eIF2B did not catalyze GDP-GTP exchange on wheat eIF2 [43]. Second, P-eIF2α barely repressed translation in the wheat germ in vitro translation system [43, 45], and expression of phospho-mimic and phospho-deficient versions of eIF2α had only minor effects on total ribosome loading in a live plant transient expression system. Moreover, the phosphorylated form of eIF2α cofractionated with the 40S subunit and with a 48S preinitiation complex [45]. Third, even though plant eIF2 was able to substitute for eIF2 in yeast [39], plant eIF2α exposed to eIF2-kinase did not bind well to rabbit eIF2B and did not work as well as endogenous rabbit eIF2 to inhibit translation [42]. Thus, there is as yet no clear evidence from in vitro studies that phosphorylation of plant eIF2α inhibits translation in plants.
As our understanding of plant GCN2 lags behind that of yeast and animals, many details remain unknown, for example, whether plant GCN2 has additional direct substrates besides eIF2α as was recently discovered in yeast [46]; whether GCN2 is phosphorylated by or regulates the TOR kinase [47, 48], which is also emerging as a regulator of amino acid signaling in plants [49]; whether GCN2 dimerizes under physiological conditions [50–53], associates with ribosomes [50, 54, 55] and is activated by the 60S P-stalk [56, 57].
5. Is plant GCN2 regulated by amino acid starvation?
In budding yeast Gcn2 is activated by multiple isoforms of uncharged tRNA [19, 21], and Gcn2 induces the transcriptional regulon known as the general amino acid control by inducing the translation of the cognate transcription factor, Gcn4. This regulation by amino acids and tRNA also occurs in vertebrates [58–60] (Fig. 2, 3). Likewise, in the fungus Neurospora crassa, where eIF2α phosphorylation peaks during the day and falls during the night, the rhythm of P-eIF2α is due to an underlying cycle of uncharged tRNA that activates the N. crassa GCN2 homolog, CPC-3 [61]. Thus, GCN2 is widely involved in communicating the cell’s amino acid status to the translation apparatus.
5.1. Evidence implicating plant GCN2 in amino acid control
Certain pieces of evidence suggest that a role for GCN2 in amino acid signaling is conserved in plants. For example, Arabidopsis GCN2 is activated by inhibitors and by certain mutations that affect amino acid biosynthesis and by certain inhibitors of aminoacyl tRNA synthetase [35, 36, 62–64]. However, other evidence paints a more complex picture, suggesting that the role of GCN2 in amino acid control has diverged in the plant lineage. GCN2 in plants is activated by a wide variety of stresses, many of which seem unlikely to affect amino acid levels or tRNA charging over the short time scale needed to activate the kinase (see Supplemental Table 1), for example UV light, cold temperature, and reactive oxygen species (ROS) [33, 35, 65, 66]. There is also little evidence as yet that activation of GCN2 triggers a gene expression program intended to rectify a shortage in amino acids. The key question remains. Does the conventional model of GCN2 activation via uncharged tRNAs that accumulate due to amino acid starvation apply to plant GCN2?
The most widely observed evidence for GCN2 having a role in amino acid sensing is that the kinase is activated rapidly when amino acid biosynthesis is inhibited. Arabidopsis GCN2 is reliably activated in planta within as little as 30 minutes [33] by numerous herbicides that target various amino acid biosynthesis pathways, such as chlorosulfuron (targets branched chain amino acids) [33, 35, 36, 67]; sulfonylurea (branched chain amino acids) [68]; glyphosate (aromatic amino acids) [33, 36, 69]; glufosinate (glutamine) [33], or IRL1803 and histidinol (histidine) [35, 36] (Fig. 4). Importantly, by supplementing the plants with the missing amino acid, the GCN2-dependent phosphorylation of eIF2α is substantially suppressed, alongside the chlorosis of the herbicide treated seedlings [36, 68]. In addition, growth of gcn2 mutant seedlings is more sensitive than wild type when exposed to herbicides, which is also reversed by addition of the appropriate amino acid [36] (see Supplemental Table 2 for a list of growth phenotypes).
Figure 4.
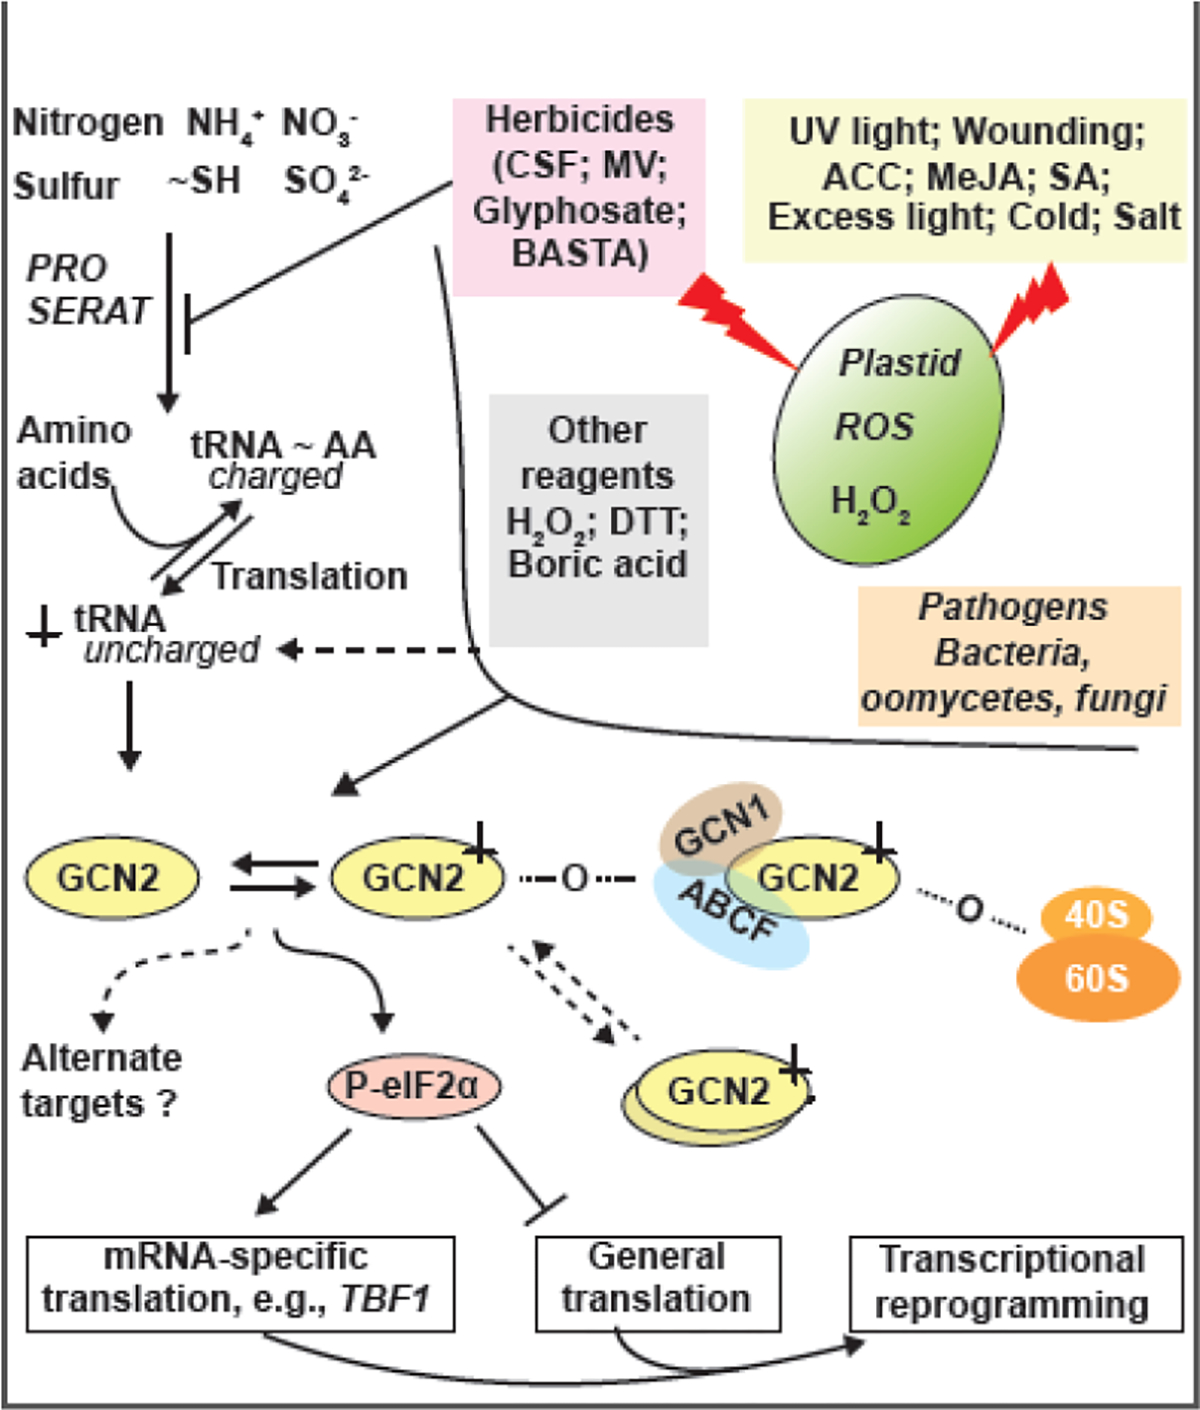
The GCN signaling network. GCN2 is activated by uncharged tRNA as well as by other signals that may or may not work through uncharged tRNA. The signals include pathogens and associated signaling molecules (the ethylene precursor ACC, salicylic acid [SA] and methyl jasmonate [MeJA]), xenobiotic agents (e.g., chlorosulfuron [CSF], glufosinate ammonium [BASTA], methyl viologen [MV]), dithiothreitol [DTT]), and abiotic stresses (e.g., ultraviolet light). Some of these triggers are known to affect the plastid reactive oxygen (ROS) levels (e.g., excess light, salt, cold, and some herbicides) which may directly or indirectly activate the cytosolic GCN2. GCN2 phosphorylates eIF2α but may potentially have other targets. The kinase activity of GCN2 requires a cofactor, GCN1, which functions with the ATP binding cassette protein ABCF3, known as Gcn20 in yeast and SCORD5 in Arabidopsis [95]. Many of the signals that activate GCN2 also repress translation and may do so through GCN2-dependent (shown) or independent channels (not shown). PRO and SERAT represent genes for amino acid biosynthetic enzymes. 40S and 60S denote the plant cytosolic ribosomal subunits. Single arrows denote influences; double arrows denote equilibria; ---o--- denotes physical interactions; stippled arrows denote events that lack direct evidence in plants.
Additional evidence that GCN2 is sensitive to amino acid status comes from mutants. GCN2 is activated in a maize mutant deficient in proline biosynthesis [64] as well as in the serat mutant of Arabidopsis, which has a defect in O-acetyl-serine (OAS) and cysteine biosynthesis [62]. Of note, GCN2 is not activated under sulfate deprivation nor in the sulfate assimilation mutant sir1; this even though sir1 is also defective in amino acid homeostasis [58]. The gcn2 mutants have increased autophagy activity, and the phosphorylation of eIF2α after herbicide treatment is accelerated in autophagy mutants [68]. These results are in keeping with a role of GCN2 in amino acid sensing.
In support of the notion that GCN2 is activated by uncharged tRNA, GCN2 becomes active when the aspartyl-tRNA synthetase is inhibited by the defense priming agent beta-aminobutyric acid (BABA) [63]. Moreover, the growth inhibition caused by BABA is mediated by GCN2; and the protection by BABA against oomycete attack does not work in the gcn2 mutant [63]. These data suggest that GCN2 can be regulated by uncharged tRNAs.
Finally, direct evidence for GCN2’s role in regulating amino acids comes from overexpression experiments in wheat, which yielded lower amino acid levels in the grains, with asparagine reduced the most, as well as varied changes in gene expression of amino acid biosynthesis genes and elevated expression of nitrate reductase [70].
5.2. Evidence that GCN2 may not function as a sensor of amino acid status
However, several other pieces of evidence paint a more complex picture. First, herbicides activate GCN2 very rapidly, well within 30 minutes. Does herbicide deplete amino acids and affect tRNA charging on such a short time frame? In fact, in the duckweed Lemna, chlorosulfuron treatment resulted in a significant increase in the free pools of several amino acids (e.g., Asn, Asp, Gln, Glu, Ser, Met, Pro) within 24 hours, while the proportion of branched chain amino acids, targeted by chlorosulfuron, declined [71]. Moreover, when one amino acid becomes rate limiting for translation, theoretically only its cognate tRNA(s) should become uncharged, while all other tRNAs may even become hypercharged because translation is stalled, thus working to reduce rather than increase the ligand that activates GCN2. In yeast there is evidence that depletion of one amino acid can rapidly affect the levels of this and other amino acids, and can lower the acylation of not only its cognate tRNA but also of certain other tRNAs [24]. However, these changes are sometimes transient, and thus the paradox remains: Why would an increase in deacylation of one or a few tRNAs be sufficient to activate GCN2 given that GCN2 apparently binds multiple tRNAs? Why is GCN2 inactive under unstressed conditions even though an easily detectable fraction of the tRNA pool is normally deacylated? Clearly, we need data on the charging status of tRNAs depending on GCN2 activation status.
More caveats regarding the role of amino acids and uncharged tRNA for regulation of GCN2 come from the observation that many of the most rapid activators of the kinase are not inhibitors of amino acid synthesis, for example UV light [35, 66] and the trigger of reactive oxygen species, methyl viologen, which causes strong P-eIF2α within 10 minutes [33]. Unfortunately, it remains to be established how rapidly amino acid levels and tRNA charging status are affected under most if not all of these treatments.
Finally, in some contrast to the effect of GCN2 overexpression in wheat [70], the activation of GCN2 by herbicide does not induce a general amino acid response at the translational or transcriptional level, as happens in yeast. In detail, P-eIF2α is detected rapidly (<30min) and polysome loading is reduced within 2 hours, yet neither at 2 hours [33] nor at 6 hours [69] was it evident that GCN2 regulates the adaptation in transcript levels for amino acid biosynthesis genes. Therefore, the conventional model that GCN2 mediates a general amino acid control in Arabidopsis as it does in yeast, is lacking critical evidence.
In this context it may be relevant that fungi often find themselves in environments where amino acids can be absorbed from the extracellular environment, whereas plants routinely produce their own amino acids after assimilating nitrogen from inorganic sources. Thus, it is not far fetched that plants would regulate amino acid synthesis quite differently from yeast and animals.
6. Is plant GCN2 activated by reactive oxygen species?
Oxidative stress is well known to inhibit global translation in all eukaryotes at the stages of initiation or elongation and even by direct damage to the translational apparatus. GCN2 has been implicated in this. In the fission yeast S. pombe, eIF2α is phosphorylated within 1 hour of exposure to 1mM H2O2 by both Hri1 and Gcn2 [72]. Although the eIF2α kinases are not required for the initial translational repression upon oxidative stress, Gcn2 cooperates with ROS-sensitive kinases that regulate elongation [73, 74]. In S. cerevisiae, translation initiation is highly sensitive, with maximal inhibition at 1mM H2O2 within as little as 15 min, a response that was partially but not fully dependent on Gcn2 [75]. Thus, H2O2 appears to inhibit global translation in both Gcn2-dependent and independent ways in S. cerevisiae and S. pombe.
Gcn4 is upregulated in response to oxidative stress and is essential for coordinating responses towards the oxidative stress in yeast [76]. As is the case with other triggers of Gcn2 activity in yeast, Gcn1 and Gcn20 are necessary for this, as is the HisRS domain of Gcn2. Moreover, the stability/activity of aminoacyl-tRNA synthetases are known to be affected by ROS [77]. Together, these data have bolstered the view that ROS activates Gcn2 via the classical uncharged tRNAdeacyl pathway. However, it is also plausible that ScGcn2 may be a direct target of ROS.
In photosynthesizing plants, chloroplasts account for the majority of ROS production [78–82]. In Arabidopsis, exposure to sudden high-light (excess light) activates GCN2 and triggers eIF2α phosphorylation. This effect is likely mediated by ROS from the chloroplast because it can be ameliorated by inhibitors of photosynthetic electron transport, and because antioxidants inhibit the light-activation of GCN2 [33]. Moreover, methyl viologen, a potent herbicide that targets ferredoxin resulting in rapid and massive production of superoxide and H2O2, also activates GCN2, as does 10mM H2O2, the latter even in darkness [33].
Other abiotic stress conditions such as salinity and cold stress also result in rapid ROS production and GCN2 activation [33, 65]. Under these conditions, the GCN2 appears to confer an adaptive benefit given that Arabidopsis gcn2 mutant seedlings show growth defects and/or reduced survival in response to high light, salt, and cold stress [33, 65], as previously observed under herbicide stress [36]. That said, other conditions that are known to trigger ROS accumulation such as heat stress, hypoxia, and ER stress did not activate GCN2 under dark as judged by P-eIF2α, suggesting light as a requirement for GCN2 activation by xenobiotic and abiotic stresses [33, 35] (Fig. 4). These observations indicate that GCN2 gets activated under conditions of high ROS pressure, not unlike the situation in fungi, which in plants is much more likely to occur when photosynthesis is active.
What remains unclear is whether ROS activates the kinase activity of GCN2 via uncharged tRNA. On this note it is relevant that the ROS effects were detected in dark adapted Arabidopsis seedlings, i.e., when global translation is already at a basal state [33]. Interestingly, exposure to an extended night of as little as two hours and beyond in Arabidopsis rosettes triggers a gradual and pronounced increase in most free amino acid pools including branched chain amino acids, aromatic amino acids, asparagine and arginine [83,84], which, together with depressed polysome loading, implies a downward pressure on the respective uncharged tRNAs. Lokdarshi and coworkers proposed that even the classical activation of GCN2 by inhibitors of amino acid synthesis, such as chlorosulfuron and glufosinate, may be mediated via ROS, because they induce rapid accumulation of ROS [33, 85], their effect on GCN2 is light- and photosynthesis-dependent, and their action may precede the depletion of amino acid pools.
Altogether, Arabidopsis GCN2 responds to ROS as is the case in yeasts; ROS may even be the unifying signal that explains how diverse environmental conditions can induce GCN2 rapidly. Because the chloroplast plays a key role, this signaling scheme qualifies as a retrograde pathway from the chloroplast to cytosolic translation [86]. What remains to be uncovered are the biochemical mechanisms by which the chloroplastic ROS activate the cytosolic GCN2 and the specific nature of mRNAs that fall under GCN2 control in plants.
7. Is plant GCN2 a sensor of microbial pathogens?
A variety of evidence suggests that plant GCN2 plays a role in innate immunity. For plants, nitrogen and the amino acids made from it are nearly always a rate limiting commodity. Plant pathogens draw on this very same amino acid pool. Thus, it is not implausible that the GCN2 system of the plant lineage, being sensitive to uncharged tRNAs, may be functioning less as an amino acid sensor but more as a sensor of pathogens. Evidence in favor of this comes from the following.
In Arabidopsis, the GCN2 is activated by salicylic acid [35, 43, 87], the key trigger of systemic acquired resistance, as well as by wounding, and methyl-jasmonate, a systemic signaling molecule in the defense against wounding and necrotrophic microbes [35] as well as by feeding damage from the whitefly [88]. More specifically, GCN2 responds to diverse microbe-associated molecular patterns, which are often applied to prime defense responses in an experimental setting; chitin [89], a cell wall component of fungi; the elf18 peptide [31], which is a peptide derived from the highly conserved prokaryotic elongation factor Tu; and the xenobiotic priming agent beta-amino butyric acid (BABA) [63]. Accordingly, GCN2 is activated within one hour by the bacterial pathogen Pseudomonas syringae [30, 90], although other investigators did not observe this [67]. In contrast, inoculation with two RNA viruses did not result in P-eIF2α [36]. Infection of Nicotiana benthamiana with tobacco mosaic virus was accompanied by P-eIF2α, and the virulence was even influenced by the phosphorylation potential of eIF2α, but the role of GCN2 in this model system was not addressed [91]. Thus, while the innate antiviral defense response of animals relies heavily on P-eIF2α (Fig. 3) via protein kinase R, this has not been observed for GCN2 in plants.
7.1. GCN2 mediates innate immunity
Given that GCN2 is activated by bacterial pathogen, various priming agents, and endogenous plant defense signals, it might be expected that GCN2 supports plant innate immunity. Indeed, gcn2 mutants are more susceptible to a variety of pathogens. Silencing of GCN2 in barley enhanced the susceptibility to the fungus Blumeria [92], whereas mutants of gcn2 in Arabidopsis are more susceptible to the necrotrophic fungus Botrytis cinerea [89]. Given that Pseudomonas could trigger P-eIF2α by GCN2, one may expect that mutants might be more susceptible to this bacterium, but the results are varied. Some investigators have seen gcn2 mutants to be less (not more) susceptible to Pseudomonas [30], while others saw no difference [31, 67].
These contrasting results might possibly be explained by the experimental conditions, specifically whether the host plants had experienced any priming agents or not prior to challenge with the pathogen. However, although GCN2 is activated by priming agents, the role of GCN2 in the priming response also varies. Consistent with a pro-defense role of GCN2 specifically in priming, the gcn2 mutant did not defend itself as well as wild type after priming by chitin [33], although surprisingly priming with flg22 peptide and with elf18 peptide or BABA, both of which also induce GCN2, were still effective in gcn2 mutants [31, 33, 63]. Thus, GCN2 is not universally needed for priming the defense response and the reason for the disparate susceptibilities of gcn2 mutants in the Pseudomonas challenge assays remains unclear.
Another possible explanation comes from careful observations that consider the time course of the interaction between the Arabidopsis host and the Pseudomonas pathogen. In the early ‘pre-invasion’ phase, wild-type GCN2 actually promotes resistance via stomata closing as ABA signaling genes are upregulated [30]. Over the course of infection, Pseudomonas employs an effector molecule, coronatine, to force stomata open, but this effect is GCN2-dependent and thus absent in gcn2. At the post-invasive stage (18h), GCN2 promotes elevated ABA levels, and this is accompanied by increased virulence and growth of Pseudomonas. Thus, GCN2 appears to have defense-promoting effects, preferentially early in infection, and virulence-promoting effects, preferentially later in infection [30]. Accordingly, infection assays with the fungus Golovinomyces cichoracearum, the oomycete Hyaloperonospora arabidopsidis and the necrotroph Pectobacterium carotovorum revealed that the gcn2 mutant was more susceptible early on in infection but less susceptible over the long term [93].
Overall, the seemingly contradictory findings regarding the role of GCN2 in plant defense can be reconciled with two arguments. First, GCN2 is activated by microbe associated molecular patterns and affects a fundamental cellular process, translation, where hundreds of mRNAs are affected in slightly different ways [33]. Even if GCN2 affected translation of mRNAs uniformly, the fact that some mRNAs promote defense while others promote virulence will on balance give rise to a situation where subtle differences in the inoculation conditions may tip the scales towards defense or disease in unpredictable ways. Second, the plant defense response plays out in stages over time, and early and late events most likely depend on GCN2 activity to different degrees.
On this note, it is opportune to consider here that GCN2 also plays seemingly contradictory roles after abiotic stress. As expected, gcn2 mutants are more sensitive than wild type to certain stresses, for example herbicides, continuous high light, cold and salt at the seedling stage [33,35,36,65]. However, interestingly, under other stress conditions, gcn2 mutants are resistant! Resistance is most evident when gcn2 mutants are exposed to the translation inhibitor paromomycin [67]. The gcn2 mutant is also slightly resistant to glyphosate spray at the rosette stage [69] and UV light [66], and is less prone to senescence than wild type in the cold [87]. One way to rationalize these results is by considering that GCN2 likely represses translation globally when activated, a rather invasive cellular event. Under those stresses where gcn2 is resistant, the large cost inflicted by the repression may outweigh the benefit from GCN2’s mitigating effects, whereas under other stresses the cost-benefit balance is positive.
7.2. What do we know about GCN2’s mechanism of action in plant defense?
To better understand the role of GCN2 in plant defense, the precise mechanism of GCN2 action needs to be clarified. As mentioned earlier, the biochemical consequence of eIF2α phosphorylation, the primary output of GCN2, is still not understood in plants. The mRNA for the defense-related transcription factor TBF1 is the best-investigated link between GCN2 and pathogens [30]. Infection with Pseudomonas [30, 90] or with elf18 peptide [31] can boost TBF1 translation via two upstream ORFs (uORFs) [90] and a purine rich ‘R-motif’ [31]. The 2nd uORF is longer than the first and appears to be inhibitory to translation, which is not surprising. But while some data suggest that GCN2 regulates TBF1 translation by Pseudomonas [30], others claim that GCN2 is not involved when TBF1 translation is stimulated by elf18 peptide [31]. In any event, a mechanism whereby GCN2 would influence how ribosomes navigate the TBF1 uORFs, as has been elaborated for yeast Gcn4 and mammalian ATF4 (Fig. 2), is not clear in the case of Arabidopsis TBF1. The effects of GCN2 on defense may be mediated in part through TBF1, but plausibly also other translational and non-translational targets.
Are GCN1 and GCN20, which are cofactors for GCN2, implicated in these pathogen responses? Severe alleles and to some degree a mild allele of gcn1 allow more growth of Pseudomonas syringae bacteria than wild type [94]. In addition, mutants of gcn1 and gcn20 are both hypersensitive to Pseudomonas syringae DC3000 in similar ways, even under conditions where gcn2 was not involved [67, 95]. Thus, all three GCN genes appear to play a role in plant defense, but their phenotypes are sufficiently distinct that one can conclude they do not always function coordinately.
In summary there is much circumstantial evidence that GCN2 contributes to plant defense and disease, but a clear molecular pathway remains to be established. It would be tempting to apply the yeast paradigm of Gcn2-mediated translational repression onto the plant priming and defense responses, but this paradigm is not at all self-evident. This paradigm predicts that pathogen or MAMP activates GCN2; this is indeed often the case. It also predicts that MAMPs cause global translational reorganization. Chitin and elf18 both appear to do so, but this was not shown to be GCN2 dependent [31, 89]. In contrast, BABA priming agent has an effect on plant growth that is GCN2-dependent, but it has not been shown that the effect is due to inhibition of translation [63]. The paradigm also predicts that certain mRNAs escape the translational inhibition with the help of uORFs, and this has been demonstrated for TBF1 [30, 31, 90], but whether GCN2 is necessary for this remains to be seen.
8. What is the role of GCN2-mediated P-eIF2α in translational control?
8.1. GCN2 and global translation
In Arabidopsis, the translation factor eIF2α gets phosphorylated under numerous stress conditions. In each case examined so far, the GCN2 has been found to be responsible for this. However, as mentioned earlier, the biochemical consequence of P-eIF2α on the plant translation apparatus is unclear. If indeed activation of GCN2 leads to translational repression, then one would expect that (i) conditions that activate GCN2 would also repress translation, and (ii) under these conditions, translation would remain active in the gcn2 mutant and /or the gcn1 mutant, which is also defective in P-eIF2α [67]. Data conforming to (i) and (ii) were shown early on when treatments with chlorosulfuron and 8-aza-adenine, which activate GCN2, repressed translation or polysome loading in wild type, but less so in the gcn2 mutant [35, 87].
However, other reports have shown that GCN2 activity, as scored by P-eIF2α, and translational repression are not well correlated. And when a particular treatment represses translation, it is often not GCN2-dependent. For example, Izquierdo and coworkers identified four different treatments that all activated GCN2 as per P-eIF2α, but the translational repression (amino acid incorporation) being observed varied and was either independent of GCN2 and GCN1, or required GCN1 but not GCN2 [67]. Likewise, treatment with hydrogen peroxide, which activated GCN2, caused a drop in mRNA-ribosome loading, but this drop was not GCN2-dependent [33]. Vice versa, two mutations that affect the two upstream branches of cysteine biosynthesis activated GCN2 to different extent, but caused similar defects in amino acid incorporation [62]. These observations suggest that the primary effect of such treatments on translation is mediated by a separate mechanism, perhaps involving GCN1, and that GCN2 plays more of an accessory role. This idea has recently earned credence in the case of the translational repression by reactive oxygen in fission yeast and mammalian cells [74].
Lastly, the potential role of P-eIF2α in the formation of stress granules is of particular interest, because the ISR in general and P-eIF2α specifically have been firmly implicated in stress granule formation in animals in some cases, though not always [96]. In Arabidopsis, heat stress, darkness, hypoxia and ER stress all trigger stress granules [97–99]. However, with the exception of dithiothreitol [67], an inducer of ER stress, none of these conditions triggered phosphorylation of eIF2α [33, 35, 43, 100]. In contrast, conditions not known to cause stress granules in plants such as UV, ROS, and inhibitors of amino acid biosynthesis, reliably induce P-eIF2α. Therefore, evidence that GCN2 and P-eIF2α are required for stress granule formation is lacking in plants.
8.2. GCN2 and mRNA-specific translation
Does GCN2’s primary role perhaps lie in mRNA-specific translation? A transcriptome-wide analysis of polysome loading in response to chlorosulfuron revealed differences in the translatome profile between wild type and gcn2 mutants. However, this experiment did not uncover the much sought-after equivalent of the yeast Gcn4 and vertebrate ATF4 mRNAs. Instead, mRNAs whose polysome loading was protected by GCN2 were not clearly enriched for functional categories and did not have a distinguishing sequence feature such as uORFs [33].
Challenging Arabidopsis with pathogen will boost the translation of the mRNA for transcription factor TBF1. This effect is mediated by uORFs in TBF1’s 5’ mRNA leader sequence [31, 90], and GCN2 may be required for its maximal translation [30]. However, the arrangement of the TBF1 uORFs is not easily compatible with the well established and detailed molecular model for GCN2- and eIF2α-mediated derepression of yeast Gcn4 and mammalian ATF4. How TBF1 gets translationally activated under pathogen challenge and the possible role of GCN2 remain to be clarified.
In summary, both the potential roles of GCN2 in repressing cytosolic translation, and its potential role in modulating translation in a sequence specific manner deserve continued attention.
9. Does GCN2 work with GCN1 and GCN20 to respond to ribosome collisions or ribosome stalling?
In yeast and mammalian cells, GCN2 is co-activated by two cofactors, the essential, large HEAT-repeat protein, GCN1, and the F-type ATP-binding cassette protein, GCN20, both of which associate with the ribosome [12, 46, 54].
There is genetic and biochemical evidence that GCN1 functions as cofactor of GCN2 in plants as well. Most importantly, gcn1 mutants cannot phosphorylate eIF2α, just like gcn2 mutants [53, 67, 87]. Second, plant GCN1 and GCN2 can interact in the yeast two hybrid system [67] and through GCN1’s C-terminal domain [53]. Third, mutations in gcn1 and mutations in gcn2 both render plants sensitive to cold [65, 87] and both gcn1 and gcn2 mutants are resistant to the antibiotic paromomycin [67], which is best known for its ability to cause tRNA decoding errors. However, GCN1 must play additional roles beyond activating GCN2, because the mutant phenotypes of gcn2 and gcn1 overlap only partially in a complex manner. The gcn1 mutants are chlorotic dwarfs [67, 87, 101] with defects in thylakoid membrane development [53] while gcn2 mutants grow normally under favorable conditions. Also, sensitivity to antimycin A and boric acid is seen in gcn1 but not in gcn2 mutants [67].
The role of ABCF3/GCN20 in the functions of GCN1 and GCN2 is less clear. Gcn20 mutants share many characteristics with gcn1 mutants, such as chlorosis [95], a common transcriptome profile, altered responses to ABA and the herbicide paraquat [102], similarly reduced protein synthesis, similar sensitivity to antimycin A, boric acid, and infection with Pseudomonas [67]. Although ABCF3 is but one of five highly similar genes in Arabidopsis, ABCF3 appears to have a unique role that is closely linked with GCN1. Surprisingly, ABCF3/GCN20 is not required for GCN2’s kinase activity as judged by P-eIF2α and abcf3/gcn20 is also not resistant to paromomycin, the way gcn2 and gcn1 are [67]. Taken together, ABCF3/GCN20 is linked to GCN2 function primarily as a cofactor of GCN1.
Recently it was discovered that in S. cerevisiae, GCN1 senses ribosome collisions (disomes) that occur after one ribosome has become stalled or slowed down sufficiently for the next ribosome to catch up on the mRNA. Structurally, the extended HEAT repeats of GCN1 allow it to bridge the collided ribosomes, and the ribosome collision activates GCN2 [103–104]. This can happen rapidly because GCN2 is already bound to the ribosome [54, 104], specifically the P-stalk of the 60S, which can activate mammalian GCN2 in the absence of uncharged tRNA [56].
In plants we have as yet no direct evidence for a role of GCN1, GCN2 or GCN20 in sensing ribosome collisions. However, this hypothesis could potentially reconcile several findings laid out in this review.
Diverse treatments including UV light, reactive oxygen, cold temperature, and inhibitors of amino acid synthesis all activate GCN2, but it is not immediately evident how all these conditions would rapidly lower the tRNA charging status. However, these conditions can quite plausibly inhibit the progression of a ribosome in a stochastic manner by protein-RNA crosslinking, misfolding of the nascent polypeptide, or slowing down the ribosome. The ribosome collision hypothesis would unify these disparate observations.
The considerations discussed in section 5.2 have been difficult to reconcile with the idea that GCN2 is controlled primarily by the cellular concentration of uncharged tRNA. If a separate signal, such as ribosome collision sensed by GCN1, were the primary trigger for GCN2, uncharged tRNA may function more as a cofactor rather than the primary regulator of GCN2.
Taken together, the information available at this time leaves open the possibility that plant GCN1-GCN2 sense ribosome collisions, also. Meanwhile, given that the phenotypes of gcn1 and gcn2 mutants overlap only partially, GCN1 and GCN2 may each have roles independent of each other.
Conclusions
The eIF2α kinase GCN2 is highly conserved between plants and other eukaryotes, and many inferences about GCN2 as a translational regulator from animals and yeast may hold true in plants as well. Investigators have been puzzled by the fact that mutants in this highly conserved kinase that allegedly represses translation have no visible phenotype under natural growth conditions; but this has changed. There are now striking phenotypes including growth defects under cold and salt stress, altered pathogen responses to many pathogens, lack of priming against oomycetes, resistance to paromomycin, sensitivity as well as resistance to herbicide, and synthetic phenotypes with autophagy. It also appears that the plant lineage has evolved a different paradigm for GCN2, a conclusion most evident from the fact that P-eIF2α is often uncoupled from translational repression. Key questions for future work include the following. What is the biochemical trigger that activates GCN2, and does it involve amino acid starvation or ribosome collisions? Does phosphorylation of eIF2α by GCN2 indeed inhibit translation, and how? Does GCN2 have activities besides eIF2α phosphorylation? How does GCN2 contribute to the translational reorganization that is commonly observed when GCN2 gets activated? And how can this knowledge be harnessed to improve the adaptation of crop plants to stress conditions? The research tools are at hand to answer these questions in the coming years.
Supplementary Material
Supplemental Table 1. A table listing comprehensively all conditions and publications under which GCN2-dependent phosphorylation of eIF2alpha was observed.
Supplemental Table 2. A table listing growth phenotypes of gcn2 mutants.
Highlights.
Activation of the GCN2 kinase is often accompanied by translational repression, but whether and how the kinase causes repression in plants is not clear
GCN2 operates together with one obligatory cofactor, GCN1, and one nonessential cofactor, an ATP-binding cassette protein
GCN2 kinase alone integrates a wide variety of stresses, qualifying it as the regulator of the ‘integrated stress response’ in plants
The role of plant GCN2 in direct amino acid sensing remains controversial, especially as reactive oxygen or ribosome collisions may have additional roles in activating plant GCN2.
Acknowledgements
We thank the members of the von Arnim lab, Ricardo Andres Urquidi Camacho, Anwesha Dasgupta and Mark Edens, for discussion.
Funding
The preparation of this article was supported by NIH grant 2R15GM129672–02 to AGvA. Beyond providing financial support, the funder was not involved in conceptualizing the article, collecting and interpreting the information, writing of the article or deciding to submit the article.
Abbreviations
- ABC
ATP-binding cassette
- bZIP
basic leucine zipper
- CTD
carboxy-terminal domain
- eIF
eukaryotic translation initiation factor
- GAAC
general amino acid control
- GCD
general control derepressed
- GCN
general control nonderepressible
- GEF
GDP-GTP exchange factor
- HEAT repeat
repeat motif found in huntingtin, elongation factor 3, phosphatase 2A and TOR kinase
- HisRS
Histidyl-tRNA synthetase
- HRI
heme regulated inhibitor
- ISR
integrated stress response
- PKR
protein kinase R
- ROS
reactive oxygen species
- uORF
upstream open reading frame
Footnotes
Declaration of Competing Interest
The authors report no competing interests.
Declaration of Competing Interest
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
Publisher's Disclaimer: This is a PDF file of an unedited manuscript that has been accepted for publication. As a service to our customers we are providing this early version of the manuscript. The manuscript will undergo copyediting, typesetting, and review of the resulting proof before it is published in its final form. Please note that during the production process errors may be discovered which could affect the content, and all legal disclaimers that apply to the journal pertain.
References
- [1].Merchante C, Stepanova AN, Alonso JM, Translation regulation in plants: an interesting past, an exciting present and a promising future, Plant J, 90 (2017) 628–653. [DOI] [PubMed] [Google Scholar]
- [2].Urquidi Camacho RA, Lokdarshi A, von Arnim AG, Translational gene regulation in plants: A green new deal, Wiley Interdiscip Rev RNA, (2020) e1597. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [3].Zur H, Tuller T, Predictive biophysical modeling and understanding of the dynamics of mRNA translation and its evolution, Nucleic Acids Research, 44 (2016) 9031–9049. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [4].Levin D, Tuller T, Whole cell biophysical modeling of codon-tRNA competition reveals novel insights related to translation dynamics, PLoS Comput Biol, 16 (2020) e1008038. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [5].Wek RC, Role of eIF2alpha Kinases in Translational Control and Adaptation to Cellular Stress, Cold Spring Harb Perspect Biol, 10 (2018). pii: cshperspect.a032870. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [6].Adomavicius T, Guaita M, Zhou Y, Jennings MD, Latif Z, Roseman AM, Pavitt GD, The structural basis of translational control by eIF2 phosphorylation, Nature Communications, 10 (2019) 2136. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [7].Gordiyenko Y, Llácer JL, Ramakrishnan V, Structural basis for the inhibition of translation through eIF2α phosphorylation, Nature Communications, 10 (2019) 2640. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [8].Krishnamoorthy T, Pavitt GD, Zhang F, Dever TE, Hinnebusch AG, Tight binding of the phosphorylated alpha subunit of initiation factor 2 (eIF2alpha) to the regulatory subunits of guanine nucleotide exchange factor eIF2B is required for inhibition of translation initiation, Mol Cell Biol, 21 (2001) 5018–5030. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [9].Muñoz A, Castellano MM, Regulation of Translation Initiation under Abiotic Stress Conditions in Plants: Is It a Conserved or Not so Conserved Process among Eukaryotes?, Comp Funct Genomics, 2012 (2012) 406357. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [10].Taniuchi S, Miyake M, Tsugawa K, Oyadomari M, Oyadomari S, Integrated stress response of vertebrates is regulated by four eIF2α kinases, Scientific Reports, 6 (2016) 32886. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [11].Kubota H, Sakaki Y, Ito T, GI Domain-mediated Association of the Eukaryotic Initiation Factor 2α Kinase GCN2 with Its Activator GCN1 Is Required for General Amino Acid Control in Budding Yeast, Journal of Biological Chemistry, 275 (2000) 20243–20246. [DOI] [PubMed] [Google Scholar]
- [12].Castilho BA, Shanmugam R, Silva RC, Ramesh R, Himme BM, Sattlegger E, Keeping the eIF2 alpha kinase Gcn2 in check, Biochim Biophys Acta, 1843 (2014) 1948–1968. [DOI] [PubMed] [Google Scholar]
- [13].Zhang Y, Dickinson JR, Paul MJ, Halford NG, Molecular cloning of an arabidopsis homologue of GCN2, a protein kinase involved in co-ordinated response to amino acid starvation, Planta, 217 (2003) 668–675. [DOI] [PubMed] [Google Scholar]
- [14].Garcia-Barrio M, Dong J, Ufano S, Hinnebusch AG, Association of GCN1–GCN20 regulatory complex with the N-terminus of eIF2α kinase GCN2 is required for GCN2 activation, The EMBO Journal, 19 (2000) 1887–1899. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [15].Lageix S, Rothenburg S, Dever TE, Hinnebusch AG, Enhanced interaction between pseudokinase and kinase domains in Gcn2 stimulates eIF2α phosphorylation in starved cells, PLoS Genet, 10 (2014) e1004326. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [16].Maia de Oliveira T, Korboukh V, Caswell S, Winter Holt JJ, Lamb M, Hird AW, Overman R, The structure of human GCN2 reveals a parallel, back-to-back kinase dimer with a plastic DFG activation loop motif, Biochem J, 477 (2020) 275–284. [DOI] [PubMed] [Google Scholar]
- [17].Hinnebusch AG, Mechanisms of gene regulation in the general control of amino acid biosynthesis in Saccharomyces cerevisiae, Microbiol Rev, 52 (1988) 248–273. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [18].Hinnebusch AG, Fink GR, Repeated DNA sequences upstream from HIS1 also occur at several other co-regulated genes in Saccharomyces cerevisiae, J Biol Chem, 258 (1983) 5238–5247. [PubMed] [Google Scholar]
- [19].Wek SA, Zhu S, Wek RC, The histidyl-tRNA synthetase-related sequence in the eIF-2 alpha protein kinase GCN2 interacts with tRNA and is required for activation in response to starvation for different amino acids, Mol Cell Biol, 15 (1995) 4497–4506. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [20].Zhu S, Sobolev AY, Wek RC, Histidyl-tRNA synthetase-related sequences in GCN2 protein kinase regulate in vitro phosphorylation of eIF-2, J Biol Chem, 271 (1996) 24989–24994. [DOI] [PubMed] [Google Scholar]
- [21].Dong J, Qiu H, Garcia-Barrio M, Anderson J, Hinnebusch AG, Uncharged tRNA activates GCN2 by displacing the protein kinase moiety from a bipartite tRNA-binding domain, Mol Cell, 6 (2000) 269–279. [DOI] [PubMed] [Google Scholar]
- [22].Padyana AK, Qiu H, Roll-Mecak A, Hinnebusch AG, Burley SK, Structural basis for autoinhibition and mutational activation of eukaryotic initiation factor 2alpha protein kinase GCN2, J Biol Chem, 280 (2005) 29289–29299. [DOI] [PubMed] [Google Scholar]
- [23].Qiu H, Hu C, Dong J, Hinnebusch AG, Mutations that bypass tRNA binding activate the intrinsically defective kinase domain in GCN2, Genes & Development, 16 (2002) 1271–1280. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [24].Zaborske JM, Narasimhan J, Jiang L, Wek SA, Dittmar KA, Freimoser F, Pan T, Wek RC, Genome-wide analysis of tRNA charging and activation of the eIF2 kinase Gcn2p, J Biol Chem, 284 (2009) 25254–25267. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [25].Young SK, Wek RC, Upstream Open Reading Frames Differentially Regulate Gene-specific Translation in the Integrated Stress Response, J Biol Chem, 291 (2016) 16927–16935. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [26].Gunišová S, Hronová V, Mohammad MP, Hinnebusch AG, Valášek LS, Please do not recycle! Translation reinitiation in microbes and higher eukaryotes, FEMS Microbiology Reviews, 42 (2017) 165–192. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [27].Pavitt GD, Ron D, New insights into translational regulation in the endoplasmic reticulum unfolded protein response, Cold Spring Harb Perspect Biol, 4 (2012) a012278. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [28].von Arnim AG, Jia Q, Vaughn JN, Regulation of plant translation by upstream open reading frames, Plant Sci, 214 (2014) 1–12. [DOI] [PubMed] [Google Scholar]
- [29].Roy B, Vaughn JN, Kim BH, Zhou F, Gilchrist MA, von Arnim AG, The h subunit of eIF3 promotes reinitiation competence during translation of mRNAs harboring upstream open reading frames, RNA, 16 (2010) 748–761. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [30].Liu X, Afrin T, Pajerowska-Mukhtar KM, Arabidopsis GCN2 kinase contributes to ABA homeostasis and stomatal immunity, Commun Biol, 2 (2019) 302. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [31].Xu G, Greene GH, Yoo H, Liu L, Marqués J, Motley J, Dong X, Global translational reprogramming is a fundamental layer of immune regulation in plants, Nature, 545 (2017) 487–490. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [32].Lam H-M, Chiao YA, Li M-W, Yung Y, Ji S, Putative Nitrogen Sensing Systems in Higher Plants, Journal of Integrative Plant Biology, 48 (2006) 873–888. [Google Scholar]
- [33].Lokdarshi A, Guan J, Urquidi Camacho RA, Cho SK, Morgan PW, Leonard M, Shimono M, Day B, von Arnim AG, Light Activates the Translational Regulatory Kinase GCN2 via Reactive Oxygen Species Emanating from the Chloroplast, The Plant Cell, 32 (2020) 1161–1178. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [34].Chang LY, Yang WY, Browning K, Roth D, Specific in vitro phosphorylation of plant eIF2 alpha by eukaryotic eIF2 alpha kinases, Plant Molecular Biology, 41 (1999) 363–370. [DOI] [PubMed] [Google Scholar]
- [35].Lageix S, Lanet E, Pouch-Pelissier MN, Espagnol MC, Robaglia C, Deragon JM, Pelissier T, Arabidopsis eIF2alpha kinase GCN2 is essential for growth in stress conditions and is activated by wounding, BMC Plant Biol, 8 (2008) 134. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [36].Zhang Y, Wang Y, Kanyuka K, Parry MA, Powers SJ, Halford NG, GCN2-dependent phosphorylation of eukaryotic translation initiation factor-2alpha in Arabidopsis, Journal of experimental botany, 59 (2008) 3131–3141. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [37].Hao YC, Yang YX, Zhang SJ, Li YB, Zhai CH, Long Y, Jia HF, Zhang ST, Expression, purification, and in vitro characterization of kinase domain of NtGCN2 from tobacco, Protein Expression and Purification, 163 (2019) 105452. [DOI] [PubMed] [Google Scholar]
- [38].Li MW, AuYeung WK, Lam HM, The GCN2 homologue in Arabidopsis thaliana interacts with uncharged tRNA and uses Arabidopsis eIF2 alpha molecules as direct substrates, Plant Biology, 15 (2013) 13–18. [DOI] [PubMed] [Google Scholar]
- [39].Chang LY, Yang WY, Roth D, Functional complementation by wheat elF2 alpha in the yeast GCN2-mediated pathway, Biochemical and Biophysical Research Communications, 279 (2000) 468–474. [DOI] [PubMed] [Google Scholar]
- [40].McWhite CD, Papoulas O, Drew K, Cox RM, June V, Dong OX, Kwon T, Wan C, Salmi ML, Roux SJ, Browning KS, Chen ZJ, Ronald PC, Marcotte EM, A Pan-plant Protein Complex Map Reveals Deep Conservation and Novel Assemblies, Cell, 181 (2020) 460–474.e414. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [41].Shaikhin SM, Smailov SK, Lee AV, Kozhanov EV, Iskakov BK, Interaction of wheat germ translation initiation factor 2 with GDP and GTP, Biochimie, 74 (1992) 447–454. [DOI] [PubMed] [Google Scholar]
- [42].Krishna VM, Janaki N, Ramaiah KV, Wheat germ initiation factor 2 (WG x eIF2) decreases the inhibition in protein synthesis and eIF2B activity of reticulocyte lysates mediated by eIF2alpha phosphorylation, Arch Biochem Biophys, 346 (1997) 28–36. [DOI] [PubMed] [Google Scholar]
- [43].Zhigailov AV, Alexandrova AM, Nizkorodova AS, Stanbekova GE, Kryldakov RV, Karpova OV, Polimbetova NS, Halford NG, Iskakov BK, Evidence That Phosphorylation of the α-Subunit of eIF2 Does Not Essentially Inhibit mRNA Translation in Wheat Germ Cell-Free System, Frontiers in plant science, 11 (2020) 936–936. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [44].Immanuel TM, Greenwood DR, MacDiarmid RM, A critical review of translation initiation factor eIF2α kinases in plants - regulating protein synthesis during stress, Funct Plant Biol, 39 (2012) 717–735. [DOI] [PubMed] [Google Scholar]
- [45].Zhigailov AV, Stanbekova GE, Nizkorodova AS, Galiakparov NN, Gritsenko DA, Polimbetova NS, Halford NG, Iskakov B, Phosphorylation of the alpha-subunit of plant eukaryotic initiation factor 2 prevents its association with polysomes but does not considerably suppress protein synthesis. Plant Science 317 (2022) 111190. [DOI] [PubMed] [Google Scholar]
- [46].Dokládal L, Stumpe M, Pillet B, Hu Z, Garcia Osuna GM, Kressler D, Dengjel J, De Virgilio C, Global phosphoproteomics pinpoints uncharted Gcn2-mediated mechanisms of translational control, Mol Cell, 81 (2021) 1879–1889.e1876. [DOI] [PubMed] [Google Scholar]
- [47].Cherkasova VA, Hinnebusch AG, Translational control by TOR and TAP42 through dephosphorylation of eIF2alpha kinase GCN2, Genes Dev, 17 (2003) 859–872. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [48].Yuan W, Guo S, Gao J, Zhong M, Yan G, Wu W, Chao Y, Jiang Y, General Control Nonderepressible 2 (GCN2) Kinase Inhibits Target of Rapamycin Complex 1 in Response to Amino Acid Starvation in Saccharomyces cerevisiae, J Biol Chem, 292 (2017) 2660–2669. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [49].Liu Y, Duan X, Zhao X, Ding W, Wang Y, Xiong Y, Diverse nitrogen signals activate convergent ROP2-TOR signaling in Arabidopsis, Developmental Cell, 56 (2021) 1283–1295.e1285. [DOI] [PubMed] [Google Scholar]
- [50].Qiu H, Garcia-Barrio MT, Hinnebusch AG, Dimerization by translation initiation factor 2 kinase GCN2 is mediated by interactions in the C-terminal ribosome-binding region and the protein kinase domain, Mol Cell Biol, 18 (1998) 2697–2711. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [51].Qiu H, Dong J, Hu C, Francklyn CS, Hinnebusch AG, The tRNA-binding moiety in GCN2 contains a dimerization domain that interacts with the kinase domain and is required for tRNA binding and kinase activation, Embo J, 20 (2001) 1425–1438. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [52].Narasimhan J, Staschke KA, Wek RC, Dimerization is required for activation of eIF2 kinase Gcn2 in response to diverse environmental stress conditions, J Biol Chem, 279 (2004) 22820–22832. [DOI] [PubMed] [Google Scholar]
- [53].Faus I, Niñoles R, Kesari V, Llabata P, Tam E, Nebauer SG, Santiago J, Hauser MT, Gadea J, Arabidopsis ILITHYIA protein is necessary for proper chloroplast biogenesis and root development independent of eIF2α phosphorylation, J Plant Physiol, 224–225 (2018) 173–182. [DOI] [PubMed] [Google Scholar]
- [54].Marton MJ, Vazquez de Aldana CR, Qiu H, Chakraburtty K, Hinnebusch AG, Evidence that GCN1 and GCN20, translational regulators of GCN4, function on elongating ribosomes in activation of eIF2alpha kinase GCN2, Mol Cell Biol, 17 (1997) 4474–4489. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [55].Ramirez M, Wek RC, Hinnebusch AG, Ribosome association of GCN2 protein kinase, a translational activator of the GCN4 gene of Saccharomyces cerevisiae, Mol Cell Biol, 11 (1991) 3027–3036. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [56].Inglis AJ, Masson GR, Shao S, Perisic O, McLaughlin SH, Hegde RS, Williams RL, Activation of GCN2 by the ribosomal P-stalk, Proceedings of the National Academy of Sciences, 116 (2019) 4946–4954. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [57].Masson GR, Towards a model of GCN2 activation, Biochem Soc Trans, 47 (2019) 1481–1488. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [58].Zhang P, McGrath BC, Reinert J, Olsen DS, Lei L, Gill S, Wek SA, Vattem KM, Wek RC, Kimball SR, The GCN2 eIF2αlpha kinase is required for adaptation to amino acid deprivation in mice, Mol Cell Biol, 22 (2002) 6681–6688. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [59].Maurin AC, Jousse C, Averous J, Parry L, Bruhat A, Cherasse Y, Zeng H, Zhang Y, Harding HP, Ron D, Fafournoux P, The GCN2 kinase biases feeding behavior to maintain amino acid homeostasis in omnivores, Cell Metab, 1 (2005) 273–277. [DOI] [PubMed] [Google Scholar]
- [60].Kimball SR, Jefferson LS, Control of protein synthesis by amino acid availability, Curr Opin Clin Nutr Metab Care, 5 (2002) 63–67. [DOI] [PubMed] [Google Scholar]
- [61].Karki S, Castillo K, Ding Z, Kerr O, Lamb TM, Wu C, Sachs MS, Bell-Pedersen D, Circadian clock control of eIF2α phosphorylation is necessary for rhythmic translation initiation, Proceedings of the National Academy of Sciences, 117 (2020) 10935–10945. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [62].Dong YH, Silbermann M, Speiser A, Forieri I, Linster E, Poschet G, Samami AA, Wanatabe M, Sticht C, Teleman AA, Deragon JM, Saito K, Hell R, Wirtz M, Sulfur availability regulates plant growth via glucose-TOR signaling, Nature Communications, 8 (2017) 1174. [DOI] [PMC free article] [PubMed] [Google Scholar] [Retracted]
- [63].Luna E, van Hulten M, Zhang YH, Berkowitz O, Lopez A, Petriacq P, Sellwood MA, Chen BN, Burrell M, van de Meene A, Pieterse CMJ, Flors V, Ton J, Plant perception of beta-aminobutyric acid is mediated by an aspartyl-tRNA synthetase, Nature Chemical Biology, 10 (2014) 450–456. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [64].Wang G, Zhang J, Wang G, Fan X, Sun X, Qin H, Xu N, Zhong M, Qiao Z, Tang Y, Song R, Proline responding1 Plays a Critical Role in Regulating General Protein Synthesis and the Cell Cycle in Maize, Plant Cell, 26 (2014) 2582–2600. [DOI] [PMC free article] [PubMed] [Google Scholar] [Retracted]
- [65].Lokdarshi A, Morgan PW, Franks M, Emert Z, Emanuel C, von Arnim AG, Light-Dependent Activation of the GCN2 Kinase Under Cold and Salt Stress Is Mediated by the Photosynthetic Status of the Chloroplast, Frontiers in Plant Science, 11 (2020) 431. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [66].Llabata P, Richter J, Faus I, Slominska-Durdasiak K, Zeh LH, Gadea J, Hauser MT, Involvement of the eIF2alpha Kinase GCN2 in UV-B Responses, Front Plant Sci, 10 (2019) 1492. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [67].Izquierdo Y, Kulasekaran S, Benito P, Lopez B, Marcos R, Cascon T, Hamberg M, Castresana C, Arabidopsis nonresponding to oxylipins locus NOXY7 encodes a yeast GCN1 homolog that mediates noncanonical translation regulation and stress adaptation, Plant Cell Environ, 41 (2018) 1438–1452. [DOI] [PubMed] [Google Scholar]
- [68].Zhao L, Deng L, Zhang Q, Jing X, Ma M, Yi B, Wen J, Ma C, Tu J, Fu T, Shen J, Autophagy contributes to sulfonylurea herbicide tolerance via GCN2-independent regulation of amino acid homeostasis, Autophagy, 14 (2018) 702–714. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [69].Faus I, Zabalza A, Santiago J, Nebauer SG, Royuela M, Serrano R, Gadea J, Protein kinase GCN2 mediates responses to glyphosate in Arabidopsis, BMC Plant Biol, 15 (2015) 14. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [70].Byrne EH, Prosser I, Muttucumaru N, Curtis TY, Wingler A, Powers S, Halford NG, Overexpression of GCN2-type protein kinase in wheat has profound effects on free amino acid concentration and gene expression, Plant Biotechnology Journal, 10 (2012) 328–340. [DOI] [PubMed] [Google Scholar]
- [71].Rhodes D, Hogan AL, Deal L, Jamieson GC, Haworth P, Amino Acid Metabolism of Lemna minor L. : II. Responses to Chlorsulfuron, Plant Physiol, 84 (1987) 775–780. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [72].Zhan K, Narasimhan J, Wek RC, Differential activation of eIF2 kinases in response to cellular stresses in Schizosaccharomyces pombe, Genetics, 168 (2004) 1867–1875. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [73].Knutsen JH, Rødland GE, Bøe CA, Håland TW, Sunnerhagen P, Grallert B, Boye E, Stress-induced inhibition of translation independently of eIF2α phosphorylation, J Cell Sci, 128 (2015) 4420–4427. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [74].Sanchez M, Lin Y, Yang C-C, McQuary P, Rosa Campos A, Aza Blanc P, Wolf DA, Cross Talk between eIF2α and eEF2 Phosphorylation Pathways Optimizes Translational Arrest in Response to Oxidative Stress, iScience, 20 (2019) 466–480. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [75].Shenton D, Smirnova JB, Selley JN, Carroll K, Hubbard SJ, Pavitt GD, Ashe MP, Grant CM, Global translational responses to oxidative stress impact upon multiple levels of protein synthesis, J Biol Chem, 281 (2006) 29011–29021. [DOI] [PubMed] [Google Scholar]
- [76].Mascarenhas C, Edwards-Ingram LC, Zeef L, Shenton D, Ashe MP, Grant CM, Gcn4 is required for the response to peroxide stress in the yeast Saccharomyces cerevisiae, Mol Biol Cell, 19 (2008) 2995–3007. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [77].Takahashi R, Goto S, Alteration of aminoacyl-tRNA synthetase with age: heat-labilization of the enzyme by oxidative damage, Arch Biochem Biophys, 277 (1990) 228–233. [DOI] [PubMed] [Google Scholar]
- [78].Czarnocka W, Karpioski S, Friend or foe? Reactive oxygen species production, scavenging and signaling in plant response to environmental stresses, Free Radic Biol Med, 122 (2018) 4–20. [DOI] [PubMed] [Google Scholar]
- [79].Schmitt F-J, Renger G, Friedrich T, Kreslavski VD, Zharmukhamedov SK, Los DA, Kuznetsov VV, Allakhverdiev SI, Reactive oxygen species: Re-evaluation of generation, monitoring and role in stress-signaling in phototrophic organisms, Biochimica et Biophysica Acta (BBA) - Bioenergetics, 1837 (2014) 835–848. [DOI] [PubMed] [Google Scholar]
- [80].Lai AG, Doherty CJ, Mueller-Roeber B, Kay SA, Schippers JH, Dijkwel PP, CIRCADIAN CLOCK-ASSOCIATED 1 regulates ROS homeostasis and oxidative stress responses, Proc Natl Acad Sci U S A, 109 (2012) 17129–17134. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [81].Foyer CH, Reactive oxygen species, oxidative signaling and the regulation of photosynthesis, Environmental and Experimental Botany, 154 (2018) 134–142. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [82].Das K, Roychoudhury A, Reactive oxygen species (ROS) and response of antioxidants as ROS-scavengers during environmental stress in plants, Frontiers in Environmental Science, 2 (2014) 53. [Google Scholar]
- [83].Gibon Y, Usadel B, Blaesing OE, Kamlage B, Hoehne M, Trethewey R, Stitt M, Integration of metabolite with transcript and enzyme activity profiling during diurnal cycles in Arabidopsis rosettes, Genome Biol, 7 (2006) R76. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [84].Usadel B, Bläsing OE, Gibon Y, Retzlaff K, Höhne M, Günther M, Stitt M, Global transcript levels respond to small changes of the carbon status during progressive exhaustion of carbohydrates in Arabidopsis rosettes, Plant Physiol, 146 (2008) 1834–1861. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [85].Takano HK, Beffa R, Preston C, Westra P, Dayan FE, Reactive oxygen species trigger the fast action of glufosinate, Planta, 249 (2019) 1837–1849. [DOI] [PubMed] [Google Scholar]
- [86].Dietz KJ, Efficient high light acclimation involves rapid processes at multiple mechanistic levels, Journal of Experimental Botany, 66 (2015) 2401–2414. [DOI] [PubMed] [Google Scholar]
- [87].Wang L, Li H, Zhao C, Li S, Kong L, Wu W, Kong W, Liu Y, Wei Y, Zhu JK, Zhang H, The inhibition of protein translation mediated by AtGCN1 is essential for cold tolerance in Arabidopsis thaliana, Plant Cell Environ, 40 (2017) 56–68. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [88].Li N, Zhang SJ, Zhao Q, Long Y, Guo H, Jia HF, Yang YX, Zhang HY, Ye XF, Zhang ST, Overexpression of Tobacco GCN2 Stimulates Multiple Physiological Changes Associated With Stress Tolerance, Front Plant Sci, 9 (2018) 725. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [89].Berrocal-Lobo M, Toribio R, Castellano MM, eIF2α Phosphorylation by GCN2 Is Induced in the Presence of Chitin and Plays an Important Role in Plant Defense against B. cinerea Infection, Int J Mol Sci, 21 (2020) 7335. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [90].Pajerowska-Mukhtar KM, Wang W, Tada Y, Oka N, Tucker CL, Fonseca JP, Dong X, The HSF-like transcription factor TBF1 is a major molecular switch for plant growth-to-defense transition, Curr Biol, 22 (2012) 103–112. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [91].Bilgin DD, Liu Y, Schiff M, Dinesh-Kumar SP, P58(IPK), a plant ortholog of double-stranded RNA-dependent protein kinase PKR inhibitor, functions in viral pathogenesis, Dev Cell, 4 (2003) 651–661. [DOI] [PubMed] [Google Scholar]
- [92].Ozturk IK, Ersoy F, Akkaya MS, HvGCN2 silencing in barley displays enhanced Blumeria graminis f. sp hordei susceptibility, Archives of Biological Sciences, 70 (2018) 513–520. [Google Scholar]
- [93].Liu X, Merchant A, Rockett KS, McCormack M, Pajerowska-Mukhtar KM, Characterization of Arabidopsis thaliana GCN2 kinase roles in seed germination and plant development, Plant Signal Behav, 10 (2015) e992264. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [94].Monaghan J, Li X, The HEAT repeat protein ILITYHIA is required for plant immunity, Plant Cell Physiol, 51 (2010) 742–753. [DOI] [PubMed] [Google Scholar]
- [95].Zeng WQ, Brutus A, Kremer JM, Withers JC, Gao XL, Jones AD, He SY, A Genetic Screen Reveals Arabidopsis Stomatal and/or Apoplastic Defenses against Pseudomonas syringae pv. tomato DC3000, Plos Pathogens, 7 (2011) e1002291. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [96].Farny NG, Kedersha NL, Silver PA, Metazoan stress granule assembly is mediated by P-eIF2alpha-dependent and -independent mechanisms, RNA, 15 (2009) 1814–1821. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [97].Lokdarshi A, Conner WC, McClintock C, Li T, Roberts DM, Arabidopsis CML38, a Calcium Sensor That Localizes to Ribonucleoprotein Complexes under Hypoxia Stress Plant Physiology, 170 (2015) 1046–1059. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [98].Chantarachot T, Bailey-Serres J, Polysomes, Stress Granules, and Processing Bodies: A Dynamic Triumvirate Controlling Cytoplasmic mRNA Fate and Function, Plant Physiol, 176 (2018) 254–269. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [99].Maruri-López I, Figueroa NE, Hernández-Sánchez IE, Chodasiewicz M, Plant Stress Granules: Trends and Beyond, Frontiers in Plant Science, 12 (2021) 1538. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [100].Kamauchi S, Nakatani H, Nakano C, Urade R, Gene expression in response to endoplasmic reticulum stress in Arabidopsis thaliana, FEBS J, 272 (2005) 3461–3476. [DOI] [PubMed] [Google Scholar]
- [101].Cui X, Gao K, Wang L, Lv M, Li Z, Zheng D, Wu W, Yao W, Ding L, Li X, Zhu J-K, Zhang H, General Control Non-derepressible 1 (AtGCN1) Is Important for Flowering Time, Plant Growth, Seed Development, and the Transcription/Translation of Specific Genes in Arabidopsis, Frontiers in Plant Science, 12 (2021) 239. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [102].Faus I, Niñoles R, Kesari V, Gadea J, The ABCF3 Gene of Arabidopsis Is Functionally Linked with GCN1 but Not with GCN2 During Stress and Development, Plant Molecular Biology Reporter, (2021) 1–10. [Google Scholar]
- [103].Pochopien AA, Beckert B, Kasvandik S, Berninghausen O, Beckmann R, Tenson T, Wilson DN, Structure of Gcn1 bound to stalled and colliding 80S ribosomes, Proceedings of the National Academy of Sciences, 118 (2021) e2022756118. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [104].Yan LL, Zaher HS, Ribosome quality control antagonizes the activation of the integrated stress response on colliding ribosomes, Mol Cell, 81 (2021) 614–628.e614. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [105].Lageix S, Zhang J, Rothenburg S, Hinnebusch AG, Interaction between the tRNA-binding and C-terminal domains of Yeast Gcn2 regulates kinase activity in vivo, PLoS Genet, 11 (2015) e1004991. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [106].He H, Singh I, Wek SA, Dey S, Baird TD, Wek RC, Georgiadis MM, Crystal structures of GCN2 protein kinase C-terminal domains suggest regulatory differences in yeast and mammals, J Biol Chem, 289 (2014) 15023–15034. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [107].Wek RC, Jackson BM, Hinnebusch AG, Juxtaposition of domains homologous to protein kinases and histidyl-tRNA synthetases in GCN2 protein suggests a mechanism for coupling GCN4 expression to amino acid availability, Proc Natl Acad Sci U S A, 86 (1989) 4579–4583. [DOI] [PMC free article] [PubMed] [Google Scholar]
- [108].Harding HP, Novoa I, Zhang Y, Zeng H, Wek R, Schapira M, Ron D, Regulated translation initiation controls stress-induced gene expression in mammalian cells, Mol Cell, 6 (2000) 1099–1108. [DOI] [PubMed] [Google Scholar]
Associated Data
This section collects any data citations, data availability statements, or supplementary materials included in this article.
Supplementary Materials
Supplemental Table 1. A table listing comprehensively all conditions and publications under which GCN2-dependent phosphorylation of eIF2alpha was observed.
Supplemental Table 2. A table listing growth phenotypes of gcn2 mutants.